Synarachnactis lloydii and other burrowing anemones in circalittoral muddy mixed sediment
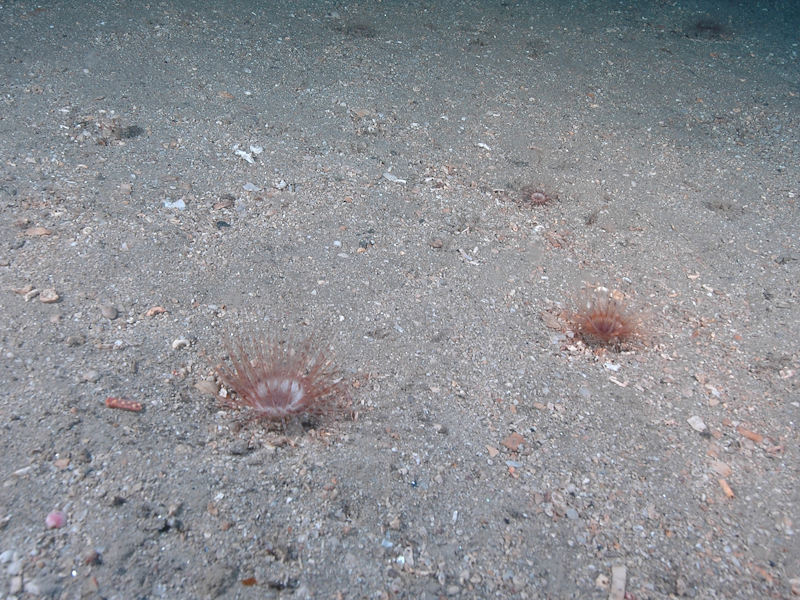
Cerianthus lloydii and other burrowing anemones in circalittoral muddy mixed sediment
Photographer: Dr Keith Hiscock Copyright: Dr Keith Hiscock

Map Key
- Orange points: Core Records
- Pale Blue points: Non-core, certain determination
- Black points: Non-core, uncertain determination
- Yellow areas: Predicted habitat extent
| Researched by | Laura Paling, Amy Watson & Frances Perry | Refereed by | This information is not refereed |
|---|
Summary
UK and Ireland classification
Description
Circalittoral plains of sandy muddy gravel may be characterized by burrowing anemones such as Synarachnactis (syn. Cerinathus) lloydii. Other burrowing anemones such as Cereus pedunculatus, Mesacmaea mitchellii and Aureliania heterocera may be locally abundant. Relatively few conspicuous species are found in any great numbers in this biotope, but they typically include ubiquitous epifauna such as Asterias rubens, Pagurus bernhardus and Polybius depurator with occasional terebellid polychaetes such as Lanice conchilega and the clam Pecten maximus. Ophiura albida may be frequent in some areas, and where surface shell or stones are present, ascidians such as Ascidiella aspersa may occur in low numbers. (Information from Connor et al., 2004; JNCC, 2015, 2022).
Depth range
5-10 m, 10-20 m, 20-30 mAdditional information
-
Sensitivity review
Sensitivity characteristics of the habitat and relevant characteristic species
The plains of sandy muddy gravel within SS.SMx.CMx.ClloMx are relatively sparse in species. This biotope is characterized by burrowing anemones, of which Synarachnactis lloydii (syn. Cerianthus lloydii) is the most abundant species. Other conspicuous species found in this biotope are mobile scavengers and predators, including Callionymus lyra, Pagurus bernhardus and Asterias rubens. Within the sub-biotope SS.SMx.CMx.ClloMx.Nem, the substratum includes more cobbles and pebbles, and the hydroids Nemertesia spp. have a high abundance and are characterizing species for this sub-biotope, in addition to Synarachnactis lloydii. Nemertesia spp., as well as some of the other hydroids, can only attach themselves to a solid substratum, which is why they are missing from SS.SMx.CMx.ClloMx. SS.SMx.CMx.ClloMx.Nem has greater species diversity than SS.SMx.CMx.ClloMx. Therefore, the sensitivity of this biotope is based on the important characterizing species Synarachnactis lloydii. The mobile scavengers probably forage over a greater range than this biotope and are not assessed specifically. The sensitivity of hydroids is mentioned where relevant to SS.SMx.CMx.ClloMx.Nem.
Resilience and recovery rates of habitat
Little evidence was found to support this resilience assessment for Synarachnactis lloydii (syn. Cerianthus lloydii). MES (2010) suggested that the genus Cerianthus would be likely to have a low recovery rate following physical disturbance based on long lifespan and slow growth rate. Ershova et al. (2019) recorded that, in the Chukchi Sea, Cerianthus larvae were found to overlap with the distribution of adults, suggesting that successful recruitment may depend on local reproduction and the retention of larvae near adult populations. No specific evidence was cited to support this conclusion. The MES (2010) review also highlighted that there were gaps in information for this genus and that age at sexual maturity and fecundity are unknown, although the larvae are pelagic (MES 2010). No empirical evidence was found for recovery rates following perturbations for Synarachnactis lloydii. This species has limited horizontal mobility and re-colonization via adults is unlikely (Tillin & Tyler-Walters, 2014).
Hydroids exhibit rapid rates of recovery from disturbance through repair, asexual reproduction, and larval colonization. Sparks (1972) reviewed the regeneration abilities and rapid repair of injuries. Fragmentation of the hydroid provides a route for short-distance dispersal. For example, each fragmented part of Sertularia cupressina can regenerate itself following damage (Berghahn & Offermann, 1999). New colonies of the same genotype may, therefore, arise from damage to existing colonies (Gili & Hughes, 1995). Many hydroid species also produce dormant, resting stages that are very resistant to environmental perturbation (Gili & Hughes, 1995). Colonies can be removed or destroyed; however, the resting stages may survive attached to the substratum and provide a mechanism for rapid recovery (Kosevich & Marfenin, 1986; Cornelius, 1995a). The lifecycle of hydroids typically alternates between an attached solitary or colonial polyp generation and a free-swimming medusa generation. Planulae larvae produced by hydroids typically metamorphose within 24 hours and crawl only a short distance away from the parent plant (Sommer, 1992). Gametes liberated from the medusae (or vestigial sessile medusae) produce gametes that fuse to form zygotes and develop into free-swimming planula larvae (Hayward & Ryland, 1994) and are present in the water column between 2 and 20 days (Sommer, 1992). Rafting on floating debris as dormant stages or reproductive adults (or on ships hulls or in ship ballast water), together with their potentially long lifespan, may have allowed hydroids to disperse over a wide area in the long-term and explain the near cosmopolitan distributions of many hydroid species (Cornelius, 1992; Boero & Bouillon 1993). Hydroids are potential fouling organisms; they rapidly colonizing a range of substrata placed in marine environments and are often the first organisms to colonize available space in settlement experiments (Gili & Hughes, 1995). For example, hydroids were reported to colonize an experimental artificial reef within less than six months, becoming abundant in the following year (Jensen et al., 1994). In similar studies, Obelia spp. recruited to the bases of reef slabs within three months and the slab surfaces within six months of the slabs being placed in the marine environment (Hatcher, 1998). Cornelius (1992) stated that Obelia spp. could form large colonies within a matter of weeks. In a study of the long-term effects of scallop dredging in the Irish Sea, Bradshaw et al. (2002) noted that hydroids increased in abundance, presumably because of their regeneration potential, good local recruitment and ability to colonize newly exposed substrata quickly. Cantero et al. (2002) described the fertility of Obelia dichotoma, Kirchenpaureria pinnata and Nemertesia ramosa in the Mediterranean as being year-round, whilst it should be noted that higher temperatures may play a factor in this year-round fecundity. Bradshaw et al. (2002) observed that reproduction in Nemertesia antennina occurred regularly, with three generations per year. In addition, the presence of adults stimulated larval settlement, so that where adults remained, reproduction was likely to result in local recruitment. Hayward & Ryland (1994) stated that medusae release in Obelia dichotoma occurred in summer.
The hydroids that are present within SS.SMx.CMx.ClloMx.Nem include Halecium halecinum, Nemertesia antennina, and Nemertesia ramosa. Halecium halecinum is an erect hydroid growing up to 25 cm and is found on stones and shells in coastal areas. It is widely distributed in the Atlantic and is present from Svalbard to the Mediterranean (Hayward & Ryland, 1994; Palerud et al., 2004; Medel et al., 1998). Nemertesia anteninna grows up to 25 cm, is found attached to shells and stones on sandy bottoms from the shallow sublittoral into deeper waters offshore, and is recorded in the northeast Atlantic, from at least the Faroes, the Barents Sea and Iceland south through Mauritania to southern Africa, including the Mediterranean, Azores and Madeira. Nemertesia ramosa is a large plumulariid hydroid which grows up to 15 cm, is found inshore to deeper water and is common throughout the British Isles and is distributed from Iceland to north-west Africa (Hayward & Ryland, 1994). In the Azores, for example, it is well known in the sublittoral at 15 to 158 m deep in the central group of islands, but historical records exist from seamounts down to bathyal grounds of nearly 1,000 m (Gomes-Pereira & Tempera, 2016). Nemertesia ramosa is observed in densities of up to 2.82 colonies/m2 on rocky substrate and 0.25 to 0.55 colonies/m2 on mixed bottoms; an aggregated spatial distribution is described, with aggregations being considered hydroid gardens at >0.1 to 0.9 /m2 (Gomes-Pereira & Tempera, 2016). During surveys between 2004 and 2011, colonies of Nemertesia ramosa measured on ROV imagery averaged 23.5 cm in height, with taller colonies (max= 36.7 cm) registered on rocky outcrops protruding more than 15 cm (Gomes-Pereira & Tempera, 2016).
Resilience assessment
The characterizing species of interest are the burrowing anemone Synarachnactis lloydii and the hydroid, Nemertesia antennina. Hydroids, including Nemertesia antennina, are likely to recover from damage very quickly. Based on the available evidence, resilience for the hydroid species assessed is ‘High’ (recovery within two years) for any level of perturbation (where resistance is ‘None’, ‘Low’, ‘Medium’ or ‘High’). Therefore, the ability of both SS.SMx.CMx.ClloMx and SS.SMx.CMx.ClloMx.Nem to recover will depend on the ability of Synarachnactis lloydii to recover. However, there is very little information regarding the resilience of Synarachnactis lloydii. A resilience of ‘Medium’ (2 – 10 years) is suggested for all resistance levels (where resistance is ‘None’, ‘Low’, ‘Medium’) based on expert judgement. Confidence in this assessment is 'Low', due to the lack of direct evidence for the characterizing species.
Note. The resilience and the ability to recover from human-induced pressures are a combination of the environmental conditions of the site, the frequency (repeated disturbances versus a one-off event) and the intensity of the disturbance. Recovery of impacted populations will always be mediated by stochastic events and processes acting over different scales, including, but not limited to, local habitat conditions, further impacts and processes such as larval supply and recruitment between populations. Full recovery is defined as the return to the state of the habitat that existed prior to impact. This does not necessarily mean that every component species has returned to its prior condition, abundance or extent, but that the relevant functional components are present and the habitat is structurally and functionally recognizable as the initial habitat of interest. It should be noted that the recovery rates are only indicative of the recovery potential.
Climate Change Pressures
Use [show more] / [show less] to open/close text displayed
| Resistance | Resilience | Sensitivity | |
Global warming (extreme) [Show more]Global warming (extreme)Extreme emission scenario (by the end of this century 2081-2100) benchmark of:
EvidenceCerianthus lloydii adults are locally abundant in many localities on all coasts of the British Isles and in some areas are common on the shore. This species occurs on all western coasts of Europe from Greenland and Spitzbergen south to the Bay of Biscay. Larvae, but not adults, have been recorded from the Mediterranean (De Kluijver et al., 2024). OBIS (2024) lists records of Cerianthus lloydii from sea surface temperatures of -5 to 20°C, although the majority of records were from 10 to15°C. Similarly, the majority of records for other burrowing anemones (Mesacmaea mitchellii and Cereus pedunclatus) are also between 10 to 15°C. Cerianthus lloydii is predominantly distributed in northern regions, and is likely to move further northward as the climate changes and temperature shifts out of its preferred range. There is no further information available on the temperature tolerance of Cerianthus lloydii. Cerianthids can occur across wide temperature range (8.36 to 11.51°C) and depth ranges from shallow waters to deep-sea environments (238 to 1,070 m). Hydrozoans have been recorded in depths ranging to 8,400 m, indicating adaptations to varied thermal niches throughout the water column (Davies et al., 2014; Stepanjants & Chernyshev, 2015). However, there is limited evidence for thermal thresholds and thermal ranges were available for the characterizing species recorded in this biotope and large knowledge gaps limit current understanding of the ecological feedback that may occur to cerianthids as a result of climate change driven temperature increase. Sensitivity assessment. Under the middle and high emission and extreme scenarios seawater temperatures are expected to temperatures rise by 3 to 5°C to potential southern summer temperatures of 23 to 24°C and northern summer temperatures of 17 to 19°C. The distribution of the important characterizing species Cerianthus lloydii suggest that they are probably resistant of chronic change in temperature for a year, but exposure to a short-term acute increase in temperature may cause Cerianthus lloydii to withdraw into their burrows temporarily. But most records of Cerianthus lloydii occur north of the Bay of Biscay so there is the possibility that it may be driven north or the greater depth to avoid ongoing climate mediated temperature increases. Therefore, for all three scenarios (middle and high emission and extreme scenarios) resistance is assessed as ‘Medium’ as a precaution. Resilience is assessed as ‘Very Low’ due to the long-term nature of ocean warming. This biotope is assessed as ‘Medium’ sensitivity to ocean warming under all three scenarios. However, there is limited evidence on thermal tolerances of the characterizing species recorded in this biotope and confidence in the assessment is ‘Low’. | MediumHelp | Very LowHelp | MediumHelp |
Global warming (high) [Show more]Global warming (high)High emission scenario (by the end of this century 2081-2100) benchmark of:
EvidenceCerianthus lloydii adults are locally abundant in many localities on all coasts of the British Isles and in some areas are common on the shore. This species occurs on all western coasts of Europe from Greenland and Spitzbergen south to the Bay of Biscay. Larvae, but not adults, have been recorded from the Mediterranean (De Kluijver et al., 2024). OBIS (2024) lists records of Cerianthus lloydii from sea surface temperatures of -5 to 20°C, although the majority of records were from 10 to15°C. Similarly, the majority of records for other burrowing anemones (Mesacmaea mitchellii and Cereus pedunclatus) are also between 10 to 15°C. Cerianthus lloydii is predominantly distributed in northern regions, and is likely to move further northward as the climate changes and temperature shifts out of its preferred range. There is no further information available on the temperature tolerance of Cerianthus lloydii. Cerianthids can occur across wide temperature range (8.36 to 11.51°C) and depth ranges from shallow waters to deep-sea environments (238 to 1,070 m). Hydrozoans have been recorded in depths ranging to 8,400 m, indicating adaptations to varied thermal niches throughout the water column (Davies et al., 2014; Stepanjants & Chernyshev, 2015). However, there is limited evidence for thermal thresholds and thermal ranges were available for the characterizing species recorded in this biotope and large knowledge gaps limit current understanding of the ecological feedback that may occur to cerianthids as a result of climate change driven temperature increase. Sensitivity assessment. Under the middle and high emission and extreme scenarios seawater temperatures are expected to temperatures rise by 3 to 5°C to potential southern summer temperatures of 23 to 24°C and northern summer temperatures of 17 to 19°C. The distribution of the important characterizing species Cerianthus lloydii suggest that they are probably resistant of chronic change in temperature for a year, but exposure to a short-term acute increase in temperature may cause Cerianthus lloydii to withdraw into their burrows temporarily. But most records of Cerianthus lloydii occur north of the Bay of Biscay so there is the possibility that it may be driven north or the greater depth to avoid ongoing climate mediated temperature increases. Therefore, for all three scenarios (middle and high emission and extreme scenarios) resistance is assessed as ‘Medium’ as a precaution. Resilience is assessed as ‘Very Low’ due to the long-term nature of ocean warming. This biotope is assessed as ‘Medium’ sensitivity to ocean warming under all three scenarios. However, there is limited evidence on thermal tolerances of the characterizing species recorded in this biotope and confidence in the assessment is ‘Low’. | MediumHelp | Very LowHelp | MediumHelp |
Global warming (middle) [Show more]Global warming (middle)Middle emission scenario (by the end of this century 2081-2100) benchmark of:
EvidenceCerianthus lloydii adults are locally abundant in many localities on all coasts of the British Isles and in some areas are common on the shore. This species occurs on all western coasts of Europe from Greenland and Spitzbergen south to the Bay of Biscay. Larvae, but not adults, have been recorded from the Mediterranean (De Kluijver et al., 2024). OBIS (2024) lists records of Cerianthus lloydii from sea surface temperatures of -5 to 20°C, although the majority of records were from 10 to15°C. Similarly, the majority of records for other burrowing anemones (Mesacmaea mitchellii and Cereus pedunclatus) are also between 10 to 15°C. Cerianthus lloydii is predominantly distributed in northern regions, and is likely to move further northward as the climate changes and temperature shifts out of its preferred range. There is no further information available on the temperature tolerance of Cerianthus lloydii. Cerianthids can occur across wide temperature range (8.36 to 11.51°C) and depth ranges from shallow waters to deep-sea environments (238 to 1,070 m). Hydrozoans have been recorded in depths ranging to 8,400 m, indicating adaptations to varied thermal niches throughout the water column (Davies et al., 2014; Stepanjants & Chernyshev, 2015). However, there is limited evidence for thermal thresholds and thermal ranges were available for the characterizing species recorded in this biotope and large knowledge gaps limit current understanding of the ecological feedback that may occur to cerianthids as a result of climate change driven temperature increase. Sensitivity assessment. Under the middle and high emission and extreme scenarios seawater temperatures are expected to temperatures rise by 3 to 5°C to potential southern summer temperatures of 23 to 24°C and northern summer temperatures of 17 to 19°C. The distribution of the important characterizing species Cerianthus lloydii suggest that they are probably resistant of chronic change in temperature for a year, but exposure to a short-term acute increase in temperature may cause Cerianthus lloydii to withdraw into their burrows temporarily. But most records of Cerianthus lloydii occur north of the Bay of Biscay so there is the possibility that it may be driven north or the greater depth to avoid ongoing climate mediated temperature increases. Therefore, for all three scenarios (middle and high emission and extreme scenarios) resistance is assessed as ‘Medium’ as a precaution. Resilience is assessed as ‘Very Low’ due to the long-term nature of ocean warming. This biotope is assessed as ‘Medium’ sensitivity to ocean warming under all three scenarios. However, there is limited evidence on thermal tolerances of the characterizing species recorded in this biotope and confidence in the assessment is ‘Low’. | MediumHelp | Very LowHelp | MediumHelp |
Marine heatwaves (high) [Show more]Marine heatwaves (high)High emission scenario benchmark: A marine heatwave occurring every two years, with a mean duration of 120 days, and a maximum intensity of 3.5°C (Marine heatwave pressure definitions). EvidenceCerianthus lloydii adults are locally abundant in many localities on all coasts of the British Isles and in some areas are common on the shore. This species occurs on all western coasts of Europe from Greenland and Spitzbergen south to the Bay of Biscay. Larvae, but not adults, have been recorded from the Mediterranean (De Kluijver et al., 2024). OBIS (2024) lists records of Cerianthus lloydii from sea surface temperatures of -5 to 20°C, although the majority of records were from 10 to 15°C. Similarly, the majority of records for other burrowing anemones (Mesacmaea mitchellii and Cereus pedunclatus) are also between 10 to 15°C. There is no further evidence available on the upper thermal limit of Cerianthus lloydii. Sensitivity Assessment. Under the middle emission scenario, if heatwaves occurred every three years, with a maximum intensity of 2°C for 80 days by the end of this century, this could lead to summer sea temperatures reaching up to 24°C in southern England. Under the high emission scenario, if heatwaves occur every two years by the end of this century, reaching a maximum intensity of 3.5°C for 120 days, this could lead to the heatwave lasting the entire summer with temperatures reaching up to 26.5°C. As a precaution, this biotope has been assessed as having ‘Medium’ sensitivity to marine heatwaves. The recovery of Cerianthus lloydii populations is likely to be ‘Low’, hence, recovery may be interrupted by the occurrence of a further heatwave before the habitat can recover. Therefore, resilience has been assessed as ‘Very Low’, leading to a sensitivity assessment of ‘Medium’ for this biotope, but with ‘Low’ confidence. | MediumHelp | Very LowHelp | MediumHelp |
Marine heatwaves (middle) [Show more]Marine heatwaves (middle)Middle emission scenario benchmark: A marine heatwave occurring every three years, with a mean duration of 80 days, with a maximum intensity of 2°C. EvidenceCerianthus lloydii adults are locally abundant in many localities on all coasts of the British Isles and in some areas are common on the shore. This species occurs on all western coasts of Europe from Greenland and Spitzbergen south to the Bay of Biscay. Larvae, but not adults, have been recorded from the Mediterranean (De Kluijver et al., 2024). OBIS (2024) lists records of Cerianthus lloydii from sea surface temperatures of -5 to 20°C, although the majority of records were from 10 to 15°C. Similarly, the majority of records for other burrowing anemones (Mesacmaea mitchellii and Cereus pedunclatus) are also between 10 to 15°C. There is no further evidence available on the upper thermal limit of Cerianthus lloydii. Sensitivity Assessment. Under the middle emission scenario, if heatwaves occurred every three years, with a maximum intensity of 2°C for 80 days by the end of this century, this could lead to summer sea temperatures reaching up to 24°C in southern England. Under the high emission scenario, if heatwaves occur every two years by the end of this century, reaching a maximum intensity of 3.5°C for 120 days, this could lead to the heatwave lasting the entire summer with temperatures reaching up to 26.5°C. As a precaution, this biotope has been assessed as having ‘Medium’ sensitivity to marine heatwaves. The recovery of Cerianthus lloydii populations is likely to be ‘Low’, hence, recovery may be interrupted by the occurrence of a further heatwave before the habitat can recover. Therefore, resilience has been assessed as ‘Very Low’, leading to a sensitivity assessment of ‘Medium’ for this biotope, but with ‘Low’ confidence. | MediumHelp | Very LowHelp | MediumHelp |
Ocean acidification (high) [Show more]Ocean acidification (high)High emission scenario benchmark: a further decrease in pH of 0.35 (annual mean) and corresponding 120% increase in H+ ions, seasonal aragonite saturation of 20% of UK coastal waters and North Sea bottom waters, and the aragonite saturation horizon in the NE Atlantic, off the continental shelf, occurring at a depth of 400 m by the end of this century 2081-2100 (Ocean acidification pressure definitions). EvidenceIncreasing levels of CO2 in the atmosphere have led to the average pH of sea surface waters dropping from 8.25 in the 1700s to 8.14 in the 1990s (Jacobson, 2005). Decreased pH, and therefore shoaling of the calcium carbonate saturation horizon, may adversely impact UK sessile benthic communities (Danovaro et al., 2017). However, cerianthid anemones are not calcifying organisms, and therefore, may not be impacted by inhibited calcification due to pH decline. Furthermore, analyses that focused on taxa present in the North Atlantic indicated that deep-sea communities containing cerianthids may not be adversely impacted by ocean acidification (Johnson et al., 2018). Knowledge gaps and data paucity were highlighted as key limitations in the study, therefore, conclusive assessments of pH decline impacts to such communities could not be made (Johnson et al., 2018). There is no direct evidence regarding the effects of ocean acidification on Cerinthus lloydii or other burrowing anemones. Ocean acidification has been documented to reduce calcification rates in some hydrocorals (de Barros Marangoni et al., 2017). In addition, hydrozoan metabolites required for cell protection from osmotic and thermal stress (betaine) have been found to be inhibited under extreme acidification (pH 7.7 to 7.75) as a result of climate change (Boco et al., 2019). In contrast, studies utilising over 40 years of Continuous Plankton Recorder (CPR) data from the North Sea have indicated a significant correlative relationship between increased hydrozoan abundance and a temporal pH decline of 0.2 (Attrill et al., 2007; Fabry et al., 2008). Furthermore, some hydrozoans have been indicated to have high tolerances to wide pH variability, exhibiting complete mortality at pH 4 and 10, and with high survival rates (>50%) within the pH range of 5 to 8.5 (Gutierre, 2012). However, tolerance ranges are likely to be species specific, therefore, it is possible that these findings cannot be inferred beyond the study. Sensitivity Assessment. Cerianthids are not calcifying organisms, therefore, they are not considered to be impacted by the shoaling of the calcium carbonate saturation horizon due to ocean acidification (Danovaro et al., 2017). Ocean acidification may limit calcification in some hydrocorals and has also been attributed to inhibiting metabolic function in hydrozoan metabolites required for cell protection against osmotic and thermal stress. (Boco et al., 2019; de Barros Marangoni et al., 2017). However, these impacts may be species-specific. Conversely, some hydrozoans have been found to be highly tolerant to wide pH ranges and CPR data have indicated a significant correlative relationship between increased hydrozoan abundance and increased acidification in the North Sea (Attrill et al., 2007; Fabry et al., 2008; Gutierre, 2012). Therefore, based on the evidence available, under both the middle and high emission scenarios resistance is assessed as ‘Medium’ to represent the possible impact on hydroids. Resilience is assessed as ‘Very Low’ as it is an ongoing long-term pressure, and sensitivity as ‘Medium’ at the benchmark level but with ‘Low’ confidence. | MediumHelp | Very LowHelp | MediumHelp |
Ocean acidification (middle) [Show more]Ocean acidification (middle)Middle emission scenario benchmark: a further decrease in pH of 0.15 (annual mean) and a corresponding 35% increase in H+ ions with no coastal aragonite undersaturation and the aragonite saturation horizon in the NE Atlantic, off the continental shelf, at a depth of 800 m by the end of this century, 2081-2100. EvidenceIncreasing levels of CO2 in the atmosphere have led to the average pH of sea surface waters dropping from 8.25 in the 1700s to 8.14 in the 1990s (Jacobson, 2005). Decreased pH, and therefore shoaling of the calcium carbonate saturation horizon, may adversely impact UK sessile benthic communities (Danovaro et al., 2017). However, cerianthid anemones are not calcifying organisms, and therefore, may not be impacted by inhibited calcification due to pH decline. Furthermore, analyses that focused on taxa present in the North Atlantic indicated that deep-sea communities containing cerianthids may not be adversely impacted by ocean acidification (Johnson et al., 2018). Knowledge gaps and data paucity were highlighted as key limitations in the study, therefore, conclusive assessments of pH decline impacts to such communities could not be made (Johnson et al., 2018). There is no direct evidence regarding the effects of ocean acidification on Cerinthus lloydii or other burrowing anemones. Ocean acidification has been documented to reduce calcification rates in some hydrocorals (de Barros Marangoni et al., 2017). In addition, hydrozoan metabolites required for cell protection from osmotic and thermal stress (betaine) have been found to be inhibited under extreme acidification (pH 7.7 to 7.75) as a result of climate change (Boco et al., 2019). In contrast, studies utilising over 40 years of Continuous Plankton Recorder (CPR) data from the North Sea have indicated a significant correlative relationship between increased hydrozoan abundance and a temporal pH decline of 0.2 (Attrill et al., 2007; Fabry et al., 2008). Furthermore, some hydrozoans have been indicated to have high tolerances to wide pH variability, exhibiting complete mortality at pH 4 and 10, and with high survival rates (>50%) within the pH range of 5 to 8.5 (Gutierre, 2012). However, tolerance ranges are likely to be species specific, therefore, it is possible that these findings cannot be inferred beyond the study. Sensitivity Assessment. Cerianthids are not calcifying organisms, therefore, they are not considered to be impacted by the shoaling of the calcium carbonate saturation horizon due to ocean acidification (Danovaro et al., 2017). Ocean acidification may limit calcification in some hydrocorals and has also been attributed to inhibiting metabolic function in hydrozoan metabolites required for cell protection against osmotic and thermal stress. (Boco et al., 2019; de Barros Marangoni et al., 2017). However, these impacts may be species-specific. Conversely, some hydrozoans have been found to be highly tolerant to wide pH ranges and CPR data have indicated a significant correlative relationship between increased hydrozoan abundance and increased acidification in the North Sea (Attrill et al., 2007; Fabry et al., 2008; Gutierre, 2012). Therefore, based on the evidence available, under both the middle and high emission scenarios resistance is assessed as ‘Medium’ to represent the possible impact on hydroids. Resilience is assessed as ‘Very Low’ as it is an ongoing long-term pressure, and sensitivity as ‘Medium’ at the benchmark level but with ‘Low’ confidence. | MediumHelp | Very LowHelp | MediumHelp |
Sea level rise (extreme) [Show more]Sea level rise (extreme)Extreme scenario benchmark: a 107 cm rise in average UK sea-level by the end of this century (2018-2100) (Sea-level rise pressure definitions). EvidenceSea-level rise is occurring through a combination of thermal expansion and ice melt. Sea levels have risen 1-3 mm yr-1 in the last century (Cazenave & Nerem, 2004, Church et al., 2004, Church & White, 2006). The most recent projections on sea-level rise suggest a rise of 50 cm under the middle emission scenario, 70 cm under the high emission scenario, and 107 cm under the extreme scenario. This biotope occurs in areas sheltered from wave action and subject to weak or negligible tidal streams (Hughes, 1998a). Understanding of how sea-level rise will affect tidal energy, and the tide-swept nature of a habitat, is fraught with uncertainty, although evidence appears to suggest that any alterations will be non-linear (Pickering et al., 2012, Li et al., 2016). Modelling potential outcomes of sea-level rise on the tidal and residual currents in the Bohai Sea, China showed effects were site dependent, with energy either increasing or decreasing (Li et al., 2016). Similarly, Pickering et al. (2012) found a similar pattern around the UK for tidal amplitude. The effects of sea-level rise and increased wave action may be increased further due to storms and storms surges. IPCC (2019) note that the frequency of extreme sea-level events (e.g. due to storms) are predicted to increase as sea-level rises, however there is no consensus on the future storm and, hence, wave climate around UK coasts (Mossman et al., 2015; Lowe et al., 2018; Palmer et al., 2018). Sensitivity assessment. This habitat occurs from 5 to 30 m, although Cerianthus lloydii has been recorded at depths ranging from 0 to 900 m (OBIS, 2024). Therefore, an increase in sea-level rise is unlikely to have a significant impact on this biotope. Therefore, resistance to sea-level rise has been assessed as ‘High’ for the middle (50 cm), and high (70 cm) emission scenario, and for the extreme scenario (107 cm). As no recovery is deemed necessary, resilience has been assessed as ‘High’, and therefore this species has been classified as ‘Not sensitive’ to sea-level rise at each of the benchmarks. | HighHelp | HighHelp | Not sensitiveHelp |
Sea level rise (high) [Show more]Sea level rise (high)High emission scenario benchmark: a 70 cm rise in average UK sea-level by the end of this century (2018-2100). EvidenceSea-level rise is occurring through a combination of thermal expansion and ice melt. Sea levels have risen 1-3 mm yr-1 in the last century (Cazenave & Nerem, 2004, Church et al., 2004, Church & White, 2006). The most recent projections on sea-level rise suggest a rise of 50 cm under the middle emission scenario, 70 cm under the high emission scenario, and 107 cm under the extreme scenario. This biotope occurs in areas sheltered from wave action and subject to weak or negligible tidal streams (Hughes, 1998a). Understanding of how sea-level rise will affect tidal energy, and the tide-swept nature of a habitat, is fraught with uncertainty, although evidence appears to suggest that any alterations will be non-linear (Pickering et al., 2012, Li et al., 2016). Modelling potential outcomes of sea-level rise on the tidal and residual currents in the Bohai Sea, China showed effects were site dependent, with energy either increasing or decreasing (Li et al., 2016). Similarly, Pickering et al. (2012) found a similar pattern around the UK for tidal amplitude. The effects of sea-level rise and increased wave action may be increased further due to storms and storms surges. IPCC (2019) note that the frequency of extreme sea-level events (e.g. due to storms) are predicted to increase as sea-level rises, however there is no consensus on the future storm and, hence, wave climate around UK coasts (Mossman et al., 2015; Lowe et al., 2018; Palmer et al., 2018). Sensitivity assessment. This habitat occurs from 5 to 30 m, although Cerianthus lloydii has been recorded at depths ranging from 0 to 900 m (OBIS, 2024). Therefore, an increase in sea-level rise is unlikely to have a significant impact on this biotope. Therefore, resistance to sea-level rise has been assessed as ‘High’ for the middle (50 cm), and high (70 cm) emission scenario, and for the extreme scenario (107 cm). As no recovery is deemed necessary, resilience has been assessed as ‘High’, and therefore this species has been classified as ‘Not sensitive’ to sea-level rise at each of the benchmarks. | HighHelp | HighHelp | Not sensitiveHelp |
Sea level rise (middle) [Show more]Sea level rise (middle)Middle emission scenario benchmark: a 50 cm rise in average UK sea-level by the end of this century (2081-2100). EvidenceSea-level rise is occurring through a combination of thermal expansion and ice melt. Sea levels have risen 1-3 mm yr-1 in the last century (Cazenave & Nerem, 2004, Church et al., 2004, Church & White, 2006). The most recent projections on sea-level rise suggest a rise of 50 cm under the middle emission scenario, 70 cm under the high emission scenario, and 107 cm under the extreme scenario. This biotope occurs in areas sheltered from wave action and subject to weak or negligible tidal streams (Hughes, 1998a). Understanding of how sea-level rise will affect tidal energy, and the tide-swept nature of a habitat, is fraught with uncertainty, although evidence appears to suggest that any alterations will be non-linear (Pickering et al., 2012, Li et al., 2016). Modelling potential outcomes of sea-level rise on the tidal and residual currents in the Bohai Sea, China showed effects were site dependent, with energy either increasing or decreasing (Li et al., 2016). Similarly, Pickering et al. (2012) found a similar pattern around the UK for tidal amplitude. The effects of sea-level rise and increased wave action may be increased further due to storms and storms surges. IPCC (2019) note that the frequency of extreme sea-level events (e.g. due to storms) are predicted to increase as sea-level rises, however there is no consensus on the future storm and, hence, wave climate around UK coasts (Mossman et al., 2015; Lowe et al., 2018; Palmer et al., 2018). Sensitivity assessment. This habitat occurs from 5 to 30 m, although Cerianthus lloydii has been recorded at depths ranging from 0 to 900 m (OBIS, 2024). Therefore, an increase in sea-level rise is unlikely to have a significant impact on this biotope. Therefore, resistance to sea-level rise has been assessed as ‘High’ for the middle (50 cm), and high (70 cm) emission scenario, and for the extreme scenario (107 cm). As no recovery is deemed necessary, resilience has been assessed as ‘High’, and therefore this species has been classified as ‘Not sensitive’ to sea-level rise at each of the benchmarks. | HighHelp | HighHelp | Not sensitiveHelp |
Hydrological Pressures
Use [show more] / [show less] to open/close text displayed
| Resistance | Resilience | Sensitivity | |
Temperature increase (local) [Show more]Temperature increase (local)Benchmark. A 5°C increase in temperature for one month, or 2°C for one year (Temperature change pressure definition). EvidenceSynarachnactis lloydii adults are locally abundant in many localities on all coasts of the British Isles and, in some areas, are common on the shore. This species occurs on all western coasts of Europe from Greenland and Spitzbergen south to Biscay. Larvae, but not adults, have been recorded from the Mediterranean. There is no further information available on the temperature tolerance of Synarachnactis lloydii. Nemertesia ramosa is found inshore to deeper water, being common throughout the British Isles and is distributed from Iceland to north-west Africa (Hayward & Ryland, 1994). In the Azores, for example, it is well known in the sublittoral at 15 to 158 m deep in the central group of islands, but historical records exist from seamounts down to bathyal grounds of nearly 1,000 m (Gomes-Pereira & Tempera, 2016). Gili & Hughes (1995) report that temperature is a critical factor stimulating or preventing reproduction and that most species have an optimal temperature for reproduction. However, limited evidence for thermal thresholds and thermal ranges was available for the characterizing species recorded in this biotope. Berrill (1949) reported that growth in Obelia commissularis (syn. dichotoma) was temperature dependent but ceased at 27°C. Hydranths did not start to develop unless the temperature was less than 20°C, and any hydranths under development would complete their development and rapidly regress at ca 25°C. Berrill (1948) reported that Obelia species were absent from a buoy in July and August during excessively high summer temperatures in Booth Bay Harbour, Maine, USA. Berrill (1948) reported that the abundance of Obelia species and other hydroids fluctuated greatly, disappearing and reappearing as temperatures rose and fell markedly above and below 20°C during this period. The upwelling of cold water (8 to 10°C colder than surface water) allowed colonies of Obelia sp. to form in large numbers. Cantero et al. (2002) describe the presence and year-round fertility of Obelia dichotoma, Kirchenpaureria pinnata, Nemertesia ramosa and Halecium spp. in the Mediterranean, indicating probable tolerance to temperature increases at the benchmark level. Sensitivity assessmentAt the level of the benchmark, a change in temperature is unlikely to have a negative impact on the biotope. Therefore, both resistance and resilience are assessed as ‘High’, and sensitivity is assessed as ‘Not sensitive’ at the benchmark level. | HighHelp | HighHelp | Not sensitiveHelp |
Temperature decrease (local) [Show more]Temperature decrease (local)Benchmark. A 5°C decrease in temperature for one month, or 2°C for one year (Temperature change pressure definition). EvidenceSynarachnactis lloydii adults are locally abundant in many localities on all coasts of the British Isles and, in some areas, are common on the shore. This species occurs on all western coasts of Europe from Greenland and Spitzbergen south to Biscay. No further information is available on the temperature tolerance of Synarachnactis lloydii. Orejas et al. (2012) describe the feeding ecology of Obelia dichotoma in an Arctic environment (Kongsfjorden, Svalbard) which experiences temperatures of 1-5°C (Beszczynska-Möller & Dye, 2013). Palerud et al. (2004) also describe the presence of Obelia dichotoma, Halecium halecinum and Nemertesia sp. in Svalbard. This suggests that the characterizing hydroids are probably tolerant of the lowest temperatures they are likely to encounter in Britain and Ireland of ca 4°C (Beszczynska-Möller & Dye, 2013). It should be noted that growth rates are reduced at low temperatures. Berrill (1949) reported that for Obelia, stolons grew, under optimal nutritive conditions, at less than 1 mm in 24 hrs at 10-12°C, 10 mm in 24 hrs at 16-17°C, and as much as 15-20 mm in 24 hrs at 20°C. Berrill (1948) also reported that the abundance of Obelia species and other hydroids fluctuated greatly, disappearing and reappearing as temperatures rose and fell markedly above and below 20°C during this period. The upwelling of cold water (8 to 10°C colder than surface water) allowed colonies of Obelia sp. to form in large numbers. In addition, the hydroids Obelia dichotoma, Halecium halecinum and Nemertesia sp. have been recorded in Svalbard (Orjas et al., 2012). Sensitivity assessmentAll species assessed are present in northern/boreal habitats and are unlikely to be affected at the benchmark level. Resistance has been assessed as ‘High’, and resilience as ‘High’. Therefore, sensitivity has been assessed as ‘Not sensitive’ at the benchmark level. | HighHelp | HighHelp | Not sensitiveHelp |
Salinity increase (local) [Show more]Salinity increase (local)Benchmark. An increase in one MNCR salinity category above the usual range of the biotope or habitat (Salinity regime change pressure definition). EvidenceNo evidence was found for osmoregulation by Synarachnactis (syn. Cerianthus) lloydii. Synarachnactis lloydii is recorded in biotopes with variable salinity regimes (18-40 psu), such as SS.SMx.CMx.ClloModHo, but most records occur in full salinity. Studies on hydroids, in general, have found that prey capture rates may be affected by salinity and temperature (Gili & Hughes, 1995), although no evidence was found for Nemertesia antennina. However, due to the lack of evidence for the characterizing species within this biotope an assessment of ‘No evidence’ has been given. | No evidence (NEv)Help | Not relevant (NR)Help | No evidence (NEv)Help |
Salinity decrease (local) [Show more]Salinity decrease (local)Benchmark. A decrease in one MNCR salinity category above the usual range of the biotope or habitat (Salinity regime change pressure definition detail). EvidenceNo evidence was found for osmoregulation by Synarachnactis (syn. Cerianthus) lloydii. Synarachnactis lloydii is recorded in biotopes with variable salinity regimes (18-40 psu), such as SS.SMx.CMx.ClloModHo, but most records occur in full salinity. Studies on hydroids, in general, have found that prey capture rates may be affected by salinity and temperature (Gili & Hughes, 1995), although no evidence was found for Nemertesia antennina. However, due to the lack of evidence for the characterizing species within this biotope an assessment of ‘No evidence’ has been given. | No evidence (NEv)Help | Not relevant (NR)Help | No evidence (NEv)Help |
Water flow (tidal current) changes (local) [Show more]Water flow (tidal current) changes (local)Benchmark. A change in peak mean spring bed flow velocity of between 0.1 m/s and 0.2 m/s for more than one year (Water flow pressure definition). EvidenceEvidence for the effect of changes in water flow on Synarachnactis lloydii is unavailable. This species is recorded from biotopes with a wide range of water flow regimes, from very weak to strong flow (Connor et al., 1997b). Therefore, it is likely to have a high tolerance to changes in water flow regimes. The characteristic hydroids are typically found in places of low to moderate water movement, although Hayward & Ryland (1995a) note that the abundant communities occur in narrow straits and headlands that may experience high levels of water flow. Hydroids can bend passively with water flow to reduce drag forces, prevent detachment and enhance feeding (Gili & Hughes, 1995). Hydroid growth form also varies to adapt to prevailing conditions, allowing species to occur in a variety of habitats (Gili & Hughes, 1995). Flow rates are an important factor for feeding in hydroids, and prey capture rates are higher in areas of greater turbulence (Gili & Hughes, 1995). The capture rate of zooplankton by hydroids is correlated with prey abundance (Gili & Hughes, 1995); thus, prey availability can compensate for sub-optimal flow rates. Water movements are also important to hydroids to prevent siltation, which can cause death (Round et al., 1961). Tillin & Tyler-Walters (2014) suggest that the range of flow speeds experienced by biotopes in which hydroids are found indicates that a change (increase or decrease) in the maximum water flow experienced by mid-range populations for the short periods of peak spring tide flow would not have negative effects on this ecological group. Sensitivity assessmentThis biotope is recorded from moderately strong (1-3 kn) to very weak flow (negligible) and wave exposed to very wave sheltered conditions from 5 m to 30 m depth. The biotope probably experiences wave-mediated flow in its more shallow examples, while tidal flow is more important in its deeper examples. The biotope probably would not occur in areas subject to both strong flow and wave action, nor in areas subject to very weak flow and shelter from wave action. Therefore, the biotope probably experiences a range of water flow and/or wave-mediated flow between the extremes cited above. Therefore, a change in the flow of 0.1 to 0.2 m/s is probably not significant, and resistance and resilience are assessed as ‘High’, so sensitivity is assessed as ‘Not sensitive’. | HighHelp | HighHelp | Not sensitiveHelp |
Emergence regime changes [Show more]Emergence regime changesBenchmark. 1) A change in the time covered or not covered by the sea for a period of ≥1 year, or 2) an increase in relative sea level or decrease in high water level for ≥1 year. (Emergence regime change pressure definition). EvidenceThis biotope does not occur in the intertidal, and consequently an increase in emergence is considered 'Not relevant' to this biotope. | Not relevant (NR)Help | Not relevant (NR)Help | Not relevant (NR)Help |
Wave exposure changes (local) [Show more]Wave exposure changes (local)Benchmark. A change in near shore significant wave height of >3% but <5% for more than one year (Wave action pressure definition). EvidenceNo evidence for the effect of changes in wave exposure on Synarachnactis lloydii was available. However, it is recorded from extremely wave sheltered to wave exposed sites (Connor et al., 1997b). Jackson (2004) reported that Nemertesia ramosa was intolerant of high wave exposure and only found in sheltered areas. Faucci & Boero (2000) recorded hydroid communities at two sites of different wave exposure and recorded the presence of Obelia dichotoma and Halecium spp. in both the exposed and sheltered sites, but only found Kirchenpaueria sp. in the sheltered site. Sensitivity assessmentThis biotope is recorded from moderately strong to very weak flow and wave exposed to very wave sheltered conditions from 5 m to 30 m depth. The biotope probably experiences wave-mediated flow in its more shallow examples, while tidal flow is more important in its deeper examples. The biotope probably would not occur in areas subject to both strong flow and wave action, nor in areas subject to very weak flow and shelter from wave action. Therefore, the biotope probably experiences a range of water flow and/or wave-mediated flow between the extremes cited above. Storms may mobilise the surface of the substratum and may explain the sparse fauna. An increase in wave exposure (e.g. to very exposed) may mobilise the sediment further, reducing the abundance of epifauna, but the important characteristic burrowing anemone would probably remain. Similarly, a further decrease in wave exposure may increase the abundance of epifauna, such as found in the sub-biotope SS.SMx.CMx.ClloMx.Nem. Therefore, resistance is assessed as 'Medium' to represent changes in the community while the biotope will probably remain. Hence, resilience is assessed as 'High,' and sensitivity as 'Low'. Confidence in the assessment is 'Low' due to the lack of direct evidence. | MediumHelp | HighHelp | LowHelp |
Chemical Pressures
Use [show more] / [show less] to open/close text displayed
| Resistance | Resilience | Sensitivity | |
Transition elements & organo-metal contamination [Show more]Transition elements & organo-metal contaminationBenchmark. Exposure of marine species or habitat to one or more relevant Transitional metal or organometal (e.g. TBT) contaminants via uncontrolled releases or incidental spills (Transitional metals and organometals pressure definition). EvidenceThis pressure is Not assessed but evidence is presented where available. | Not Assessed (NA)Help | Not assessed (NA)Help | Not assessed (NA)Help |
Hydrocarbon & PAH contamination [Show more]Hydrocarbon & PAH contaminationBenchmark. Exposure of marine species or habitat to one or more relevant hydrocarbon or polyaromatic hydrocarbon (PAH) contaminants via uncontrolled releases or incidental spills (Hydrocarbon & PAH pressure definition). EvidenceThis pressure is Not assessed but evidence is presented where available. | Not Assessed (NA)Help | Not assessed (NA)Help | Not assessed (NA)Help |
Synthetic compound contamination [Show more]Synthetic compound contaminationBenchmark. Exposure of marine species or habitat to one or more synthetic compound contaminants via uncontrolled releases or incidental spills (Synthetic compound contamination pressure definition). EvidenceThis pressure is Not assessed but evidence is presented where available. | Not Assessed (NA)Help | Not assessed (NA)Help | Not assessed (NA)Help |
Radionuclide contamination [Show more]Radionuclide contaminationBenchmark. An increase in 10µGy/h above background levels (Radionuclides contamination pressure definition). EvidenceNo evidence. | No evidence (NEv)Help | Not relevant (NR)Help | No evidence (NEv)Help |
Introduction of other substances [Show more]Introduction of other substancesBenchmark. Exposure of marine species or habitat to one or more relevant "other" substances (solid, liquid or gas) contaminants via uncontrolled releases or incidental spills (Introduction of other substances pressure definition). EvidenceThis pressure is Not assessed. | Not Assessed (NA)Help | Not assessed (NA)Help | Not assessed (NA)Help |
De-oxygenation [Show more]De-oxygenationBenchmark. Exposure to dissolved oxygen concentration of less than or equal to 2 mg/l for one week (a change from WFD poor status to bad status) (deoxygenation pressure definition). EvidenceIn general, respiration in most marine invertebrates does not appear to be significantly affected until extremely low concentrations are reached. For many benthic invertebrates, this concentration is about 2 ml/l (Herreid, 1980; Rosenberg et al., 1991; Diaz & Rosenberg, 1995). Cole et al. (1999) suggest possible adverse effects on marine species below 4 mg/l and probable adverse effects below 2mg/l. Hydroids mainly inhabit environments in which the oxygen concentration exceeds 5 ml/l (Gili & Hughes, 1995). Diaz & Rosenberg (1995) noted that anemones include species that were reported to be particularly tolerant of hypoxia (e.g. Cerianthus sp and Epizoanthus erinaceus). A major hypoxic event due to a pycnocline in the Gulf of Trieste resulted in a mass mortality of benthos between 12 and 26th September 1983 (Stachowitsch, 1992), during which the oxygen levels fell below 4.2 mg/l, became anoxic, and hydrogen sulphide and ammonia were released (Faganeli et al., 1985). Amongst the epifauna, even hypoxia resistant polychaetes and bivalves died after 4 to 5 days, and the only organisms to survive after one week were the anemones Cerianthus sp and Epizoanthus erinaceus, the gastropods Aporrhais pespelecani and Trunculariopsis trunculus and the sphinuculid Sipunculus nudis (Stachowitsch, 1992). Sensitivity assessmentThe above evidence suggests that Synarachnactis (syn. Cerianthus) lloydii would probably survive for a week at or below 2 mg O2/l while the hydroids would probably be reduced to resting stages. Therefore, a resistance of 'Low' is recorded to represent the probable significant mortality of hydroids in the community. However, the hydroids would recover rapidly, so that resilience is likely to be 'High' and sensitivity is assessed as 'Low'. | LowHelp | HighHelp | LowHelp |
Nutrient enrichment [Show more]Nutrient enrichmentBenchmark. Increased levels of the elements nitrogen, phosphorus, silicon, and iron in the marine environment compared to background concentrations (Nutrient enrichment pressure definition). EvidenceNo information was available on the effect of nutrient enrichment on Synarachnactis (syn. Cerianthus) lloydii. Witt et al. (2004) found that the hydroid Obelia sp. was more abundant in a sewage disposal area in the Weser estuary (Germany), which experienced sedimentation of 1 cm for more than 25 days. It should be noted that another hydroid (Sertularia cupressina) was reduced in abundance when compared with unimpacted reference areas. However, there is no direct evidence for the characterizing hydroid species Nemertesia anteninna. Hence, no evidence was found on which to base an assessment. | No evidence (NEv)Help | Not relevant (NR)Help | No evidence (NEv)Help |
Organic enrichment [Show more]Organic enrichmentBenchmark. A deposit of 100 gC/m2/yr (Organic enrichment pressure definition). EvidenceBorja et al. (2000) and Gittenberger & van Loon (2011), in the development of the AZTI Marine Biotic Index (AMBI) to assess disturbance (including organic enrichment), both assigned Synarachnactis (syn. Cerianthus) lloydii to their Ecological Group I, ‘species very sensitive to organic enrichment and present under unpolluted conditions (initial state)’. The basis for their assessment and relation to the pressure benchmark was not clear (Tillin & Tyler-Walters, 2014). Witt et al. (2004) found that the hydroid Obelia spp. was more abundant in a sewage disposal area in the Weser estuary (Germany) which experienced sedimentation of 1 cm for more than 25 days. It should be noted that another hydroid (Sertularia cupressina) was reduced in abundance when compared with unimpacted reference areas. As suspension feeders, an increase in organic content at the benchmark is likely to be of benefit to the characterizing hydroids. Sensitivity assessmentThis biotope is considered to have a 'Low' resistance at the pressure benchmark, which refers to enrichment rather than gross organic pollution. Hence, resilience is assessed as 'Medium' and sensitivity as 'Medium'. | LowHelp | MediumHelp | MediumHelp |
Physical Pressures
Use [show more] / [show less] to open/close text displayed
| Resistance | Resilience | Sensitivity | |
Physical loss (to land or freshwater habitat) [Show more]Physical loss (to land or freshwater habitat)Benchmark. A permanent loss of existing saline habitat within the site (Physical loss pressure definition). EvidenceAll marine habitats and benthic species are considered to have a resistance of ‘None’ to this pressure and to be unable to recover from a permanent loss of habitat; resilience is ‘Very Low’. Sensitivity within the direct spatial footprint of this pressure is, therefore ‘High’. Although no specific evidence is described, confidence in this assessment is ‘High’, due to the incontrovertible nature of this pressure. | NoneHelp | Very LowHelp | HighHelp |
Physical change (to another seabed type) [Show more]Physical change (to another seabed type)Benchmark. Permanent change from sedimentary or soft rock substrata to hard rock or artificial substrata, or vice versa (Physical change in subtratum type pressure definition). EvidenceIf the sedimentary habitat was replaced with a rocky habitat, the biotope would be lost because it is characterized by sandy, muddy gravel, on which the community depends. The resistance to this change is ‘None’, and the resilience is assessed as ‘Very low’ due to the permanent nature of the change in the substratum. The biotope is assessed to have a ‘High’ sensitivity to this pressure at the benchmark. | NoneHelp | Very LowHelp | HighHelp |
Physical change (to another sediment type) [Show more]Physical change (to another sediment type)Benchmark. Permanent change in one Folk class (based on UK SeaMap simplified classification) (Physical change in sediment type pressure definition). EvidenceSynarachnactis (syn. Cerianthus) lloydii is found in a very wide range of substrata (Tillin & Tyler-Walters, 2014), but only dominates the fauna in the mixed substrata biotope described in this biotope. A change in Folk class from mixed to coarse or sandy mud substrata would result in loss of the biotope, even though the population of Synarachnactis lloydii may remain. Nemertesia antennina and other hydroids are only found attached to large pebbles and cobbles within SS.SMx.CMx.ClloMx.Nem. A reduction in the presence of cobbles and pebbles due to a change in sediment type would also reduce the abundance of the characteristic hydroids. Sensitivity assessmentA change in the substratum by one Folk class would result in the loss of the biotope. Therefore, a resistance of ‘None’ is recorded. As resilience is 'Very low' (the pressure is a permanent change), sensitivity is, therefore, 'High'. | NoneHelp | Very LowHelp | HighHelp |
Habitat structure changes - removal of substratum (extraction) [Show more]Habitat structure changes - removal of substratum (extraction)Benchmark. The extraction of substratum to 30 cm (where substratum includes sediments and soft rock but excludes hard bedrock) (Removal of substratum pressure definition). EvidenceResistance is assessed as ‘None’ based on expert judgment but supported by the literature relating to the position of these species on or within the seabed. At the pressure benchmark, the exposed sediments are considered suitable for recolonization almost immediately following extraction. Recovery will be mediated by the scale of the disturbance and the suitability of the sedimentary habitat. Recovery is most likely to occur via larval recolonization. Resilience is probably ‘Low’, so that sensitivity is assessed as ‘High’. | NoneHelp | LowHelp | HighHelp |
Abrasion / disturbance of the surface of the substratum or seabed [Show more]Abrasion / disturbance of the surface of the substratum or seabedBenchmark. Damage to surface features (e.g. species and physical structures within the habitat) (Surface abrasion/disturbance pressure definition). EvidenceNo direct evidence was found to assess the sensitivity of Synarachnactis lloydii to surface abrasion. The burrowing habit of the species specifically assessed would confer some protection from surface disturbance, although individuals would be more exposed when close to the surface feeding. Synarachnactis lloydii inhabits a soft tube, which can be up to 40 cm long and is permanently buried. The anemone can move freely within the tube and can retract swiftly if required (Tillin & Tyler-Walters, 2014). The available evidence indicates that hydroids can be entangled and removed by abrasion. Drop-down video surveys of Scottish reefs exposed to trawling showed that visual evidence of damage to bryozoans and hydroids on rock surfaces was generally limited and restricted to scrape scars on boulders (Boulcott & Howell, 2011). The study showed that damage was incremental, with damage increasing with the frequency of trawls rather than a blanket effect occurring on the pass of the first trawls. Re-sampling of grounds that were historically studied (from the 1930s) indicated that some species have increased in areas subject to scallop fishing (Bradshaw et al., 2002). This study also found (unquantified) increase in abundance of tough-stemmed hydroids including Nemertesia spp.; whose morphology may have prevented excessive damage. Bradshaw et al. (2002) suggested that as well as having high resistance to abrasion pressures, Nemertesia spp. have benthic larvae that could rapidly colonize disturbed areas with newly exposed substrata close to the adult. Hydroids may also recover rapidly as the surface covering of hydrorhizae may remain largely intact, from which new uprights are likely to grow. In addition, the resultant fragments of colonies may be able to develop into new colonies. Hydroid colonies were still present in the heavily fished area, albeit at lower densities than in the closed area. This may largely be because the Isle of Man scallop fishery is closed from 1st June to 31st October (Andrews et al., 2011), so at the time the samples were taken for the study in question, the seabed had not been dredged for at least 3.5 months. The summer period is also the peak growing/breeding season for many marine species (Bradshaw et al., 2003). Physical disturbance by fishing gear has been shown to adversely affect sessile benthic and emergent epifaunal communities, with hydroid and bryozoan matrices reported to be greatly reduced in fished areas and increase when fishing activity is removed (Jennings & Kaiser, 1998; Sheehan et al., 2017; Kaiser et al., 2018; Long et al., 2021; Langton, Stirling & Boulcott, 2023). Sensitivity assessmentAbrasion at the surface only is considered likely to damage and remove epiphytic species. Synarachnactis lloydii can retract into its tube. However, there is the possibility of the tube being damaged, which could affect the health of the organism. Given the sessile, erect nature of hydroids, damage and mortality following a physical disturbance are likely to be significant. However, hydroids have rapid growth rates, and potentially high recruitment and can recover quickly from fragments or dormant resting stages. The resistance of the biotope is assessed as ‘Medium’, although the significance of the impact for the bed will depend on the spatial scale of the pressure footprint. Resilience is assessed as ‘Medium’ (2 to10 years), and sensitivity is assessed as ‘Medium’. | MediumHelp | MediumHelp | MediumHelp |
Penetration or disturbance of the substratum subsurface [Show more]Penetration or disturbance of the substratum subsurfaceBenchmark. Damage to sub-surface features (e.g. species and physical structures within the habitat) (Sub-surface penetration pressure definition). EvidencePenetration and disturbance of the substratum would result in similar effects as abrasion or removal of this biotope. Damage to Synarachnactis lloydii would be greater within this pressure, as their ability to retract within their tubes would be limited. Therefore, the resistance of the biotope is assessed as ‘Low’, although the significance of the impact for the bed will depend on the spatial scale of the pressure footprint. Resilience is assessed as ‘Medium’, and sensitivity is assessed as ‘Medium’. | LowHelp | MediumHelp | MediumHelp |
Changes in suspended solids (water clarity) [Show more]Changes in suspended solids (water clarity)Benchmark. A change in one rank on the WFD (Water Framework Directive) scale, e.g. from clear to intermediate for one year (Suspended sediment pressure definition). EvidenceAn increase in suspended sediment may have a deleterious effect on the suspension-feeding community. It is likely to clog their feeding apparatus to some degree, resulting in reduced ingestion over the benchmark period and, subsequently, a decrease in growth rate (Jackson, 2004). As the hydroids capture small prey in suspension (Gili & Hughes, 1995), a reduction in feeding efficiency could potentially lead to a reduction in overall biomass. No evidence on the effect of a change in turbidity on Synarachnactis lloydii could be found. Nemertesia ramosa is a passive suspension feeder, extracting seston from the water column. Increased siltation may clog up the feeding apparatus, requiring energetic expenditure to clear. Recovery is likely to take only a few days. (Jackson, 2004). A decrease in suspended sediment is likely to benefit the community associated with this biotope. The suspension feeders may be able to feed more efficiently due to a reduction in time and energy spent cleaning feeding apparatus. Over the course of the benchmark, the hydroids may increase in abundance. Sensitivity assessment.No directly relevant evidence was found to assess the effect of pressure. Resistance to this pressure is assessed as 'High' as an increase in turbidity may influence feeding and growth rates but not result in mortality of adults. Resilience is assessed as 'High' (by default), and the biotope is assessed as 'Not sensitive' to changes in turbidity at the benchmark level. | HighHelp | HighHelp | Not sensitiveHelp |
Smothering and siltation rate changes (light) [Show more]Smothering and siltation rate changes (light)Benchmark. ‘Light’ deposition of up to 5 cm of fine material added to the seabed in a single discrete event (Smothering pressure definition). EvidenceIn normal accretion, Synarachnactis lloydii keeps pace with the accretion and, as a result, develops burrows much larger than the animal itself (Schäfer, 1972; Bromley, 2012). Schäfer (1972) reported that an increase in depositional rate led to avoidance behaviour in Synarachnactis lloydii. The organism ceases tube building activity, and instead the animal bunches its tentacles and intrudes its way up to the new surface, where it establishes a new burrow. However, no information on the depth of material through which it can burrow was given. In general, it appears that hydroids are sensitive to silting (Boero, 1984; Gili & Hughes, 1995) and the decline of beds in the Wadden Sea has been linked to environmental changes including siltation. Round et al. (1961) reported that the hydroid Sertularia (now Amphisbetia) operculata died when covered with a layer of silt after being transplanted to sheltered conditions. Boero (1984) suggested that deepwater hydroid species develop upright, thin colonies that accumulate little sediment, while species in turbulent water movement were adequately cleaned of silt by water movement. Hughes (1977) found that maturing hydroids that were smothered with detritus and silt lost most of the hydrocladia and hydranths. After one month, the hydroids were seen to have recovered, but although neither the growth rate nor the reproductive potential appeared to have been affected, the viability of the planulae may have been affected. Nemertesia ramosa is an upright hydroid with a height of up to 15 cm. The colony structure is fairly tough and flexible. Smothering with 5 cm of sediment may cover over some individuals; others may just have the lower section of the main stem covered (Hayward & Ryland, 1994). Halecium halecinum can grow up to 25 cm, and Kirchenpaueria pinnata can grow to ca 10 cm (Hayward & Ryland, 1994). Some of the hydroid community is therefore likely to survive smothering by 5 cm. Sensitivity assessment. Synarachnactis lloydii will actively burrow up through sediment that has smothered the entrance to its burrow. The thickness of sediment through which Synarachnactis lloydii is able to burrow is not known. However, it can grow up to 15 cm in length, and its burrows can reach 40 cm in depth. Hence, smothering by 5 cm of sediment is unlikely to cause mortality of Synarachnactis lloydii. This pressure will also influence the hydroid species within SS.SMx.CMx.ClloMx.Nem. Given the information available, the resistance to this pressure is considered to be ‘High’, as is the resilience, so sensitivity is assessed as ‘Not sensitive’ at the benchmark level. | HighHelp | HighHelp | Not sensitiveHelp |
Smothering and siltation rate changes (heavy) [Show more]Smothering and siltation rate changes (heavy)Benchmark. ‘Heavy’ deposition of up to 30 cm of fine material added to the seabed in a single discrete event (Smothering pressure definition). EvidenceIn normal accretion, Synarachnactis lloydii keeps pace with the accretion and, as a result, develops burrows much larger than the animal itself (Schäfer, 1972; Bromley, 2012). Schäfer (1972) reported that an increase in depositional rate led to avoidance behaviour in Synarachnactis lloydii. The organism ceases tube building activity, and instead the animal bunches its tentacles and intrudes its way up to the new surface, where it establishes a new burrow. However, no information on the depth of material through which it can burrow was given. In general, it appears that hydroids are sensitive to silting (Boero, 1984; Gili & Hughes, 1995) and the decline of beds in the Wadden Sea has been linked to environmental changes including siltation. Round et al. (1961) reported that the hydroid Sertularia (now Amphisbetia) operculata died when covered with a layer of silt after being transplanted to sheltered conditions. Boero (1984) suggested that deepwater hydroid species develop upright, thin colonies that accumulate little sediment, while species in turbulent water movement were adequately cleaned of silt by water movement. Hughes (1977) found that maturing hydroids that were smothered with detritus and silt lost most of the hydrocladia and hydranths. After one month, the hydroids were seen to have recovered, but although neither the growth rate nor the reproductive potential appeared to have been affected, the viability of the planulae may have been affected. Nemertesia ramosa is an upright hydroid with a height of up to 15 cm. The colony structure is fairly tough and flexible. Smothering with 5 cm of sediment may cover over some individuals; others may just have the lower section of the main stem covered (Hayward & Ryland, 1994). Halecium halecinum can grow up to 25 cm, and Kirchenpaueria pinnata can grow to ca 10 cm (Hayward & Ryland, 1994). Some of the hydroid community is therefore likely to survive smothering by 5 cm. Sensitivity assessment. Synarachnactis lloydii will actively burrow up through sediment that has smothered the entrance to its burrow. The thickness of sediment through which Synarachnactis lloydii is able to burrow is not known. However, it can grow up to 15 cm in length, and its burrows can reach 40 cm in depth. Smothering by 30 cm of sediment may cause some mortality of Synarachnactis lloydii. This pressure will also influence the hydroid species within SS.SMx.CMx.ClloMx.Nem. Given the information available, the resistance to this pressure is considered to be ‘Medium’, as is the resilience, so sensitivity is assessed as ‘Medium’ at the benchmark level but with 'Low' confidence. | MediumHelp | MediumHelp | MediumHelp |
Litter [Show more]LitterBenchmark. The introduction of man-made objects able to cause physical harm (surface, water column, seafloor or strandline) (Litter pressure definition). EvidenceNot assessed. | Not Assessed (NA)Help | Not assessed (NA)Help | Not assessed (NA)Help |
Electromagnetic changes [Show more]Electromagnetic changesBenchmark. A local electric field of 1 V/m or a local magnetic field of 10 µT (Electromagnetic pressure definition). EvidenceEvidence on the effect of electromagnetic fields (EMFs) on benthic organisms is still severely lacking. Some studies have investigated the effect of anthropogenically induced EMFs on benthic invertebrates at intensities ranging between 2 nT and 40 mT, which is often much higher than in-situ measurements from subsea cables. While some report changes to behaviour, physiology, reproduction, development, immunology, cytotoxicity and orientation, others demonstrate no effect from exposure to the EMF (Albert et al., 2020; Hutchison et al., 2020), depending on the study species and duration and intensity of exposure. There have been no studies investigating the effect of EMFs at the population or community level for benthic organisms. Sensitivity assessment. No studies have examined the effect of EMFs on burrowing anemones or hydroids. Therefore, there is ‘Insufficient evidence’ on which to base an assessment of the likely sensitivity of Synarachnactis lloydii to EMFs. | Insufficient evidence (IEv)Help | Not relevant (NR)Help | Help |
Underwater noise changes [Show more]Underwater noise changesBenchmark. MSFD indicator levels (SEL or peak SPL) exceeded for 20% of days in a calendar year. Further detail EvidenceSpecies characterizing this habitat do not have hearing perception but vibrations may cause a response. However, noise, as defined by the pressure, is probably 'Not relevant'. | Not relevant (NR)Help | Not relevant (NR)Help | Not relevant (NR)Help |
Introduction of light or shading [Show more]Introduction of light or shadingBenchmark. A change in incident light via anthropogenic means (Introduced light or shade pressure definition). EvidenceSince 2016, research on artificial light at night (ALAN) has expanded considerably in the marine and coastal environment. Light was previously assumed to be of low ecological significance in subtidal and intertidal habitats, but there is now evidence that ALAN is widespread in the marine environment, with biologically relevant levels of light penetrating to depths of up to 50 m (Davies et al., 2020; Smyth et al., 2021). ALAN can alter biological processes across taxa and at multiple levels of organisation. Documented responses include disruption of diel and circalunar rhythms, changes in activity and foraging, altered predator–prey interactions, shifts in community composition, and impacts on algal growth and phenology (Davies et al., 2014, 2015; Gaston et al., 2017; Tidau et al., 2021; Lynn et al., 2022; Marangoni et al., 2022; Miller & Rice, 2023; Ferretti et al., 2025). Evidence for benthic habitats and assemblages specifically is beginning to emerge (e.g. Trethewy et al., 2023; Schaefer et al., 2025), but remains limited and fragmented, often focusing on single taxa or short-term experiments. Mortality thresholds, long-term consequences, and responses at the biotope scale are rarely addressed, and there are major gaps around indirect effects such as trophic cascades or habitat modification. Therefore, given the rapid expansion of the evidence base but the continuing lack of data at the level of individual biotopes, resistance and resilience cannot be robustly assessed. Sensitivity is therefore recorded as 'Insufficient evidence'. | Insufficient evidence (IEv)Help | Not relevant (NR)Help | Help |
Barrier to species movement [Show more]Barrier to species movementBenchmark. A permanent or temporary barrier to species movement over ≥50% of water body width or a 10% change in tidal excursion (Barrier to species movement pressure definition). EvidenceNot relevant – this pressure is considered applicable to mobile species, e.g. fish and marine mammals rather than seabed habitats. Physical and hydrographic barriers may limit propagule dispersal. But propagule dispersal is not considered under the pressure definition and benchmark. | Not relevant (NR)Help | Not relevant (NR)Help | Not relevant (NR)Help |
Death or injury by collision [Show more]Death or injury by collisionBenchmark. Injury or mortality from collisions of biota with both static or moving structures due to 0.1% of tidal volume on an average tide, passing through an artificial structure (Death for collision pressure definition). EvidenceNot relevant’ to seabed habitats. NB. Collision by grounding vessels is addressed under ‘surface abrasion. | Not relevant (NR)Help | Not relevant (NR)Help | Not relevant (NR)Help |
Visual disturbance [Show more]Visual disturbanceBenchmark. The daily duration of transient visual cues exceeds 10% of the period of site occupancy by the feature (Visual disturbance pressure definition). EvidenceNot relevant. | Not relevant (NR)Help | Not relevant (NR)Help | Not relevant (NR)Help |
Biological Pressures
Use [show more] / [show less] to open/close text displayed
| Resistance | Resilience | Sensitivity | |
Genetic modification & translocation of indigenous species [Show more]Genetic modification & translocation of indigenous speciesBenchmark. Translocation of indigenous species or the introduction of genetically modified or genetically different populations of indigenous species may result in changes in the genetic structure of local populations, hybridization, or a change in community structure (Translocation pressure definition). EvidenceHabitat restoration projects may translocate stock to repopulate areas of suitable habitat (Elsäßer et al., 2013). No evidence was found for detrimental effects arising from this practice in the habitat, although there is potential for the movement of pathogens and non-indigenous, invasive species. | No evidence (NEv)Help | Not relevant (NR)Help | No evidence (NEv)Help |
Introduction of microbial pathogens [Show more]Introduction of microbial pathogensBenchmark. The introduction of relevant microbial pathogens or metazoan disease vectors to an area where they are currently not present (e.g. Martelia refringens and Bonamia, Avian influenza virus, viral Haemorrhagic Septicaemia virus) (pathogen or disease pressure definition). EvidenceNo evidence was available on the effect of microbial pathogens on Synarachnactis (syn. Cerianthus) lloydii. Hydroids exhibit astonishing regeneration and rapid recovery from injury (Sparks, 1972), and the only inflammatory response is active phagocytosis (Tokin & Yaricheva, 1959, 1961, as cited in Sparks, 1972). No record of diseases in the characterizing hydroids could be found. Therefore, there was 'Insufficient evidence' to assess the effect of this pressure on the biotope. | Insufficient evidence (IEv)Help | Not relevant (NR)Help | Help |
Removal of target species [Show more]Removal of target speciesBenchmark. Removal of species targeted by fishery, shellfishery or harvesting at a commercial or recreational scale (targeted removal pressure definition). EvidenceNone of the characterizing species within this biotope are currently directly targeted in the UK and hence this pressure is considered to be ‘Not relevant’. | Not relevant (NR)Help | Not relevant (NR)Help | Not relevant (NR)Help |
Removal of non-target species [Show more]Removal of non-target speciesBenchmark. Removal of features or incidental non-targeted catch (by-catch) through targeted fishery, shellfishery or harvesting at a commercial or recreational scale (non-targeted removed pressure definition). EvidenceDirect, physical impacts from harvesting are assessed under the abrasion and penetration of the seabed pressures. The characterizing species within this biotope could easily be incidentally removed from this biotope as by-catch when other species are being targeted. The loss of these species and other associated species would decrease species richness and negatively impact ecosystem function. Removal of a large percentage of the characterizing species would alter the character of the biotope. The resistance to removal is ‘Low’ due to the easy accessibility of the biotopes' location and the inability of these species to evade collection. The resilience is ‘Medium’, with recovery only being able to begin when the harvesting pressure is removed altogether. This gives an overall sensitivity score of ‘Medium’. | MediumHelp | MediumHelp | MediumHelp |
Introduction or spread of invasive non-indigenous species (INIS) Pressures
Use [show more] / [show less] to open/close text displayed
| Resistance | Resilience | Sensitivity | |
The American slipper limpet, Crepidula fornicata [Show more]The American slipper limpet, Crepidula fornicataEvidenceThe American slipper limpet Crepidula fornicata was introduced to the UK and Europe in the 1870s from the Atlantic coasts of North America with imports of the eastern oyster Crassostrea virginica. It was recorded in Liverpool in 1870 and on the Essex coast in 1887-1890. It has spread through expansion and introductions along the full extent of the English Channel and into the European mainland (Blanchard, 1997, 2009; Bohn et al., 2012, 2013a, 2013b, 2015; De Montaudouin et al., 2018; Helmer et al., 2019; Hinz et al., 2011; McNeill et al., 2010; Powell-Jennings & Calloway, 2018; Preston et al., 2020; Stiger-Pouvreau & Thouzeau, 2015). Crepidula fornicata is recorded from shallow, sheltered bays, lagoons and estuaries or the sheltered sides of islands, in variable salinity (18 to 40), although it prefers ca 30 (Tillin et al., 2020). Larvae require hard substrata for settlement. It prefers muddy, gravelly, shell-rich substrata that include gravel, or shells of other Crepidula, or other species, e.g., oysters, and mussels. It is highly gregarious and seeks out adult shells for settlement, forming characteristic ‘stacks’ of adults. But it also recorded in a wide variety of habitats including clean sands, artificial substrata, Sabellaria alveolata reefs and areas subject to moderately strong tidal streams (Blanchard, 1997, 2009; Bohn et al., 2012, 2013a, 2013b, 2015; De Montaudouin et al., 2018; Hinz et al., 2011; Powell-Jennings & Calloway, 2018; Preston et al., 2020; Stiger-Pouvreau & Thouzeau, 2015; Tillin et al., 2020). High densities of Crepidula fornicata cause ecological impacts on sedimentary habitats. The species can form dense carpets that can smother the seabed in shallow bays, changing and modifying the habitat structure. At high densities, the species physically smothers the sediment, and the resultant build-up of silt, pseudofaeces, and faeces is deposited and trapped within the bed (Tillin et al., 2020; Fitzgerald, 2007; Blanchard, 2009; Stiger-Pouvreau & Thouzeau, 2015). The biodeposition rates of Crepidula are extremely high and, once deposited, form an anoxic mud, making the environment suitable for other species, including most infauna (Stiger-Pouvreau & Thouzeau, 2015; Blanchard, 2009). For example, in fine sands, the community is replaced by a reef of slipper limpets that provide hard substrata for sessile suspension-feeders (e.g., sea squirts, tube worms and fixed shellfish), while mobile carnivorous microfauna occupy spaces between or within shells, resulting in a homogeneous Crepidula dominated habitat (Blanchard, 2009). Blanchard (2009) suggested the transition occurred and became irreversible at 50% cover of the limpet. De Montaudouin et al. (2018) suggested that homogenization occurred above a threshold of 20-50 Crepidula /m2. Impacts on the structure of benthic communities will depend on the type of habitat that Crepidula colonizes. De Montaudouin & Sauriau (1999) reported that in muddy sediment dominated by deposit-feeders, species richness, abundance and biomass increased in the presence of high densities of Crepidula (ca 562 to 4772 ind./m2), in the Bay of Marennes-Oléron, presumably because the Crepidula bed provided hard substrata in an otherwise sedimentary habitat. In medium sands, Crepidula density was moderate (330-1300 ind./m2), but there was no significant difference between communities in the presence of Crepidula. Intertidal coarse sediment was less suitable for Crepidula, with only moderate or low abundances (11 ind./m2), and its presence did not affect the abundance or diversity of macrofauna. However, there was a higher abundance of suspension–feeders and mobile Crustacea in the absence of Crepidula (De Montaudouin & Sauriau, 1999). The presence of Crepidula as an ecosystem engineer has created a range of new niche habitats, reducing biodiversity as it modifies habitats (Fitzgerald, 2007). De Montaudouin et al. (1999) concluded that Crepidula did not influence macroinvertebrate diversity or density significantly under experimental conditions, on fine sands in Arcachon Bay, France. De Montaudouin et al. (2018) noted that the limpet reef increased the species diversity in the bed, but homogenised diversity compared to areas where the limpets were absent. In the Milford Haven Waterway (MHW), the highest densities of Crepidula were found in areas of sediment with hard substrata, e.g., mixed fine sediment with shell or gravel or both (grain sizes 16-256 mm), but while Crepidula density increased as gravel cover increased in the subtidal, the reverse was found in the intertidal (Bohn et al., 2015). Bohn et al. (2015) suggested that high densities of Crepidula in high-energy environments were possible in the subtidal but not the intertidal, suggesting the availability of this substratum type is beneficial for its establishment. Hinz et al. (2011) reported a substantial increase in the occurrence of Crepidula off the Isle of Wight, between 1958 and 2006, at a depth of ca 60 m, on hard substrata (gravel, cobbles, and boulders), swept by strong tidal streams. Presumably, Crepidula is more tolerant of tidal flow than the oscillatory flow caused by wave action, which may be less suitable (Tillin et al., 2020). Sensitivity assessmentThe evidence suggests that Crepidula could colonize mixed sediment habitats in the subtidal, typical of this biotope, due to the presence of gravel or any other hard substrata that can be used for larval settlement (Tillin et al., 2020). Bohn et al. (2015) demonstrated that Crepidula had a preference for gravelly habitats, while De Montaudouin & Sauriau (1999) and Bohn et al. (2015) noted that Crepidula densities were low in intertidal coarse sediments. Therefore, Crepidula has the potential to colonize, and modify the habitat and its associated community due to the introduction of Crepidula shell biomass, silt, pseudofaeces and faeces (Blanchard, 2009; Tillin et al., 2020), as occurs in maerl gravels (Grall & Hall-Spencer, 2003), resulting in the loss of the biotope. This is a wave exposed to very sheltered habitat, so storms may mobilise the sediment (JNCC, 2022), which may also mitigate or prevent colonization by Crepidula at high densities, although it has been recorded from areas of strong tidal streams (Hinz et al., 2011). Therefore, the habitat may be more suitable for Crepidula in wave sheltered areas of the biotope and where water movement is mediated by tidal flow rather than wave action, e.g., the deeper examples of the biotope. Therefore, resistance is assessed as 'Medium' in examples where wave action is high and subject to storms, but 'Low' in wave sheltered areas dominated by tidal flow. Resilience is assessed as 'Very low' as it would require the removal of Crepidula, probably by artificial means. Hence, sensitivity is assessed as 'High' based on the worst-case scenario. Crepidula has not yet been reported to occur in this biotope, so the confidence in the assessment is 'Low' and further evidence is required. | LowHelp | Very LowHelp | HighHelp |
The carpet sea squirt, Didemnum vexillum [Show more]The carpet sea squirt, Didemnum vexillumEvidenceThe carpet sea squirt Didemnum vexillum (syn. Didemnum vestitum; Didemnum vestum) is a colonial ascidian with rapidly expanding populations that have invaded most temperate coastal regions around the world (Kleeman, 2009; Stefaniak et al., 2012; Tillin et al., 2020). It is an ‘ecosystem engineer’ that can change or modify invaded habitats and alter biodiversity (Griffith et al., 2009; Mercer et al., 2009). Didemnum vexillum has colonized and established populations in the northeast Pacific, Canadian and USA coast; New Zealand; France, Spain, and the Wadden Sea, Netherlands; the Mediterranean Sea and Adriatic Sea (Bullard et al., 2007; Coutts & Forrest, 2007; Dijkstra et al., 2007; Valentine et al., 2007a; Valentine et al., 2007b; Lambert, 2009; Hitchin, 2012; Tagliapietra et al., 2012; Gittenberger et al., 2015; Vercaemer et al., 2015; Mckenzie et al., 2017; Cinar & Ozgul, 2023; Holt, 2024). In the UK, Didemnum vexillum has colonized Holyhead marina and Milford Haven, Wales; the west coast of Scotland (marinas around Largs, Clyde, Loch Creran and Loch Fyne), South Devon (Plymouth, Yealm, and Dartmouth estuaries), the Solent, northern Kent, Essex, and Suffolk coasts (Griffith et al., 2009; Lambert, 2009; Hitchin, 2012; Minchin & Nunn, 2013; Bishop et al., 2015; Mckenzie et al., 2017; Tillin et al., 2020, Holt, 2024; NBN, 2024). Although a widespread invader, Didemnum vexillum has a limited ability for natural dispersal since the pelagic larvae remain in the water column for a short time (up to 36 hours). Therefore, it has a short dispersal phase that can allow the species to build localized populations (Herborg et al., 2009; Vercaemer et al., 2015; Holt, 2024). However, Bullard et al. (2007) suggested that Didemnum vexillum can form new colonies asexually by fragmentation. Colonies can produce long tendrils from an encrusting colony, which can fragment, disperse and settle, attaching to suitable hard substrata elsewhere (Bullard et al., 2007; Lambert, 2009; Stefaniak & Whitlatch, 2014). A fragmented colony can spread naturally for up to three weeks, transported by ocean currents, attached to floating seaweed, seagrass or other floating biota, or as free-floating spherical colonies (Bullard et al., 2007; Lengyel et al., 2009; Stefaniak & Whitlatch, 2014; Holt, 2024). Fragments can reattach to suitable substrata within six hours of contact. Fragments have the potential to disperse around 20 km before reattachment (Lengyel et al., 2009). Valentine et al. (2007a) reported that colonies of Didemnum vexillum enlarged by 6 to 11 times by asexual budding after 15 days and enlarged 11 to 19 times after 30 days. Valentine et al. (2007a) concluded fragments could successfully grow, survive, and help to spread Didemnum vexillum. While natural fragmentation of tendrils is thought to allow Didemnum vexillum to invade longer distances and increase its dispersal potential, Stefaniak & Whitlatch (2014) found that only one tendril out of 80 reattached to the flat, bare substrata used in their study, because tendrils required an extensive (at least eight-hour) period of contact to reattach. Stefaniak & Whitlatch (2014) suggested that once fragmented from a colony, the success of tendril reattachment was limited, and reattachment was not a major contributor to the invasive success of Didemnum vexillum. However, Stefaniak & Whitlatch (2014) also found that larvae-packed tendril fragments may increase natural dispersal distance, reproduction, and invasive success of Didemnum vexillum, and increase the distance larvae can travel. Not all colonies produce tendrils at all locations. Human-mediated transport via aquaculture facilities, boat hulls, commercial fishing vessels, and ballast water is probably the most important vector that has aided the long-distance dispersal of Didemnum vexillum and explains its prevalence in harbours and marinas (Bullard et al., 2007; Dijkstra et al., 2007; Griffith et al., 2009; Herborg et al., 2009). Fragmentation of colonies during transport or human disturbance (such as trawling or dredging) could indirectly disperse the species and enable it to find suitable conditions for establishment (Herborg et al., 2009). For example, in oyster farms in British Columbia, large fragments of Didemnum sp. come off oyster strings when they are pulled out of water, and other fragments can be pulled off oysters and mussels and thrown back into the water, which is likely to aid dispersal of the invasive species (Bullard et al., 2007). Dijkstra et al. (2007) hypothesised that Didemnum sp. was introduced to the Gulf of Maine with oyster aquaculture in the Damariscotta River and transported via Pacific oysters. Didemnum vexillum was likely introduced into the UK from northern Europe or Ireland via poorly maintained or not antifouled vessels, movement of contaminated shellfish stock and aquaculture equipment, or via marine industries such as oil, gas, renewables, and dredging (Holt, 2024). Recent evidence from genetic material suggests that human-mediated dispersal, between marinas and shellfish culture sites, is the most likely pathway for connectivity of Didemnum vexillum populations throughout Ireland and Britain (Prentice et al., 2021; Holt, 2024). Didemnum vexillum can disperse away from artificial substrata, invading and colonizing natural substrata in surrounding areas (Tillin et al., 2020). Holt (2024) noted that Didemnum vexillum had not spread as far as feared in the UK since it was first recorded. The current evidence of Didemnum vexillum’s ability to spread on natural habitats in this area is sparse and often conflicting, complicated by genetics, and its apparent variable habitat preferences and tolerances and its variable ability to adapt to ‘new’ conditions (Holt 2024). Didemnum vexillum has a seasonal growth cycle that is influenced by temperature (Valentine et al., 2007a). In warmer months (June and July), colonies may be large and well-developed encrusting mats. Populations experience more rapid growth from July to September, sometimes continuing into December. Colonies begin to decline in health and ‘die-off’ when temperatures drop below 5°C during winter months from around October to April (Gittenberger, 2007; Valentine et al., 2007a; Herborg et al., 2009). Cold water months cause colonies to regress and reduce in size, yet they often regenerate as temperatures warm (Griffith et al., 2009; Kleeman, 2009; Mercer et al., 2009), although some populations may not survive winter at all (Dijkstra et al., 2007). The early growth phase, from May to July, is initiated by smaller colonies developing from remnants of colonies that survived the cold water (Valentine et al., 2007a). The seasonal growth cycle is also likely influenced by location. For example, the Didemnum sp. growth cycle for colonies in Sandwich tide pool (temperature range from -1°C to 24°C, with daily fluctuations) probably does not occur in deep offshore subtidal habitats in Georges Bank (annual temperature range from 4°C to 15°C, and daily fluctuations are minimal) (Valentine et al., 2007a). Larval release and recruitment typically occur between 14 and 20°C and slow or cease below 9 to 11°C as summer ends (Griffith et al., 2009; McKenzie et al., 2017). In New Zealand, recruitment occurs from November to July, where the highest average temperatures were recorded in February (18 to 22°C), and the lowest average temperatures were recorded in July (9 to 10°C) (Fletcher et al., 2013a). In this New Zealand study, higher water temperatures were associated with a higher level of recruitment (Fletcher et al., 2013a). Didemnum vexillum requires suitable hard substrata for successful settlement and the establishment of colonies. It can grow quickly and establish large colonies of dense encrusting mats on a variety of hard substrata (Valentine et al., 2007a; Griffith et al., 2009; Lambert, 2009; Groner et al., 2011; Cinar & Ozgul, 2023). Gittenberger (2007) stated that invasive Didemnum sp. was a threat to native ecosystems because of its ability to overgrow virtually all hard substrata present. Suitable hard substrata can include rocky substrata such as bedrock, gravel, pebble, cobble, or boulders or artificial substrata such as a variety of maritime structures, such as pontoons, docks, wood and metal pilings, chains, ropes and moorings, plastic and ship hulls and at aquaculture facilities (Valentine et al., 2007a&b; Bullard et al., 2007; Griffith et al., 2009; Lambert, 2009; Tagliapietra et al., 2012; Tillin et al., 2020). Didemnum vexillum has been reported colonizing these types of hard substrata in the USA, Canada, northern Kent, and the Solent (Bullard et al., 2007; Valentine et al., 2007a; Valentine et al., 2007b; Hitchin, 2012; Vercaemer et al., 2015; Tillin et al., 2020). Didemnum vexillum has the ability to rapidly overgrow and displace on other sessile organisms such as other colonial ascidians (Ciona intestinalis, Styela clava, Ascidiella aspera, Botrylloides violaceus, Botryllus schlosseri, Diplosoma listerianium and Aplidium spp.), bryozoan, hydroids, sponges (Clione celata and Halichrondria sp.), anemone (Diadumene cincta), calcareous tube worms, eelgrass (Zostera marina), kelp (Laminaria spp. and Agarum sp.), green algae (Codium fragile subsp. fragile), red algae (Plocamium, Chondrus crispus and bush weed Agardhiella subulata), brown algae (Ascophyllum nodosum, Sargassum, Halidrys, Fucus evanescens and Fucus serratus), calcareous algae (Corallina officinalis), mussels (Mytilus galloprovincialis, Perna canaliculus and Mytilus edulis), barnacles, oysters (Magallana gigas, Ostrea edulis and Crassostrea virginica), sea scallops (Placopecten magellanicus), or dead shells (Dijkstra et al., 2007; Gittenberger, 2007; Valentine et al., 2007a; Valentine et al., 2007b; Griffith et al., 2009; Carman & Grunden, 2010; Dijkstra & Nolan, 2011; Groner et al., 2011; Hitchin, 2012; Tagliapietra et al., 2012; Minchin & Nunn, 2013; Gittenberger et al., 2015; Long & Groholz, 2015; Vercaemer et al., 2015). In contrast, Didemnum vexillum’s preference for sheltered conditions, established colonies observed in Georges Bank and Long Island Sound were exposed to moderately strong tidal currents (1 to 2 knots; ca 0.5 to 1 m/s recorded at both sites) that may mobilise sediment (Valentine et al., 2007b; Mercer et al., 2009; Tillin et al., 2020). However, Valentine et al. (2007b) describe the substratum as immobile, presumably consolidated, gravel, cobbles, and pebbles. Kleeman (2009) stated that the presence of a consistent mild wave action or ‘swash zone’ appears to favour Didemnum sp. establishment in the intertidal. Although some evidence suggests that waves and currents can facilitate the fragmentation and spread of Didemnum vexillum (Mckenzie et al., 2017), the tidal current velocities at some sites where Didemnum vexillum has been reported (for example, New England, where current velocities reach up to around 3 m/s) is lower than the current velocity required for the dislodgement of Didemnum vexillum fragments (around 7.6 m/s) (Reinhardt et al., 2012). This suggests that not all tidal currents are likely to dislodge Didemnum vexillum fragments. When on boat hulls, the species can experience higher current velocities, which are enough to cause dislodgement (Reinhardt et al., 2012). Kaplan et al. (2018) reported that Cerianthus tube anemones in the Georges Bank were less abundant in areas with higher per cent cover Didemnum vexillum, indicating a negative association between the two species. Sensitivity assessmentDidemnum vexillum has been recorded in the sublittoral to depths of 81 m in Georges Bank and 30 m in Long Island, USA (Bullard et al., 2007; Valentine et al., 2007b; Mercer et al., 2009). This biotope occurs on sandy muddy gravel, containing cobbles, pebbles and shells which could provide a suitable hard substratum for colonization by Didemnum sp (Tillin et al., 2020). Didemnum vexillum is reported to prefer sheltered conditions but has also been recorded in moderately strong currents (Valentine et al., 2007b; Mercer et al., 2009; Tillin et al., 2020) and is predicted to survive stronger currents, as the current velocity which will dislodge Didemnum vexillum is around 7.6 m/s (Reinhardt et al., 2012). This biotope experiences very weak to moderately strong water flow (1 to 3 m/s) and very sheltered to moderately exposed wave exposure. However, the effect of wave action reduces with depth, so it is possible that only the most wave-exposed examples of the biotope could be unsuitable for Didemnum. Didemnum vexillum regresses as temperatures decline in winter, so shallow examples may be able to recover their condition in winter (Gittenberger, 2007; Valentine et al., 2007a; Herborg et al., 2009). However, deeper examples may not experience enough temperature change to trigger the decline in Didemnum vexillum (Valentine et al., 2007a). If Didemnum sp. could gain a 'foothold', it might overgrow, smother or cause mortality of epifauna. Holt (2024) noted that Didemnum vexillum had not spread as far as feared in the UK since it was first recorded. Therefore, a resistance of 'Medium' (some, <25% mortality) is suggested as a precaution in case Didemnum vexillum could colonize the biotope, but with 'Low' confidence due to the lack of direct evidence. Resilience is assessed as 'Very low' as recovery would require the physical removal of Didemnum sp., so sensitivity is assessed as 'Medium'. | MediumHelp | Very LowHelp | MediumHelp |
The Pacific oyster, Magallana gigas [Show more]The Pacific oyster, Magallana gigasEvidenceThe Pacific oyster, Magallana (syn. Crassostrea) gigas, is native to warm temperate regions from the northwest Pacific to Japan and northeast Asia, including Cape Mariya (Russia) to Hong Kong (China) (Carrasco & Baron, 2010; GBNNSIP, 2011, 2012). It is a fast-growing and tolerant species that has become a successful invader in the coastal waters of all continents, aside from Antarctica (Wrange et al., 2010; Carrasco & Baron, 2010; Padilla, 2010). Magallana gigas is recognised as a beneficial and important species in aquaculture worldwide (Padilla, 2010). It was initially introduced for aquaculture in Europe and the UK in the 1960s due to a decline in the Portuguese oyster (Crassostrea angulata) and the European flat oyster (Ostrea edulis) (Spencer et al., 1994; GBNNSIP, 2011, 2012; Humphreys et al., 2014 cited in Alves et al., 2021; Hansen et al., 2023). Since its introduction, the species has invaded and established self-sustaining natural populations throughout Europe from the North Sea, Wadden Sea and Scandinavian coastlines to the Atlantic coastlines of Spain and Portugal, as well as the Mediterranean and Adriatic Sea (Wrange et al., 2010; GBNNSIP, 2011, 2012; Ezgeta-Balic et al., 2019; Spagnolo et al., 2019; Bergstrom et al., 2021; Hansen et al., 2023). In the UK, the species predominantly occurs around the southern and western coastlines (OBIS, 2024; NBN, 2024). Shipping activity has also been associated with the introduction of Magallana gigas in the north-eastern Adriatic Sea, where it was not introduced for aquaculture (Ezgeta-Balic et al., 2019). It was also suggested that some Magallana gigas populations were established in south-west England from France, possibly via fouling on ships (GBNNSIP, 2011, 2012; Padilla, 2010; Ezgeta-Balic et al., 2019). Magallana gigas requires hard substrata for successful settlement and establishment, including littoral rock, bedrock, chalk, bare boulders, cobbles and pebbles and shells (Kochmann et al., 2012, 2013; McKinstry & Jensen, 2013; Herbert et al., 2016; Tillin et al., 2020) because its larvae require hard substrata for successful settlement and development (McKinstry & Jensen, 2013; Tillin et al., 2020). It also prefers mudflats with mixed sediment composed of shingle and sand, attaching to whatever hard substrata are available within otherwise unsuitable fine muddy sediment (Spencer et al., 1994; McKinstry & Jensen, 2013; Tillin et al., 2020). Invasive populations of Magallana gigas have been found on wave-exposed rocky shores to wave-sheltered soft sediment environments, and it has been described as a habitat generalist (Troost, 2010; Kochmann et al., 2012, 2013). For example, in Scotland, wild Magallana gigas are mainly located in the lower intertidal on bedrock, bedrock encrusted with barnacles, within bedrock crevices, and large and small boulders (Cook et al., 2014). They are unlikely to occur under boulders as they require access to the water column (Tillin et al., 2020). Patches of Pacific oyster reefs have been recorded on littoral rock in Kent, southern England and on littoral sediments in southern England, the North Sea, and the English Channel (Herbert et al., 2012, 2016; Morgan et al., 2021). Magallana gigas typically occurs in the lower intertidal and shallow subtidal, mostly abundant at depths 1 m to 10 m (Tillin et al., 2020). However, the preferred depth range varies with substratum. On littoral rock in Brittany, the Pacific oyster colonizes all intertidal levels from Mean High Water to Mean Low Water on sheltered (low energy), moderately exposed (moderate energy) and high energy rock shores (Herbert et al., 2012). However, in the Northwest Pacific, Magallana gigas is commonly found on sheltered low energy littoral rock and has less than 10% cover on exposed high energy littoral rock shores (Herbert et al., 2012, 2016). Magallana gigas was recorded in the mid intertidal on hard rock and artificial harbour structures in northern and eastern Adriatic, but absent from beam trawl surveys off the coast of Istria (Ezgeta-Balic et al., 2019). Ezgeta-Balic et al. (2019) noted that the only oysters found in their trawls were large Ostrea edulis, often confused for Magallana gigas by local fishermen. Magallana gigas has not been found at extreme low water levels or subtidally beneath rocky habitats, as it has been in soft sediment areas (Herbert et al., 2012). Sensitivity assessment.No reports were found of Magallana gigas existing with Synarachnactis lloydii. The sandy muddy gravel found in this biotope would provide suitable attachment for the species due to the presence of hard substrata (shells, pebbles and cobbles) that occur in this biotope. Most of the evidence suggests that Magallana gigas is limited to 10 m, but they can form beds down to 42 m where conditions allow (Smaal et al., 2009; Herbert et al., 2012, 2016; Tillin et al., 2020). Shallow examples of this biotope (5 to 10 m) may, therefore, be susceptible to invasion by Magallana gigas, given the sheltered nature in which they are found and the provision of suitable attachment substrata by both the mixed sediment. Therefore, a precautionary worst-case resistance of ‘Medium’ is suggested for this biotope. Resilience is 'Very low' as the Magallana gigas population would need to be removed for recovery to occur. Therefore, sensitivity is assessed as ‘Medium’. As Magallana gigas has not yet been reported to interact with either characterizing species from this biotope (2026), confidence in the assessment is ‘Low’. | MediumHelp | Very LowHelp | MediumHelp |
Wireweed, Sargassum muticum [Show more]Wireweed, Sargassum muticumEvidenceSargassum muticum is a circumglobal invasive species (Engelen et al., 2015). It is recorded (2015) from Norway to Morocco and into the Mediterranean in the eastern Atlantic and from Alaska to Baja California in the eastern Pacific and from southern Russia to southern China in the western Pacific (Engelen et al., 2015). It colonizes a variety of habitats and can tolerate -1°C to 30°C and survive salinities below 10 ppt, but has a preference for full salinity ranges, 30 to 34 psu. Although fertilization does not occur below 15 ppt and growth of germlings is limited below 10°C, it can complete its life cycle as long as temperatures are over 8°C for at least four months of the year (Engelen et al., 2015). However, its distribution is limited by the availability of hard substrata (e.g., stones >10 cm) and light (Staehr et al., 2000; Strong & Dring, 2011; Engelen et al., 2015). It is most abundant between 1 and 3 m below mean water. But it has been recorded at 18 m or 30 m in the clear waters of California. However, it is a poor competitor under low light and only develops dense canopies in shallow areas (Engelen et al., 2015). Sensitivity assessmentThe depth (5 to 30 m) and lack of large enough attachment substrata likely exclude macroalgae from this biotope. Hence, it is unlikely to be colonized by Sargassum. Therefore, resistance and resilience are ‘High’, and this biotope is assessed as 'Not sensitive’ to Sargassum muticum. | HighHelp | HighHelp | Not sensitiveHelp |
Wakame, Undaria pinnatifida [Show more]Wakame, Undaria pinnatifidaEvidenceUndaria pinnatifida (Wakame or Asian kelp) is a large brown seaweed and an Invasive Non-Indigenous Species (INIS) that could out-compete native UK macroalgae species (Farrell & Fletcher, 2006; Thompson & Schiel, 2012; Brodie et al., 2014; Heiser et al., 2014; Arnold et al., 2016; Epstein & Smale, 2017, 2018; Kraan, 2017; Epstein et al., 2019a,b; Tidbury, 2020). Undaria pinnatifida originates from Japan but is currently established on the coastlines of New Zealand, Australia, Northern France, Spain, Italy, the UK, Portugal, Belgium, Holland, Argentina, Mexico, and the USA (De Leij et al., 2017). Undaria pinnatifida was first recorded in the UK in the Hamble Estuary in 1994 (Macleod et al., 2016) and has since proliferated along UK coastlines. One year after its discovery at the Queen Anne Battery marina, Plymouth, it became a major fouling plant on pontoons (Minchin & Nunn, 2014). Although initially restricted to artificial habitats, such as marinas and ports, it is now widespread in natural habitats in several areas, including Plymouth Sound. In Plymouth Sound, Epstein et al. (2019b) found that within its depth range (+1 to –4 m), Undaria pinnatifida co-existed with seven species of canopy-forming brown macroalgae, including Laminaria hyperborea. Undaria pinnatifida seems to settle better on artificial substrata (e.g., floats, marinas or piers) than on natural rocky shores among local kelps (Vaz-Pinto et al., 2014). It is found predominantly in low intertidal to shallow subtidal habitats (Epstein et al., 2019b) and is significantly more abundant on artificial substrata compared to natural rocky substrata (Heiser et al., 2014; Epstein & Smale, 2018). Undaria pinnatifida has a wide physiological niche, meaning it can occur in both coastal and estuarine environments, but has a preference for full salinity ranges, 27 to 33 psu, and displays tolerance for varying salinities, turbidity and siltation (Heiser et al., 2014; Epstein & Smale, 2018). Undaria pinnatifida has a greater preference for sites sheltered with low wave exposure and weak tidal streams (Heiser et al., 2014; Epstein & Smale, 2018). In natural habitats, Undaria pinnatifida was not recorded if the wave fetch was greater than 642 km and increased in abundance and cover in very sheltered sites (Epstein & Smale, 2018). Sensitivity assessmentThe depth (5 to 30 m) and lack of large enough attachment substrata likely exclude macroalgae from this biotope. Hence, it is unlikely to be colonized by Undaria. Therefore, resistance and resilience are ‘High’, and this biotope is assessed as 'Not sensitive’ to Undaria pinnatifida. | HighHelp | HighHelp | Not sensitiveHelp |
Other INIS [Show more]Other INISEvidenceCompass sea squirt, Asterocarpa humilis. This species has been observed colonizing intertidal and shallow subtidal habitats down to 26 m. It can tolerate fully marine to low estuarine salinities and appears to prefer sheltered sites such as harbours and marinas (Tillin et al., 2020). Given the overlap between depth ranges (5 to 30 m) and the availability of suitable attachment substrata (pebbles, cobbles, and gravel), this biotope is considered potentially suitable habitat for Asterocarpa humilis (Tillin et al., 2020). However, little is known about the potential impacts of Asterocapa humilis colonization, and no reports of it interacting with Synarachnactis lloydii were found. American jack knife clam, Ensis leei. This burrowing infaunal species can be found in coarse to muddy sediments, at depths from 5 to 100 m, and can reportedly withstand salinities of 7 to 32 ppt (Tillin et al., 2020). Given its preference for the soft substrata found in this biotope and the suitable depth and salinity range, it has been suggested (albeit with low confidence) as potentially suitable habitat for Ensis leei (Tillin et al., 2020); however, no reports of its colonization have been found. | Insufficient evidence (IEv)Help | Not relevant (NR)Help | Help |
Bibliography
Arnold, M., Teagle, H., Brown, M.P. & Smale, D.A., 2016. The structure of biogenic habitat and epibiotic assemblages associated with the global invasive kelp Undaria pinnatifida in comparison to native macroalgae. Biological Invasions, 18 (3), 661–676. DOI https://doi.org/10.1007/s10530-015-1037-6
Albert, L., Deschamps, F., Jolivet, A., Olivier, F., Chauvaud, L. & Chauvaud, S., 2020. A current synthesis on the effects of electric and magnetic fields emitted by submarine power cables on invertebrates. Marine Environmental Research, 159. DOI https://doi.org/10.1016/j.marenvres.2020.104958
Alves, M. T., Taylor, N. G. H. & Tidbury, H. J., 2021. Understanding drivers of wild oyster population persistence. Sci Rep, 11 (1), 7837. DOI https://doi.org/10.1038/s41598-021-87418-1
Andrews, J.W., Brand, A.R. & Holt, T.J., 2011. Isle of Man Queen Scallop Trawl and Dredge Fishery. MSC assessment report. pp. 203.
Attrill, M.J., Wright, J. & Edwards, M., 2007. Climate-related increases in jellyfish frequency suggest a more gelatinous future for the North Sea. Limnology and Oceanography, 52 (1), 480-485. DOI https://doi.org/10.4319/lo.2007.52.1.0480
Berghahn, R. & Offermann, U. 1999. Laboratory investigations on larval development, motility and settlement of white weed (Sertularia cupressina L.) - in view of its assumed decrease in the Wadden Sea. Hydrobiogia, 392(2), 233–239.
Bergström, P., Thorngren, L., Strand, Å & Lindegarth, M., 2021. Identifying high-density areas of oysters using species distribution modeling: Lessons for conservation of the native Ostrea edulis and management of the invasive Magallana (Crassostrea) gigas in Sweden. Ecology and Evolution, 11 (10), 5522-5532. DOI https://doi.org/10.1002/ece3.7451
Berrill, N.J., 1948. A new method of reproduction in Obelia. Biological Bulletin, 95, 94-99.
Berrill, N.J., 1949. The polymorphic transformation of Obelia. Quarterly Journal of Microscopical Science, 90, 235-264.
Beszczynska-Möller, A., & Dye, S.R., 2013. ICES Report on Ocean Climate 2012. In ICES Cooperative Research Report, vol. 321 pp. 73.
Bishop, J. D. D., Wood, C. A., Yunnie, A. L. E. & Griffiths, C. A., 2015. Unheralded arrivals: non-native sessile invertebrates in marinas on the English coast. Aquatic Invasions, 10 (3), 249-264. DOI https://doi.org/10.3391/ai.2015.10.3.01
Blanchard, M., 2009. Recent expansion of the slipper limpet population (Crepidula fornicata) in the Bay of Mont-Saint-Michel (Western Channel, France). Aquatic Living Resources, 22 (1), 11-19. DOI https://doi.org/10.1051/alr/2009004
Blanchard, M., 1997. Spread of the slipper limpet Crepidula fornicata (L.1758) in Europe. Current state and consequences. Scientia Marina, 61, Supplement 9, 109-118. Available from: http://scimar.icm.csic.es/scimar/index.php/secId/6/IdArt/290/
Boco, S.R., Pitt, K.A. & Melvin, S.D., 2019. Extreme, but not moderate climate scenarios, impart sublethal effects on polyps of the Irukandji jellyfish, Carukia barnesi. Science of The Total Environment, 685, 471-479. DOI https://doi.org/10.1016/j.scitotenv.2019.05.451
Boero, F., 1984. The ecology of marine hydroids and effects of environmental factors: a review. Marine Ecology, 5, 93-118.
Bohn, K., Richardson, C. & Jenkins, S., 2012. The invasive gastropod Crepidula fornicata: reproduction and recruitment in the intertidal at its northernmost range in Wales, UK, and implications for its secondary spread. Marine Biology, 159 (9), 2091-2103. DOI https://doi.org/10.1007/s00227-012-1997-3
Bohn, K., Richardson, C.A. & Jenkins, S.R., 2015. The distribution of the invasive non-native gastropod Crepidula fornicata in the Milford Haven Waterway, its northernmost population along the west coast of Britain. Helgoland Marine Research, 69 (4), 313.
Bohn, K., Richardson, C.A. & Jenkins, S.R., 2013a. Larval microhabitat associations of the non-native gastropod Crepidula fornicata and effects on recruitment success in the intertidal zone. Journal of Experimental Marine Biology and Ecology, 448, 289-297. DOI https://doi.org/10.1016/j.jembe.2013.07.020
Bohn, K., Richardson, C.A. & Jenkins, S.R., 2013b. The importance of larval supply, larval habitat selection and post-settlement mortality in determining intertidal adult abundance of the invasive gastropod Crepidula fornicata. Journal of Experimental Marine Biology and Ecology, 440, 132-140. DOI https://doi.org/10.1016/j.jembe.2012.12.008
Borja, A., Franco, J. & Perez, V., 2000. A marine biotic index to establish the ecological quality of soft-bottom benthos within European estuarine and coastal environments. Marine Pollution Bulletin, 40 (12), 1100-1114.
Boulcott, P. & Howell, T.R.W., 2011. The impact of scallop dredging on rocky-reef substrata. Fisheries Research (Amsterdam), 110 (3), 415-420.
Bradshaw, C., Collins, P. & Brand, A., 2003. To what extent does upright sessile epifauna affect benthic biodiversity and community composition? Marine Biology, 143 (4), 783-791.
Bradshaw, C., Veale, L.O., Hill, A.S. & Brand, A.R., 2002. The role of scallop-dredge disturbance in long-term changes in Irish Sea benthic communities: a re-analysis of an historical dataset. Journal of Sea Research, 47, 161-184. DOI https://doi.org/10.1016/S1385-1101(02)00096-5
Brodie J., Williamson, C.J., Smale, D.A., Kamenos, N.A., Mieszkowska, N., Santos, R., Cunliffe, M., Steinke, M., Yesson, C. & Anderson, K.M., 2014. The future of the northeast Atlantic benthic flora in a high CO2 world. Ecology and Evolution, 4 (13), 2787-2798. DOI https://doi.org/10.1002/ece3.1105
Bromley, R.G., 2012. Trace Fossils: Biology, Taxonomy and Applications: Routledge.
Bullard, S. G., Lambert, G., Carman, M. R., Byrnes, J., Whitlatch, R. B., Ruiz, G., Miller, R. J., Harris, L., Valentine, P. C., Collie, J. S., Pederson, J., McNaught, D. C., Cohen, A. N., Asch, R. G., Dijkstra, J. & Heinonen, K., 2007. The colonial ascidian Didemnum sp. A: Current distribution, basic biology and potential threat to marine communities of the northeast and west coasts of North America. Journal of Experimental Marine Biology and Ecology, 342 (1), 99-108. DOI https://doi.org/10.1016/j.jembe.2006.10.020
Cantero, Á.L.P., Carrascosa, A.M.G. & Vervoort, W., 2002. The benthic hydroid fauna of the Chafarinas Islands (Alborán Sea, western Mediterranean): Nationaal Natuurhistorisch Museum.
Carman, M.R. & Grunden, D.W., 2010. First occurrence of the invasive tunicate Didemnum vexillum in eelgrass habitat. Aquatic Invasions, 5 (1), 23-29. DOI https://doi.org/10.3391/ai.2010.5.1.4
Carrasco, Mauro F. & Barón, Pedro J., 2010. Analysis of the potential geographic range of the Pacific oyster Crassostrea gigas (Thunberg, 1793) based on surface seawater temperature satellite data and climate charts: the coast of South America as a study case. Biological Invasions, 12 (8), 2597-2607. DOI https://doi.org/10.1007/s10530-009-9668-0
Cazenave, A. & Nerem, R.S., 2004. Present-day sea-level change: Observations and causes. Reviews of Geophysics, 42 (3). DOI https://doi.org/10.1029/2003rg000139
Chauvaud, L., Jean, F., Ragueneau, O. & Thouzeau, G., 2000. Long-term variation of the Bay of Brest ecosystem: benthic-pelagic coupling revisited. Marine Ecology Progress Series, 200, 35-48. DOI https://doi.org/10.3354/meps200035
Chu, F. E., Volety, A. K. & Constantin, G., 1996. A comparison of Crassostrea gigas and Crassostrea virginica: effects of temperature asalinity on susceptibility to the protozoan parasite, Perkinsus marinus. Journal of Shellfish Research, 15 (2), 375–380.
Church, J.A. & White, N.J., 2006. A 20th century acceleration in global sea-level rise. Geophysical Research Letters, 33 (1). DOI https://doi.org/10.1029/2005gl024826
Church, J.A., White, N.J., Coleman, R., Lambeck, K. & Mitrovica, J.X., 2004. Estimates of the Regional Distribution of Sea Level Rise over the 1950–2000 Period. Journal of Climate, 17 (13), 2609-2625.
Cinar, M. E. & Ozgul, A., 2023. Clogging nets Didemnum vexillum (Tunicata: Ascidiacea) is in action in the eastern Mediterranean. Journal of the Marine Biological Association of the United Kingdom, 103. DOI https://doi.org/10.1017/s0025315423000802
Cole, S., Codling, I.D., Parr, W. & Zabel, T., 1999. Guidelines for managing water quality impacts within UK European Marine sites. Natura 2000 report prepared for the UK Marine SACs Project. 441 pp., Swindon: Water Research Council on behalf of EN, SNH, CCW, JNCC, SAMS and EHS. [UK Marine SACs Project.]. Available from: http://ukmpa.marinebiodiversity.org/uk_sacs/pdfs/water_quality.pdf
Connor, D.W., Allen, J.H., Golding, N., Howell, K.L., Lieberknecht, L.M., Northen, K.O. & Reker, J.B., 2004. The Marine Habitat Classification for Britain and Ireland. Version 04.05. ISBN 1 861 07561 8. In JNCC (2015), The Marine Habitat Classification for Britain and Ireland Version 15.03. [2019-07-24]. Joint Nature Conservation Committee, Peterborough. Available from https://mhc.jncc.gov.uk/
Connor, D.W., Brazier, D.P., Hill, T.O., & Northen, K.O., 1997b. Marine biotope classification for Britain and Ireland. Vol. 1. Littoral biotopes. Joint Nature Conservation Committee, Peterborough, JNCC Report no. 229, Version 97.06., Joint Nature Conservation Committee, Peterborough, JNCC Report No. 230, Version 97.06.
Cook, E., Beveridge, C., Lamont, P., O'Higgins, T. & Wilding, T., 2014. Survey of wild Pacific Oyster (Crassostrea gigas) in Scotland. Scottish Aquaculture Research Forum. DOI https://doi.org/10.13140/RG.2.1.1371.7369
Cornelius, P.F.S., 1992. Medusa loss in leptolid Hydrozoa (Cnidaria), hydroid rafting, and abbreviated life-cycles among their remote island faunae: an interim review.
Cornelius, P.F.S., 1995a. North-west European thecate hydroids and their medusae. Part 1. Introduction, Laodiceidae to Haleciidae. Shrewsbury: Field Studies Council. [Synopses of the British Fauna no. 50]
Coutts, A.D.M. & Forrest, B.M., 2007. Development and application of tools for incursion response: Lessons learned from the management of the fouling pest Didemnum vexillum. Journal of Experimental Marine Biology and Ecology, 342 (1), 154-162. DOI https://doi.org/10.1016/j.jembe.2006.10.042
Danovaro, R., Corinaldesi, C., Dell'Anno, A. & Snelgrove, P.V.R., 2017. The deep-sea under global change. Current biology: CB, 27 (11), R461-R465. DOI https://doi.org/10.1016/j.cub.2017.02.046
- Davies, J.S., Howell, K.L., Stewart, H.A., Guinan, J. & Golding, N., 2014. Defining biological assemblages (biotopes) of conservation interest in the submarine canyons of the South West Approaches (offshore United Kingdom) for use in marine habitat mapping. Deep Sea Research Part II: Topical Studies in Oceanography, 104, 208-229
Davies, T.W., McKee, D., Fishwick, J., Tidau, S. & Smyth, T., 2020. Biologically important artificial light at night on the seafloor. Scientific Reports, 10 (1). DOI https://doi.org/10.1038/s41598-020-69461-6
Davies, T.W., Coleman, M., Griffith, K.M. & Jenkins, S.R., 2015. Night-time lighting alters the composition of marine epifaunal communities. Biology Letters, 11 (4), 20150080. DOI https://doi.org/10.1098/rsbl.2015.0080
De Barros Marangoni, L.F., Calderon, E.N., Marques, J.A., Duarte, G.A.S., Pereira, C.M., e Castro, C.B. & Bianchini, A.J.C.R., 2017. Effects of CO2-driven acidification of seawater on the calcification process in the calcareous hydrozoan Millepora alcicornis (Linnaeus, 1758). 36 (4), 1133-1141. DOI https://doi.org/10.1007/s00338-017-1605-6
De Kluijver, M., Ingalsuo, S., Van Nieuwenhuijzen, A. and van Zanten, H.V., 2024. Macrobenthos of the North Sea. Vol. II – Anthozoa. [Online] Available from https://ns-anthozoa.linnaeus.naturalis.nl/linnaeus_ng/app/views/introduction/topic.php?id=3402
De Leij, R., Epstein, G., Brown, M.P. & Smale, D.A., 2017. The influence of native macroalgal canopies on the distribution and abundance of the non-native kelp Undaria pinnatifida in natural reef habitats. Marine Biology, 164 (7). DOI https://doi.org/10.1007/s00227-017-3183-0
De Montaudouin, X. & Sauriau, P.G., 1999. The proliferating Gastropoda Crepidula fornicata may stimulate macrozoobenthic diversity. Journal of the Marine Biological Association of the United Kingdom, 79, 1069-1077. DOI https://doi.org/10.1017/S0025315499001319
De Montaudouin, X., Andemard, C. & Labourg, P-J., 1999. Does the slipper limpet (Crepidula fornicata L.) impair oyster growth and zoobenthos diversity ? A revisited hypothesis. Journal of Experimental Marine Biology and Ecology, 235, 105-124.
De Montaudouin, X., Blanchet, H. & Hippert, B., 2018. Relationship between the invasive slipper limpet Crepidula fornicata and benthic megafauna structure and diversity, in Arcachon Bay. Journal of the Marine Biological Association of the United Kingdom, 98 (8), 2017-2028. DOI https://doi.org/10.1017/s0025315417001655
Diaz, R.J. & Rosenberg, R., 1995. Marine benthic hypoxia: a review of its ecological effects and the behavioural responses of benthic macrofauna. Oceanography and Marine Biology: an Annual Review, 33, 245-303.
Dijkstra, J. A. & Nolan, R., 2011. Potential of the invasive colonial ascidian, Didemnum vexillum, to limit escape response of the sea scallop, Placopecten magellanicus. Aquatic Invasions, 6 (4), 451-456. DOI https://doi.org/10.3391/ai.2011.6.4.10
Dijkstra, J., Harris, L.G. & Westerman, E., 2007. Distribution and long-term temporal patterns of four invasive colonial ascidians in the Gulf of Maine. Journal of Experimental Marine Biology and Ecology, 342 (1), 61-68. DOI https://doi.org/10.1016/j.jembe.2006.10.015
Elsäßer, B., Fariñas-Franco, J.M., Wilson, C.D., Kregting, L. & Roberts, D., 2013. Identifying optimal sites for natural recovery and restoration of impacted biogenic habitats in a special area of conservation using hydrodynamic and habitat suitability modelling. Journal of Sea Research, 77, 11-21.
Engelen, A.H., Serebryakova, A., Ang, P., Britton-Simmons, K., Mineur, F., Pedersen, M. F., & Toth, G., 2015. Circumglobal invasion by the brown seaweed Sargassum muticum. Oceanography and Marine Biology: An Annual Review, 53, 81-126.
Epstein, G. & Smale, D.A., 2017. Undaria pinnatifida: A case study to highlight challenges in marine invasion ecology and management. Ecology and Evolution, 7 (20), 8624-8642. DOI https://doi.org/10.1002/ece3.3430
Epstein, G. & Smale, D.A., 2018. Environmental and ecological factors influencing the spillover of the non-native kelp, Undaria pinnatifida, from marinas into natural rocky reef communities. Biological Invasions, 20 (4), 1049-1072. DOI https://doi.org/10.1007/s10530-017-1610-2
Epstein, G., Foggo, A. & Smale, D.A., 2019a. Inconspicuous impacts: Widespread marine invader causes subtle but significant changes in native macroalgal assemblages. Ecosphere, 10 (7). DOI https://doi.org/10.1002/ecs2.2814
Epstein, G., Hawkins, S.J. & Smale, D.A., 2019b. Identifying niche and fitness dissimilarities in invaded marine macroalgal canopies within the context of contemporary coexistence theory. Scientific Reports, 9. DOI https://doi.org/10.1038/s41598-019-45388-5
Ershova, E.A., Descoteaux, R., Wangensteen, O.S., Iken, K., Hoperoft, R.R., Smoot, C., Grebmeier, J.M. & Bluhm, B.A., 2019. Diversity and distribution of meroplanktonic larvae in the Pacific Arctic and connectivity with adult benthic invertebrate communities. Frontiers in Marine Science, 6. DOI https://doi.org/10.3389/fmars.2019.00490
Ezgeta-Balic, D., Segvic-Bubic, T., Staglicic, N., Lin, Y. P., Bojanic Varezic, D., Grubisic, L. & Briski, E., 2019. Distribution of non-native Pacific oyster Magallana gigas (Thunberg, 1793) along the eastern Adriatic coast. Acta Adriatica, 60 (2), 137-146. DOI https://doi.org/10.32582/aa.60.2.3
Fabry, V.J., Seibel, B.A., Feely, R.A. & Orr, J.C., 2008. Impacts of ocean acidification on marine fauna and ecosystem processes. ICES Journal of Marine Science, 65 (3), 414-432. DOI https://doi.org/10.1093/icesjms/fsn048
Faganeli, J., Avčin, A., Fanuko, N., Malej, A., Turk, V., Tušnik, P., Vrišer, B. & Vukovič, A., 1985. Bottom layer anoxia in the central part of the Gulf of Trieste in the late summer of 1983. Marine Pollution Bulletin, 16(2), 75-78.
Farrell, P. & Fletcher, R., 2006. An investigation of dispersal of the introduced brown alga Undaria pinnatifida (Harvey) Suringar and its competition with some species on the man-made structures of Torquay Marina (Devon, UK). Journal of Experimental Marine Biology and Ecology, 334 (2), 236-243.
Ferretti, M., Rossi, F., Benedetti-Cecchi, L. & Maggi, E., 2025. Ecological consequences of artificial light at night on coastal species in natural and artificial habitats: a review. Marine Biology, 172 (1). DOI https://doi.org/10.1007/s00227-024-04568-2
FitzGerald, A., 2007. Slipper Limpet Utilisation and Management. Final Report. Port of Truro Oyster Management Group., Truro, 101 pp. Available from https://www.shellfish.org.uk/files/Literature/Projects-Reports/0701-Slipper_Limpet_Report_Final_Small.pdf
Fletcher, L. M., Forrest, B. M., Atalah, J. & Bell, J. J., 2013a. Reproductive seasonality of the invasive ascidian Didemnum vexillum in New Zealand and implications for shellfish aquaculture. Aquaculture Environment Interactions, 3 (3), 197-211. DOI https://doi.org/10.3354/aei00063
Gaston, K.J., Davies, T.W., Nedelec, S.L. & Holt, L.A., 2017. Impacts of artificial light at night on biological timings. In Futuyma, D.J. (eds.). Annual Review of Ecology, Evolution, and Systematics, Vol 48 (1), pp. 49-68. DOI https://doi.org/10.1146/annurev-ecolsys-110316-022745
GBNNSIP, 2011b. Risk assessment for Crassostrea gigas. GB Non-native Species Information Portal, GB Non-native Species Secretariat. Available from: https://www.nonnativespecies.org/assets/Uploads/RA_Crassostrea_gigas_finalpoc.pdf
GBNNSIP, 2012. Pacific oyster Magallana gigas. Factsheet. GB Non-native Species Information Portal, [online] GB Non-native Species Secretariat. [Accessed July 2024]. Available from: https://www.nonnativespecies.org/non-native-species/information-portal/view/1013
Gili, J-M. & Hughes, R.G., 1995. The ecology of marine benthic hydroids. Oceanography and Marine Biology: an Annual Review, 33, 351-426.
Gittenberger, A, Rensing, M, Dekker, R, Niemantsverdriet, P, Schrieken, N & Stegenga, H, 2015. Native and non-native species of the Dutch Wadden Sea in 2014. Issued by Office for Risk Assessment and Research, The Netherlands Food and Consumer Product Safety Authority.
Gittenberger, A., 2007. Recent population expansions of non-native ascidians in The Netherlands. Journal of Experimental Marine Biology and Ecology, 342 (1), 122-126. DOI https://doi.org/10.1016/j.jembe.2006.10.022
Gittenberger, A. & Van Loon, W.M.G.M., 2011. Common marine macrozoobenthos species in the Netherlands, their characteristics and sensitivities to environmental pressures. GiMaRIS Report no 2011.08. DOI: https://doi.org/10.13140/RG.2.1.3135.7521
Gomes-Pereira, J. & Tempera, F., 2016. Hydroid gardens of Nemertesia ramosa (Lamarck, 1816) in the central North Atlantic. Marine Biodiversity, 46 (1), 85–94. DOI http://doi.org/10.1007/s12526-015-0325-9
Grall J. & Hall-Spencer J.M. 2003. Problems facing maerl conservation in Brittany. Aquatic Conservation: Marine and Freshwater Ecosystems, 13, S55-S64. DOI https://doi.org/10.1002/aqc.568
Griffith, K., Mowat, S., Holt, R.H., Ramsay, K., Bishop, J.D., Lambert, G. & Jenkins, S.R., 2009. First records in Great Britain of the invasive colonial ascidian Didemnum vexillum Kott, 2002. Aquatic Invasions, 4 (4), 581-590.
Groner, F., Lenz, M., Wahl, M. & Jenkins, S.R., 2011. Stress resistance in two colonial ascidians from the Irish Sea: The recent invader Didemnum vexillum is more tolerant to low salinity than the cosmopolitan Diplosoma listerianum. Journal of Experimental Marine Biology and Ecology, 409 (1), 48-52. DOI https://doi.org/10.1016/j.jembe.2011.08.002
Gutierre, S.M.M., 2012. pH tolerance of the biofouling invasive hydrozoan Cordylophora caspia. Hydrobiologia, 679 (1), 91-95. DOI https://doi.org/10.1007/s10750-011-0855-5
Hansen, B.W., Dolmer, P. & Vismann, B., 2023. Too late for regulatory management on Pacific oysters in European coastal waters? Journal of Sea Research, 191. DOI https://doi.org/10.1016/j.seares.2022.102331
Hatcher, A.M., 1998. Epibenthic colonization patterns on slabs of stabilised coal-waste in Poole Bay, UK. Hydrobiologia, 367, 153-162.
Hayward, P.J. & Ryland, J.S. 1994. The marine fauna of the British Isles and north-west Europe. Volume 1. Introduction and Protozoans to Arthropods. Oxford: Clarendon Press.
Hayward, P.J. & Ryland, J.S. (ed.), 1995. The marine fauna of the British Isles and north-west Europe. Volume 2. Molluscs to Chordates. Oxford Science Publications. Oxford: Clarendon Press.
Heiser, S., Hall-Spencer, J.M. & Hiscock, K., 2014. Assessing the extent of establishment of Undaria pinnatifida in Plymouth Sound Special Area of Conservation, UK. Marine Biodiversity Records, 7, e93. DOI https://doi.org/10.1017/S1755267214000608
Helmer, L., Farrell, P., Hendy, I., Harding, S., Robertson, M. & Preston, J., 2019. Active management is required to turn the tide for depleted Ostrea edulis stocks from the effects of overfishing, disease and invasive species. Peerj, 7 (2). DOI https://doi.org/10.7717/peerj.6431
Herbert, R.J.H., Humphreys, J., Davies, C.J., Roberts, C., Fletcher, S. & Crowe, T.P., 2016. Ecological impacts of non-native Pacific oysters (Crassostrea gigas) and management measures for protected areas in Europe. Biodiversity and Conservation, 25 (14), 2835-2865. DOI https://doi.org/10.1007/s10531-016-1209-4
Herbert, R.J.H., Roberts, C., Humphreys, J., & Fletcher, S. 2012. The Pacific oyster (Crassostrea gigas) in the UK: economic, legal and environmental issues associated with its cultivation, wild establishment and exploitation. Available from: https://www.daera-ni.gov.uk/publications/pacific-oyster-uk-issues-associated-its-cultivation-wild-establishment-and-exploitation
Herborg, L.M., O’Hara, P. & Therriault, T.W., 2009. Forecasting the potential distribution of the invasive tunicate Didemnum vexillum. Journal of Applied Ecology, 46 (1), 64-72. DOI https://doi.org/10.1111/j.1365-2664.2008.01568.x
Herreid, C.F., 1980. Hypoxia in invertebrates. Comparative Biochemistry and Physiology Part A: Physiology, 67 (3), 311-320. DOI https://doi.org/10.1016/S0300-9629(80)80002-8
Hinz, H., Capasso, E., Lilley, M., Frost, M. & Jenkins, S.R., 2011b. Temporal differences across a bio-geographical boundary reveal slow response of sub-littoral benthos to climate change. Marine Ecology Progress Series, 423, 69-82. DOI https://doi.org/10.3354/meps08963
Hitchin, B., 2012. New outbreak of Didemnum vexillum in North Kent: on stranger shores. Porcupine Marine Natural History Society Newsletter, 31, 43-48.
Holt, R., 2024. GB Non-native organism risk assessment for Didemnum vexillum. GB Non-native Species Information Portal, GB Non-native Species Secretariat. Available from: https://www.nonnativespecies.org/assets/Uploads/Didemnum-vexillum-final_forwebsite.pdf
Hughes, D.J., 1998a. Sea pens & burrowing megafauna (volume III). An overview of dynamics and sensitivity characteristics for conservation management of marine SACs. Natura 2000 report prepared for Scottish Association of Marine Science (SAMS) for the UK Marine SACs Project., Scottish Association for Marine Science. (UK Marine SACs Project). Available from: http://ukmpa.marinebiodiversity.org/uk_sacs/pdfs/seapens.pdf
Hughes, R.G., 1977. Aspects of the biology and life-history of Nemertesia antennina (L.) (Hydrozoa: Plumulariidae). Journal of the Marine Biological Association of the United Kingdom, 57, 641-657.
Humphreys, J., Herbert, R. J. H., Roberts, C. & Fletcher, S., 2014. A reappraisal of the history and economics of the Pacific oyster in Britain. Aquaculture, 428-429, 117–124. DOI https://doi.org/10.1016/j.aquaculture.2014.02.034
Hutchison, Z.L., Secor, D.H. & Gill, A.B., 2020. The interaction between resource species an electromagnetic fields associated with electricity production by offshore wind farms. Oceanography, 33 (4), 96–107. DOI https://doi/org/10.5670/oceanog.2020.409
IPCC (Intergovernmental Panel on Climate Change), 2019. IPCC Special Report on the Ocean and Cryosphere in a Changing Climate. Intergovernmental Panel on Climate Change, Geneva, Switzerland, 1170 pp. Available from https://www.ipcc.ch/srocc/home/
Jackson, A. 2004. Nemertesia ramosa, A hydroid. In Tyler-Walters H. and Hiscock K. (eds) Marine Life Information Network: Biology and Sensitivity Key Information Reviews [on-line]. Plymouth: Marine Biological Association of the United Kingdom. [cited 02/03/16] Available from: http://www.marlin.ac.uk/species/detail/1318
Jacobson, M.Z., 2005. Studying ocean acidification with conservative, stable numerical schemes for nonequilibrium air-ocean exchange and ocean equilibrium chemistry. Journal of Geophysical Research: Atmospheres, 110 (D7). DOI https://doi.org/10.1029/2004JD005220
Jennings, S. & Kaiser, M.J., 1998. The effects of fishing on marine ecosystems. Advances in Marine Biology, 34, 201-352.
Jensen, A.C., Collins, K.J., Lockwood, A.P.M., Mallinson, J.J. & Turnpenny, W.H., 1994. Colonization and fishery potential of a coal-ash artificial reef, Poole Bay, United Kingdom. Bulletin of Marine Science, 55, 1263-1276.
JNCC (Joint Nature Conservation Committee), 2022. The Marine Habitat Classification for Britain and Ireland Version 22.04. [Date accessed]. Available from: https://mhc.jncc.gov.uk/
JNCC (Joint Nature Conservation Committee), 2022. The Marine Habitat Classification for Britain and Ireland Version 22.04. [Date accessed]. Available from: https://mhc.jncc.gov.uk/
Johnson, D., Adelaide Ferreira, M. & Kenchington, E., 2018. Climate change is likely to severely limit the effectiveness of deep-sea ABMTs in the North Atlantic. Marine Policy, 87, 111-122. DOI https://doi.org/10.1016/j.marpol.2017.09.034
Kaiser, M.J., Hormbrey, S., Booth, J.R., Hinz, H. & Hiddink, J.G., 2018. Recovery linked to life history of sessile epifauna following exclusion of towed mobile fishing gear. Journal of Applied Ecology, 55 (3), 1060–1070. DOI https://doi.org/10.1111/1365-2664.13087
Kaplan, K.A., Hart, D.R., Hopkins, K., Gallager, S., York, A., Taylor, R. & Sullivan, P.J., 2018. Invasive tunicate restructures invertebrate community on fishing grounds and a large protected area on Georges Bank. Biological Invasions, 20 (1), 87–103. DOI https://doi.org/10.1007/s10530-017-1517-y
Kleeman, S.N., 2009. Didemnum vexillum - Feasibility of Eradication and/or Control. CCW Contract Science report, 53 pp. Available from: https://www.nonnativespecies.org/assets/Management-documents/Kleeman_2009-1.pdf
Kochmann, J, 2012. Into the Wild Documenting and Predicting the Spread of Pacific Oysters (Crassostrea gigas) in Ireland. PhD Thesis, University College Dublin. Available from: https://www.tcd.ie/research/simbiosys/images/JKPhD.pdf
Kochmann, J., O’Beirn, F., Yearsley, J. & Crowe, T.P., 2013. Environmental factors associated with invasion: modelling occurrence data from a coordinated sampling programme for Pacific oysters. Biological Invasions, 15 (10), 2265-2279. DOI https://doi.org/10.1007/s10530-013-0452-9
Kosevich, I.A. & Marfenin, N.N., 1986. Colonial morphology of the hydroid Obelia longissima (Pallas, 1766) (Campanulariidae). Vestnik Moskovskogo Universiteta Seriya Biologiya, 3, 44-52.
Kraan, S., 2017. Undaria marching on; late arrival in the Republic of Ireland. Journal of Applied Phycology, 29 (2), 1107-1114. DOI https://doi.org/10.1007/s10811-016-0985-2
Lambert, G., 2009. Adventures of a sea squirt sleuth: unraveling the identity of Didemnum vexillum, a global ascidian invader. Aquatic Invaders, 4(1), 5-28. DOI https://doi.org/10.3391/ai.2009.4.1.2
Langton, R., Stirling, D. & Boulcott, P., 2023. Using regional-scale predictive habitat models to assess protection and identify potential locations for additional management or monitoring for a species of conservation interest. Aquatic conservation: Marine and Freshwater Ecosystems, 33 (11), 1263–1280. DOI https://doi.org/10.1002/aqc.4021
Lengyel, N.L., Collie, J.S. & Valentine, P.C., 2009. The invasive colonial ascidian Didemnum vexillum on Georges Bank - Ecological effects and genetic identification. Aquatic Invasions, 4(1), 143-152. DOI https://doi.org/10.3391/ai.2009.4.1.15
Li, Y., Zhang, H., Tang, C., Zou, T. & Jiang, D., 2016. Influence of Rising Sea Level on Tidal Dynamics in the Bohai Sea. 74 (SI), 22-31. DOI https://doi.org/10.2112/si74-003.1
Long, H. A. & Grosholz, E. D., 2015. Overgrowth of eelgrass by the invasive colonial tunicate Didemnum vexillum: Consequences for tunicate and eelgrass growth and epifauna abundance. Journal of Experimental Marine Biology and Ecology, 473, 188-194. DOI https://doi.org/10.1016/j.jembe.2015.08.014
Long, S., Blicher, M., Arboe, N., Fuhrmann, M., Darling, M., Kemp, K., Nygaard, R., Zinglersen, K. & Yesson, C., 2021. Deep-sea benthic habitats and the impacts of trawling on them in the offshore Greenland halibut fishery, Davis Strait, west Greenland. ICES Journal of Marine Science, 78 (8), 2724–2744. DOI http://doi.org/10.1093/icesjms/fsab148
Lowe, J., Bernie, D., Bett, P., Bricheno, L., Brown, S., Calvert, D., Clark, R.T., Eagle, K.E., Edwards, T., Fosser, G., Fung, F., Gohar, L., Good, P., Gregory, J., Harris, G.R., Howard, T., Kaye, N., Kendon, E.J., Krijnen, J., Maisey, P., McDonald, R.E., McInnes, R.N., McSweeney, C.F., Mitchell, J.F.B., Murphy, J.M., Palmer, M., Roberts, C., Rostron, J.W., Sexton, D.M.H., Thornton, H.E., Tinker, J., Tucker, S., Yamazaki, K. & Belcher, S., 2018. UKCP18 Science Overview Report. Meterological Office, Hadley Centre, Exeter, UK, 73 pp. Available from https://www.metoffice.gov.uk/research/approach/collaboration/ukcp/index
Lynn, K.D., Quintanilla-Ahumada, D., Duarte, C. & Quijon, P. A., 2022. Hemocyanin as a biological indicator of artificial light at night stress in sandy beach amphipods. Marine Pollution Bulletin, 184. DOI https://doi.org/10.1016/j.marpolbul.2022.114147
Macleod, A., Cottier-Cook, E., Hughes, D. & Allen, C., 2016. Investigating the impacts of marine invasive non-native species. Natural England Commissioned Report NECR223, Natural England, 58 pp. Available from: https://pureadmin.uhi.ac.uk/ws/portalfiles/portal/3729569/NECR223_edition_1.pdf
Marangoni, L.F.B., Davies, T., Smyth, T., Rodríguez, A., Hamann, M., Duarte, C., Pendoley, K., Berge, J., Maggi, E. & Levy, O., 2022. Impacts of artificial light at night in marine ecosystems - A review. Global Change Biology, 28 (18), 5346–5367. DOI https://doi.org/10.1111/gcb.16264
McKenzie, C.H, Reid, V., Lambert, G., Matheson, K., Minchin, D., Pederson, J., Brown, L., Curd, A., Gollasch, S., Goulletquer, P, Occphipinti-Ambrogi, A., Simard, N. & Therriault, T.W., 2017. Alien species alert: Didemnum vexillum Kott, 2002: Invasion, impact, and control. ICES Cooperative Research Reports (CRR), 33 pp. DOI http://doi.org/10.17895/ices.pub.2138
McKinstry K. & Jensen A., 2013. Distribution, abundance and temporal variation of the Pacific oyster, Crassostrea gigas in Poole Harbour. Available from: https://assets.publishing.service.gov.uk/government/uploads/system/uploads/attachment_data/file/313003/fcf-oyster.pdf
McNeill, G., Nunn, J. & Minchin, D., 2010. The slipper limpet Crepidula fornicata Linnaeus, 1758 becomes established in Ireland. Aquatic Invasions, 5 (Suppl. 1), S21-S25. DOI https://doi.org/10.3391/ai.2010.5.S1.006
Medel, M., García, F. & Vervoort, W., 1998. The family Haleciidae (Cnidaria: Hydrozoa) from the Strait of Gibraltar and nearby areas. Zoologische Mededeelingen, 72, 29-50.
Menesguen, A. & Gregoris, T., 2018. Modelling benthic invasion by the colonial gastropod Crepidula fornicata and its competition with the bivalve Pecten maximus. 1. A new 0D model for population dynamics of colony-forming species. Ecological Modelling, 368, 277-287. DOI https://doi.org/10.1016/j.ecolmodel.2017.12.005
Mercer, J.M, Whitlatch, R.B, & Osman, R.W. 2009. Potential effects of the invasive colonial ascidian (Didemnum vexillum Kott, 2002) on pebble-cobble bottom habitats in Long Island Sound, USA. Aquatic Invasions, 4, 133-142. DOI https://doi.org/10.3391/ai.2009.4.1.14
MES (Marine Ecological Surveys), 2008. Marine Macrofauna Genus Trait Handbook. Marine Ecological Surveys Limited. Available from: https://www.researchgate.net/profile/Bryony-Pearce/publication/323855218_Genus_Trait_Handbook/links/5aafb798a6fdcc1bc0bd01ab/Genus-Trait-Handbook.pdf
Miller, C.R. & Rice, N., 2023. A synthesis of the risks of marine light pollution across organismal and ecological scales. Aquatic Conservation-Marine and Freshwater Ecosystems, 33 (12), 1590–1602. DOI https://doi.org/10.1002/aqc.4011
Minchin, D. & Nunn, J., 2014. The invasive brown alga Undaria pinnatifida (Harvey) Suringar, 1873 (Laminariales: Alariaceae), spreads northwards in Europe. Bioinvasions Records, 3 (2), 57-63. DOI http://dx.doi.org/10.3391/bir.2014.3.2.01
Minchin, D.M & Nunn, J.D., 2013. Rapid assessment of marinas for invasive alien species in Northern Ireland. Northern Ireland Environment Agency Research and Development Series, Northern Ireland Environment Agency.
Morgan, A., Slater, M., Mortimer, N., McNie, F., Singfield, C., Bailey, L., Covey, R., McNair, S., Waddell, C., Crundwell, R., Gall, A., Selley, H. & Packer, N., 2021. Partnership led strategy to monitor and manage spread of Pacific oyster populations in south Devon and Cornwall. Natural England Research Reports, NERR100. Natural England Research Reports, NERR100, Natural England, Truro, Cornwall, 258 pp. Available from: https://publications.naturalengland.org.uk/publication/4889256448491520#:~:text=Between 2017 and 2020, volunteers,method of controlling population expansion.
Mossman, H.L., Grant, A., Lawrence, P.J. & Davy, A.J., 2015. Biodiversity climate change impacts report card technical paper 10. Implications of climate change for coastal and inter-tidal habitats of the UK. Biodiversity climate change impacts, Living With Environmental Change, NERC, UKRI, 26 pp. Available from https://nerc.ukri.org/research/partnerships/ride/lwec/report-cards/biodiversity-source10/
NBN, 2024. National Biodiversity Network 2024(20/05/2024).https://data.nbn.org.uk/
OBIS (Ocean Biodiversity Information System), 2026. Global map of species distribution using gridded data. Available from: Ocean Biogeographic Information System. www.iobis.org. Accessed: 2026-09-09
Orejas, C., Rossi, S., Peralba, À., García, E., Gili, J.M. & Lippert, H., 2012. Feeding ecology and trophic impact of the hydroid Obelia dichotoma in the Kongsfjorden (Spitsbergen, Arctic). Polar biology, 36 (1), 61-72.
Padilla, D.K., 2010. Context-dependent impacts of a non-native ecosystem engineer, the Pacific Oyster Crassostrea gigas. Integrative and Comparative Biology, 50 (2), 213-225. DOI https://doi.org/10.1093/icb/icq080
Palerud, R., Gulliksen, B., Brattegard, T., Sneli, J.-A. & Vader, W., 2004. The marine macro-organisms in Svalbard waters. A catalogue of the terrestrial and marine animals of Svalbard. Norsk Polarinstitutt Skrifter, 201, 5-56.
Palmer, M., Howard, T., Tinker, J., Lowe, J., Bricheno, L., Calvert, D., Edwards, T., Gregory, J., Harris, G., Krijnen, J., Pickering, M., Roberts, C. & Wolf, J., 2018. UKCP18 Marine Report. Met Office, The Hadley Centre, Exeter, UK, 133 pp. Available from https://www.metoffice.gov.uk/pub/data/weather/uk/ukcp18/science-reports/UKCP18-Marine-report.pdf
Pickering, M.D., Wells, N.C., Horsburgh, K.J. & Green, J.A.M., 2012. The impact of future sea-level rise on the European Shelf tides. Continental Shelf Research, 35, 1-15. DOI https://doi.org/10.1016/j.csr.2011.11.011
Powell-Jennings, C. & Callaway, R., 2018. The invasive, non-native slipper limpet Crepidula fornicata is poorly adapted to sediment burial. Marine Pollution Bulletin, 130, 95-104. DOI https://doi.org/10.1016/j.marpolbul.2018.03.006
Prentice, M. B., Vye, S. R., Jenkins, S. R., Shaw, P. W. & Ironside, J. E., 2021. Genetic diversity and relatedness in aquaculture and marina populations of the invasive tunicate Didemnum vexillum in the British Isles. Biological Invasions, 23 (12), 3613-3624. DOI https://doi.org/10.1007/s10530-021-02615-3
Preston, J., Fabra, M., Helmer, L., Johnson, E., Harris-Scott, E. & Hendy, I.W., 2020. Interactions of larval dynamics and substrate preference have ecological significance for benthic biodiversity and Ostrea edulis Linnaeus, 1758 in the presence of Crepidula fornicata. Aquatic Conservation: Marine and Freshwater Ecosystems, 30 (11), 2133-2149. DOI https://doi.org/10.1002/aqc.3446
Ragueneau, O., Raimonet, M., Maze, C., Coston-Guarini, J., Chauvaud, L., Danto, A., Grall, J., Jean, F., Paulet, Y. M. & Thouzeau, G., 2018. The Impossible Sustainability of the Bay of Brest? Fifty Years of Ecosystem Changes, Interdisciplinary Knowledge Construction and Key Questions at the Science-Policy-Community Interface. Frontiers in Marine Science, 5. DOI https://doi.org/10.3389/fmars.2018.00124
Reinhardt, J.F., Gallagher, K.L., Stefaniak, L.M., Nolan, R., Shaw, M.T. & Whitlatch, R. B., 2012. Material properties of Didemnum vexillum and prediction of tendril fragmentation. Marine Biology, 159 (12), 2875-2884. DOI https://doi.org/10.1007/s00227-012-2048-9
Rosenberg, R., Hellman, B. & Johansson, B., 1991. Hypoxic tolerance of marine benthic fauna. Marine Ecology Progress Series, 79, 127-131. DOI https://dx.doi.org/10.3354/meps079127
Round, F.E., Sloane, J.F., Ebling, F.J. & Kitching, J.A., 1961. The ecology of Lough Ine. X. The hydroid Sertularia operculata (L.) and its associated flora and fauna: effects of transference to sheltered water. Journal of Ecology, 49, 617-629.
Schäfer, W., 1972. Ecology and palaeoecology of marine environments, 568 pp. Edinburgh: Oliver & Boyd.
Schaefer, N., Hoey, A.S., Bishop, M.J., Bugnot, A.B., Herbert, B., Mayer-Pinto, M., Sherman, C.D.H., Foster-Thorpe, C., Vozzo, M.L. & Dafforn, A., 2025. Shining the light on marine infrastructure: The use of artificial light to manipulate benthic marine communities. Journal of Applied Ecology, 62 (2), 220–230. DOI https://doi.org/10.1111/1365-2664.14843
Sheehan, E.V., Rees, A., Bridger, D., Williams, T. & Hall-Spencer, J.M., 2017. Strandings of NE Atlantic gorgonians. Biological Conservation, 209, 482–487. DOI https://doi.org/10.1016/j.biocon.2017.03.020
Smyth, T.J., Wright, A.E., McKee, D., Tidau, S., Tamir, R., Dubinsky, Z., Iluz, D. & Davies, T.W., 2021. A global atlas of artificial light at night under the sea. Elementa: Science of the Anthropocene, 9 (1). DOI https://doi.org/10.1525/elementa.2021.00049
Sommer, C., 1992. Larval biology and dispersal of Eudendrium racemosum (Hydrozoa, Eudendriidae). Scientia Marina, 56, 205-211. [Proceedings of 2nd International Workshop of the Hydrozoan Society, Spain, September 1991. Aspects of hydrozoan biology (ed. J. Bouillon, F. Cicognia, J.M. Gili & R.G. Hughes).]
Spagnolo, A., Auriemma, R., Bacci, T., Balkovic, I., Bertasi, F., Bolognini, L., Cabrini, M., Cilenti, L., Cuicchi, C., Cvitkovic, I., Despalatovic, M., Grati, F., Grossi, L., Jaklin, A., Lipej, L., Markovic, O., Mavric, B., Mikac, B., Nasi, F., Nerlovic, V., Pelosi, S., Penna, M., Petovic, S., Punzo, E., Santucci, A., Scirocco, T., Strafella, P., Trabucco, B., Travizi, A. & Zuljevic, A., 2019. Non-indigenous macrozoobenthic species on hard substrata of selected harbours in the Adriatic Sea. Marine Pollution Bulletin, 147, 150-158. DOI https://doi.org/10.1016/j.marpolbul.2017.12.031
Sparks, A., 1972. Invertebrate Pathology Noncommunicable diseases: Elsevier.
Spencer, B. E., Edwards, D. B., Kaiser, M. J. & Richardson, C. A., 1994. Spatfalls of the non-native Pacific oyster, Crassostrea gigas, in British waters. Aquatic Conservation: Marine and Freshwater Ecosystems, 4 (3), 203-217. DOI https://doi.org/10.1002/aqc.3270040303
Stachowitsch, M., 1992b. Benthic communities: eutrophication's memory mode. In The Response of marine transitional systems to human impact: problems and perspectives for restoration Proceedings of an International Conferencee, Bologna, Italy, 21-24 March, 1990, (ed. R.A. Vollenweider, R. Marchetti, & R. Viviani), pp.1017-1028. Amsterdam: Elsevier.
Staehr, P.A., Pedersen, M.F., Thomsen, M.S., Wernberg, T. & Krause-Jensen, D., 2000. Invasion of Sargassum muticum in Limfjorden (Denmark) and its possible impact on the indigenous macroalgal community. Marine Ecology Progress Series, 207, 79-88. DOI https://doi.org/10.3354/meps207079
Stefaniak, L. M. & Whitlatch, R. B., 2014. Life history attributes of a global invader: factors contributing to the invasion potential of Didemnum vexillum. Aquatic Biology, 21 (3), 221-229. DOI https://doi.org/10.3354/ab00591
Stefaniak, L., Zhang, H., Gittenberger, A., Smith, K., Holsinger, K., Lin, S. & Whitlatch, R.B., 2012. Determining the native region of the putatively invasive ascidian Didemnum vexillum Kott, 2002. Journal of Experimental Marine Biology and Ecology, 422-423, 64-71. DOI https://doi.org/10.1016/j.jembe.2012.04.012
Stepanjants, S.D. & Chernyshev, A.V., 2015. Deep-sea epibiotic hydroids from the abyssal plain adjacent to the Kuril–Kamchatka Trench with description of Garveia belyaevi sp. nov. (Hydrozoa, Bougainvilliidae). Deep Sea Research Part II: Topical Studies in Oceanography, 111, 44-48. DOI https://doi.org/10.1016/j.dsr2.2014.07.015
Stiger-Pouvreau, V. & Thouzeau, G., 2015. Marine Species Introduced on the French Channel-Atlantic Coasts: A Review of Main Biological Invasions and Impacts. Open Journal of Ecology, 5, 227-257. DOI https://doi.org/10.4236/oje.2015.55019
Strong, J.A. & Dring, M.J., 2011. Macroalgal competition and invasive success: testing competition in mixed canopies of Sargassum muticum and Saccharina latissima. Botanica Marina, 54 (3), 223-229.
Tagliapietra, D., Keppel, E., Sigovini, M. & Lambert, G., 2012. First record of the colonial ascidian Didemnum vexillum Kott, 2002 in the Mediterranean: Lagoon of Venice (Italy). Bioinvasions Records, 1 (4), 247-254. DOI http://dx.doi.org/10.3391/bir.2012.1.4.02
Thompson, G.A. & Schiel, D.R., 2012. Resistance and facilitation by native algal communities in the invasion success of Undaria pinnatifida. Marine Ecology, Progress Series, 468, 95-105.
Thouzeau, Gérard, Chauvaud, Laurent, Grall, Jacques & Guérin, Laurent, 2000. Rôle des interactions biotiques sur le devenir du pré-recrutement et la croissance de Pecten maximus (L.) en rade de Brest. Comptes Rendus de l#&39;Académie des Sciences - Series III - Sciences de la Vie, 323 (9), 815-825. DOI https://doi.org/10.1016/S0764-4469(00)01232-4
Thouzeau, G., Chavaud, L., Grall, J. & Guerin, L., 2000. Do biotic interactions control pre-recruitment and growth of Pecten maximus (L.) in the Bay of Brest ? Comptes rendus - acadamies des sciences, Paris, 323, 815-825.
Tidau, S., Smyth, T., McKee, D., Wiedenmann, J., D'Angelo, C., Wilcockson, D., Ellison, A., Grimmer, A.J., Jenkins, S.R., Widdicombe, S., Queiros, A.M., Talbot, E., Wright, A. & Davies, T.W., 2021. Marine artificial light at night: An empirical and technical guide. Methods in Ecology and Evolution, 12 (9), 1588–1601. DOI https://doi.org/10.1111/2041-210x.13653
Tidbury, H, 2020. Wakame (Undaria pinnatifida). GB Non-native Species Rapid Risk Assessment., 15 pp. Available from: http://www.nonnativespecies.org/index.cfm?pageid=143
Tillin, H. & Tyler-Walters, H., 2014b. Assessing the sensitivity of subtidal sedimentary habitats to pressures associated with marine activities. Phase 2 Report – Literature review and sensitivity assessments for ecological groups for circalittoral and offshore Level 5 biotopes. JNCC Report No. 512B, 260 pp. Available from: www.marlin.ac.uk/publications
Tillin, H.M., Kessel, C., Sewell, J., Wood, C.A. & Bishop, J.D.D., 2020. Assessing the impact of key Marine Invasive Non-Native Species on Welsh MPA habitat features, fisheries and aquaculture. NRW Evidence Report. Report No: 454. Natural Resources Wales, Bangor, 260 pp. Available from https://naturalresourceswales.gov.uk/media/696519/assessing-the-impact-of-key-marine-invasive-non-native-species-on-welsh-mpa-habitat-features-fisheries-and-aquaculture.pdf
Trethewy, M., Mayer-Pinto, M. & Dafforn, K.A., 2023. Urban shading and artificial light at night alter natural light regimes and affect marine intertidal assemblages. Marine Pollution Bulletin, 193. DOI https://doi.org/10.1016/j.marpolbul.2023.115203
Troost, K., 2010. Causes and effects of a highly successful marine invasion: case-study of the introduced Pacific oyster Crassostrea gigas in continental NW European estuaries. Journal of Sea Research, 64 (3), 145-165. DOI https://doi.org/10.1016/j.seares.2010.02.004
Valentine, P.C., Carman, M.R., Blackwood, D.S. & Heffron, E.J., 2007a. Ecological observations on the colonial ascidian Didemnum sp. in a New England tide pool habitat. Journal of Experimental Marine Biology and Ecology, 342 (1), 109-121. DOI https://doi.org/10.1016/j.jembe.2006.10.021
Valentine, P.C., Collie, J.S., Reid, R.N., Asch, R.G., Guida, V.G. & Blackwood, D.S., 2007b. The occurrence of the colonial ascidian Didemnum sp. on Georges Bank gravel habitat — Ecological observations and potential effects on groundfish and scallop fisheries. Journal of Experimental Marine Biology and Ecology, 342 (1), 179-181. DOI https://doi.org/10.1016/j.jembe.2006.10.038
Vaz-Pinto, F., Rodil, I.F., Mineur, F., Olabarria, C. & Arenas, F., 2014. Understanding biological invasions by seaweeds. In Pereira, L. & Neto, J.M. (eds.). Marine algae: biodiversity, taxonomy, environmental assessment and biotechnology. Boca Raton, Florida: CRC Press, pp. 140-177.
Vercaemer, B., Sephton, D., Clément, P., Harman, A., Stewart-Clark, S. & DiBacco, C., 2015. Distribution of the non-indigenous colonial ascidian Didemnum vexillum (Kott, 2002) in the Bay of Fundy and on offshore banks, eastern Canada. Management of Biological Invasions, 6, 385-394. DOI https://doi.org/10.3391/mbi.2015.6.4.07
Witt, J., Schroeder, A., Knust, R. & Arntz, W.E., 2004. The impact of harbour sludge disposal on benthic macrofauna communities in the Weser estuary. Helgoland Marine Research, 58 (2), 117-128.
Wood, L. E., Silva, T. A. M., Heal, R., Kennerley, A., Stebbing, P., Fernand, L. & Tidbury, H. J., 2021. Unaided dispersal risk of Magallana gigas into and around the UK: combining particle tracking modelling and environmental suitability scoring. Biological Invasions, 23 (6), 1719-1738. DOI https://doi.org/10.1007/s10530-021-02467-x
Wrange, A.L., Valero, J., Harkestad, L.S., Strand, Ø., Lindegarth, S., Christensen, H.T., Dolmer, P., Kristensen, P. S. & Mortensen, S., 2010. Massive settlements of the Pacific oyster, Crassostrea gigas, in Scandinavia. Biological Invasions, 12 (5), 1145-1152. DOI https://doi.org/10.1007/s10530-009-9535-z
Citation
This review can be cited as:
Last Updated: 15/07/2025