Alaria esculenta, Mytilus edulis and coralline crusts on very exposed sublittoral fringe bedrock
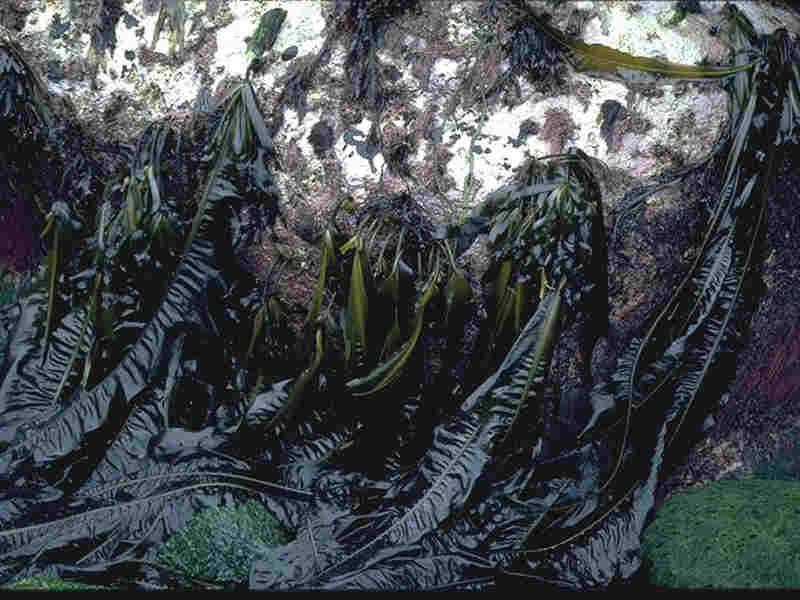
Alaria esculenta, Mytilus edulis and coralline crusts on very exposed sublittoral fringe bedrock
Photographer: Roger Mitchell Copyright: Joint Nature Conservation Committee (JNCC)

Map Key
- Orange points: Core Records
- Pale Blue points: Non-core, certain determination
- Black points: Non-core, uncertain determination
- Yellow areas: Predicted habitat extent
| Researched by | Emma Moyse, Owen Harris, Thomas Stamp, Emma Williams, Dr Harvey Tyler-Walters & Ellie Burdett | Refereed by | This information is not refereed |
|---|
Summary
UK and Ireland classification
Description
Very exposed sublittoral fringe bedrock characterized by the kelp Alaria esculenta and dense patches of small Mytilus edulis, both of which grow over a dense cover of encrusting coralline algae. Foliose red algae may also be present, but the species composition and their abundance varies between sites. Species such as Corallina officinalis, Mastocarpus stellatus and Plocamium cartilagineum occur widely. Limpets and barnacles are often common. Patches of anemones (such as Cylista elegans) and the hydroid Tubularia indivisa also occur in wave-surged areas. Laminaria digitata is usually absent, although stunted plants may be present at a few sites (typically greater than frequent). On very exposed shores this biotope is usually found beneath the Mytilus edulis-barnacle zone (ELR.MytB) and above the sublittoral Laminaria hyperborea forest (EIR.LhypR or EIR.LhypFa). In extremely exposed areas the Alaria zone may extend as deep at 15 m, where it generally has less Mytilus and greater densities of Tubularia (e.g. Barra and shallow areas of Rockall). This biotope is, however, distinguished from the deep Alaria forest (EIR.AlaAnSC) found on Rockall by its lack of short turf-forming hydroids. On less exposed shores an Alaria-dominated zone may, however, lie immediately above a narrow Laminaria digitata zone (MIR.Ldig). This biotope can also occur on exposed steep or vertical shores, where wave-crash restricts the growth of Laminaria digitata (JNCC, 2015, 2022).
Depth range
Lower shore, 0-5 mAdditional information
-
Sensitivity review
Sensitivity characteristics of the habitat and relevant characteristic species
IR.HIR.KFaR.Ala (and its sub-biotopes) and KFaR.AlaAnCrSp (reviewed separately) are characterized by the northern/boreal kelp Alaria esculenta and are indicative of very wave exposed sublittoral bedrock. IR.HIR.KFaR.Ala occurs predominantly on sublittoral fringe bedrock to a depth of 1 to 2 m. However, at extremely exposed sites, wave action can prevent competition with Laminaria hyperborea in the infralittoral zone and the Alaria esculenta-defined biotope KFaR.AlaAnCrSp can extend to a depth of 14 to 35 m under the KFaR.Ala.Myt biotopes, which occur at 5 to 13 m (JNCC, 2022). In slightly less wave exposed conditions, Laminaria digitata can compete with Alaria esculenta in the sub-biotope KFaR.Ala.Ldig where the two species form a mixed canopy.
The understorey community beneath Alaria esculenta canopies is defined by the degree of wave exposure at the site. Common understorey species across Alaria esculenta biotopes are encrusting coralline algae and Corallina officinalis turf. In the mixed Alaria esculenta and Laminaria digitata biotope KFaR.Ala.Ldig, the red seaweeds; Palmaria palmata, Mastocarpus stellatus and Chondrus crispus are predominant features of the understorey. In KFaR.Ala.Myt, Mytilus edulis is an abundant component of the understorey, while patches of anthozoans and the hydroid Tubularia spp. occur in more wave-surged areas.
In this sensitivity assessment, Alaria esculenta is the primary focus of research, as the dominant characteristic species, without which the biotopes would not be recognized. However, Laminaria digitata and Mytilus edulis are included as they define KFaR.Ala.Ldig and KFaR.Ala.Myt, respectively. Examples of important species groups are mentioned where appropriate.
Resilience and recovery rates of habitat
Alaria esculenta
Alaria esculenta is a perennial kelp found in the North Atlantic (Birkett et al., 1998b), which dominates the sublittoral fringe in areas exposed to severe wave action or where water surges along the sides of gullies or steep/vertical bedrock (Lewis, 1964; Connor et al., 2004; JNCC, 2022). In extreme wave action Laminaria digitata & Laminaria hyperborea are likely to become damaged and die back, whereas morphological features and high growth rates allow Alaria esculenta to survive in such conditions (Birkett et al., 1998b). Alaria esculenta has a compact holdfast, a flexible “short” stipe, and a flexible frond with a conspicuous reinforcing midrib (Birkett et al., 1998). Maximum growth rates are recorded in April-May, which can exceed 20 cm/month (Birkett et al., 1998b). From June-July, growth rates slow and continual erosion along the frond margins can reduce the sporophyte to a holdfast, stipe, and short length of the blade, in which state the sporophyte overwinters. In extremely wave exposed conditions, especially in winter months, the blade may be reduced to just the midrib. The sporophyte can reach a total length of 4 m (Werner & Kraan, 2004), fronds can reach a total length of 2 m, however, growth rates are locally variable, and fronds are more typically 30 to 90 cm in length (Birkett et al., 1998b). Alaria esculenta can reach maturity rapidly in 10 to 14 months and lives for 4 to 7 years (Birkett et al., 1998b; Baardseth, 1956).
Alaria esculenta has a heteromorphic life history (Fredersdorf et al., 2009). Between November to March a vast number of meiotic haploid zoospores are released from sori located on sporophylls (found at the top of the stipe). Zoospore dispersal is greatly influenced by local water movements and zoospore densities. Laminarian spores also need to settle in high density so that the resultant gametophytes are close enough to cross-fertilize (Fredriksen et al., 1995). Recruitment of Alaria esculenta may therefore be influenced by the proximity of mature sporophytes producing viable zoospores (Kain, 1979; Fredriksen et al., 1995). Laminarians are expected to disperse zoospores over considerable distances. However, Alaria esculenta may have a lower dispersal capacity than other Laminarians due to the basal location of the sporophylls (Norton, 1992). Sundene (1962) also observed that Alaria esculenta germlings were restricted to within 10 m of the parental source in an Alaria esculenta translocation experiment conducted in a Norwegian fjord.
Alaria esculenta is an opportunistic colonizing species (Kain 1975; Hawkins & Harkin 1985; Hill 1993; Engelen, 2010). Alaria esculenta can settle on bare surfaces, including mobile boulders and in deeper water than the infralittoral fringe. Alaria esculenta often appears early in the algal succession (approx. 3 months after clearance of dominant algae) before being outcompeted by other kelp species in moderately wave exposed shores. During kelp canopy removal experiments in the Isle of Man, Hawkins & Harkin (1985) found that in moderately wave exposed areas cleared of Laminaria digitata (the dominant canopy-forming species) Alaria esculenta became the dominant canopy algae within nine months (October to June) and Laminaria digitata did not re-establish dominance within the study period (15 months). In areas of moderate to sheltered wave exposure Alaria esculenta colonized the blocks within one month of clearance and reached 25% coverage within five months. However, within seven months, Laminaria digitata had outcompeted Alaria esculenta and re-established dominance within the community reaching 90 to 95% coverage.
The resilience of this Alaria esculenta can depend on any combination of factors that could be unrelated causes of disturbance. These factors can strongly affect the success of gametophytes and their development into sporophytes.
The development of Alaria esculenta gametophytes into sporophytes can also depend on light. Martins et al. (2022) showed that gametophyte growth increased with increasing daylength to a limit. While continuous light with no dark period resulted in faster growth, it also produced abnormal recruits with irregular form and reduced pigmentation. They also found that the direction of photoperiod effects on Alaria esculenta changed with life stage. Sporophytes that developed from the gametophytes under the increased daylengths grew slower than those that were cultured under the reduced daylengths. In addition, temperature was found to have an interactive effect with light. Elevated temperatures reduced growth, therefore exacerbating the effects of suboptimal light regimes experienced during the gametophyte stage.
Gametophytes are more likely to be more sensitive to siltation and smothering than mature sporophytes. Picard et al. (2022) showed that the addition of just 2.5 g of fine-grained sediment to petri dishes resulted in a single-grain layer of sediment as small as 63 to 125 μm in thickness which was enough to significantly hinder Alaria esculenta spore development. Moreover, Zacher et al. (2016) found that 10 g of sediment in petri dishes with Alaria esculenta gametophytes was enough to significantly reduce germination and sporophyte density.
Different optimum temperatures for gametophyte growth have been reported. Park et al. (2017) reported higher growth rates at 10 to 15°C than at 5°C in Alaria esculenta gametophytes sourced from Arctic waters. In addition, they reported gametophyte mortality at 20°C. Zacher et al. (2019) found that in Arctic populations, gametogenesis and sporophyte growth was reduced at 15°C compared to 9 to 10°C. They also found that co-cultivation with Laminaria digitata enhanced growth.
Sporophytes show rapid recovery of growth and photosynthetic activity after the return of light following polar night, where kelps spend months in total darkness, but this can be diminished by elevated temperatures by as little as 4°C (Gordillo et al., 2022; Cobos et al., 2026).
The timing of disturbance is likely to have significant effects on the resilience of Alaria esculenta. Silva et al. (2022) found that Alaria esculenta gametophytes cultured from sporophytes originating from Spitsbergen, Norway, showed no significant growth and no gametogenesis under natural winter conditions (2°C in complete darkness for 60 days). During the first 38 days, gametophyte density decreased by 42%, indicating limited resistance to prolonged darkness. However, density did not continue to decline during the remaining 22 days, suggesting an ability of surviving gametophytes to tolerate extended dark periods once initial mortality had occurred. Gametophytes did not become fertile after being returned to spring conditions (5°C a 12:12 h light:dark regime for 36 days), indicating limited resilience of this life stage to prolonged winter darkness and suggesting that sporogenesis, sexual reproduction and recruitment must occur during summer or autumn. Therefore, recovery following disturbance during winter may be more constrained than recovery following disturbance later in the year.
Mytilus edulis
Blue mussels, Mytilus edulis, are sessile, attached organisms that are unable to repair significant damage to individuals. Spawning occurs in spring and later summer allowing two periods of recruitment (Seed, 1969). Mytilus edulis has a high fecundity producing >1,000,000 eggs per spawning event. Larvae stay in the plankton for between 20 days to two months depending on water temperature (Bayne, 1976). In unfavourable conditions, they may delay metamorphosis for six months (Lane et al., 1985). Larval dispersal depends on the currents and the length of time they spend in the plankton. Larvae subject to ocean currents for up to six months can have a high dispersal potential.
Settlement occurs in two phases, an initial attachment using their foot (the pediveliger stage) and then a second attachment by the byssus thread before which they may alter their location to a more favourable one (Bayne, 1964). The final settlement often occurs around or between individual mussels of an established population. In areas of high water flow the mussel bed will rely on recruitment from other populations as larvae will be swept away and therefore recovery will depend on recruitment from elsewhere.
Larval mortality can be as high as 99% due to adverse environmental conditions, especially temperature, inadequate food supply (fluctuations in phytoplankton populations), inhalation by suspension feeding adult mytilids, difficulty in finding suitable substrata and predation (Lutz & Kennish, 1992). After settlement, the larvae and juveniles are subject to high levels of predation as well as dislodgement from waves and sand abrasion, depending on the area of settlement. Height on the shore generally determines lifespan, with mussels in the low shore only surviving between 2 to 3 years due to high predation levels whereas a wider variety of age classes are found higher up on the shore (Seed, 1969). Theisen (1973) reported that specimens of Mytilus edulis could reach 18 to 24 years of age.
Mainwaring et al. (2014) reviewed the evidence for recovery of Mytilus edulis beds from disturbance and an earlier study by Seed & Suchanek (1992) reviewed studies on the recovery of ‘gaps’ in Mytilus spp. beds. It was concluded that beds occurring high on the shore and on less exposed sites took longer to recover after a disturbance event than beds found low on the shore or at more exposed sites. However, the slowest recovering sites (high shore and sheltered shores) are at the least risk of natural disturbance and often considered more ‘stable’ (Lewis, 1964) as they are less vulnerable to removal by wave action or wave driven logs. Continued disturbance will lead to a patchy distribution of mussels.
Recruitment of Mytilus edulis is often sporadic, occurring in unpredictable pulses (Seed & Suchanek, 1992), although persistent mussel beds can be maintained by relatively low levels or episodic recruitment (McGrorty et al., 1990). A good annual recruitment could result in rapid recovery (Holt et al., 1998). However, the unpredictable pattern of recruitment based on environmental conditions could result in recruitment taking much longer. For example, in the northern Wadden Sea, strong year classes (resulting from a good recruitment episode) that lead to the rejuvenation of blue mussel beds are rare and usually follow severe winters, even though mussel spawning and settlement are extended and occur throughout the year (Diederich, 2005). In the List tidal basin (northern Wadden Sea) a mass recruitment of mussels occurred in 1996 but had not been repeated by 2003 (the date of the study), i.e. for seven years (Diederich, 2005).
Recent studies provide more detailed insights into the restoration and recovery potential of Mytilus edulis beds. Large-scale restoration experiments in shallow subtidal habitats demonstrated that suitable attachment substratum is critical for persistence, particularly in physically exposed locations. Banke et al. (2024) relayed suspension-grown Mytilus edulis either directly onto bare sandy sediments or on coir nets as a proxy for secure attachment. Over 1.5 years of monitoring the net treatment maintained significantly higher coverage and biomass, highlighting the dual importance of substratum and protection from dislodgement. However, regardless of treatment, high juvenile mortality (almost complete loss of individuals <30 mm within the first season), likely due to predation, rendered the populations unable to maintain themselves long-term (Banke et al., 2024). Similarly, Capelle et al. (2019) found that in high-energy environments (approx. 0.6 m/s), 100% of juveniles were dislodged in the absence of additional shell layers, though denser mussel aggregations reduced losses. Christensen et al. (2015) further demonstrated that complex substrata enhanced early bed formation, reducing mussel loss by approx. threefold within the first two days compared to smooth substrata, although this was associated with slightly slower growth rates.
In some long-term studies of Mytilus californianus gaps could continue to increase in size post-disturbance due to wave action and predation (Paine & Levin, 1981; Brosnan & Crumrine, 1994; Smith & Murray, 2005) potentially due to the weakening of the byssus threads leaving them more vulnerable to environmental conditions (Denny, 1987). On rocky shores, barnacles and fucoids are often quick to colonize the ‘gaps’ created. The presence of macroalgae appears to inhibit recovery whilst the presence of barnacles enhances subsequent mussel recruitment (Seed & Suchanek, 1992). Brosnan & Crumrine (1994) observed little recovery of the congener Mytilus californianus in two years after trampling disturbance. Paine & Levin (1981) estimated that recovery times of beds could be between 8 and 24 years while Seed & Suchanek (1992) suggested it could take longer-time scales, suggesting that meaningful recovery was unlikely in some areas. It has, however, been suggested that Mytilus edulis recovers quicker than other Mytilus species (Seed & Suchanek 1992), which may mean that these predicted recovery rates are too low for Mytilus edulis.
Patches of Mytilus edulis have been shown to recover faster than full, homogenous mussel beds (Van de Koppel et al., 2005; Liu et al., 2014). It is suggested that patchiness reduces competition for food and allows mussels to grow into the surrounding empty space after disturbances. Liu et al. (2014) showed that the greater the spatial complexity of a mussel bed, the faster it recovers from disturbance. Homogenous beds with no self-organisation showed the slowest recovery time (20 to 25 days) after a 30% reduction in density. Beds with only small-scale clusters recovered slightly faster, followed by those with only large-scale banded patterns, The fastest recovery (within 48 hours) occurred in the nested pattern where both small- and large-scale processes interact. In this case, fine-scale clustering helps mussels rapidly increase local density after disturbance, which then facilitates the re-establishment of the larger-scale banded structures.
Resilience Assessment
Alaria esculenta is an opportunistic and rapidly colonizing species capable of growing 20 cm/month in optimal conditions, reaching maturity within 10 to 14 months, and often appearing early in the algal succession (approx. 3 months after clearance of dominant algae). In canopy removal experiments in the Isle of Man, Hawkins & Harkin (1985) found that in moderately exposed areas cleared of Laminaria digitata, Alaria esculenta became the dominant canopy algae within nine months. Hence, the Alaria canopy would probably recover within <2 years (‘High’ resilience).
Mytilus spp. populations are considered to have a strong ability to recover from environmental disturbance (Holt et al., 1998; Seed & Suchanek, 1992). Good annual recruitment may allow a bed to recover rapidly, though this cannot always be guaranteed within a certain time scale due to the episodic nature of Mytilus edulis recruitment (Lutz & Kennish, 1992; Seed & Suchanek, 1992) and the influence of site-specific variables. While Mytilus is recorded as ‘Common’ in the understory turf of KFaR.Ala, ‘Frequent’ in KFaR.Ala.Ldig, and ‘Abundant’ as dense patches of small individuals in KFaR.Ala.Myt, it does not form beds in these biotopes (JNCC, 2022). Therefore, the patches of small individuals probably represent single recruitment events, where larger individuals are removed by wave action. Where KFaR.Ala.Myt occurs below the mussel-barnacle zone (MytB), recruitment may be rapid. However, given the sporadic nature of its recruitment they may recover from loss within one year or significantly longer (‘Medium’ resilience). Nevertheless, the KFaR.Ala and KFaR.Ala.Myt biotopes would be recognisable once the Alaria canopy recovered its abundance. Therefore, resilience is assessed as ‘High’ (<2 years) even though some members of the understory community (inc. Mytilus) could take longer to recover their prior abundance.
Note. The resilience and the ability to recover from human induced pressures is a combination of the environmental conditions of the site, the frequency (repeated disturbances versus a one-off event) and the intensity of the disturbance. Recovery of impacted populations will always be mediated by stochastic events and processes acting over different scales including, but not limited to, local habitat conditions, further impacts and processes such as larval supply and recruitment between populations. Full recovery is defined as the return to the state of the habitat that existed prior to impact. This does not necessarily mean that every component species has returned to its prior condition, abundance, or extent but that the relevant functional components are present and the habitat is structurally and functionally recognizable as the initial habitat of interest. It should be noted that the recovery rates are only indicative of the recovery potential.
Climate Change Pressures
Use [show more] / [show less] to open/close text displayed
| Resistance | Resilience | Sensitivity | |
Global warming (extreme) [Show more]Global warming (extreme)Extreme emission scenario (by the end of this century 2081-2100) benchmark of:
EvidenceAlaria esculentaThe distribution of seaweeds is climatically defined (Kain, 1979, Van Den Hoek, 1982, Breeman, 1990, Lüning, 1990). Northern boundaries are set by winter temperatures that are lethal or summer temperatures too low for growth and/or reproduction, whilst southern limits are set by high lethal summer temperatures or winter temperatures too high for induction of a crucial step in the life cycle (Breeman, 1990). Kelps have a high dependence on ocean temperatures, which makes them highly vulnerable to ocean warming (Assis et al., 2014). As temperatures increase, populations found towards the upper limit of their temperature range may be adversely affected by warming as physiological thresholds are exceeded (Wiens, 2016). Thermal stress can lead to mortality and consequent population-level effects, such as decreased abundance, altered size structure, local extinction and range contractions (Smale, 2020). Alaria esculenta is a polar to cold-temperate species that has been recorded from Brittany, France to Northern Norway (Birkett et al., 1998b). Sea temperature regulates metabolism and reproduction and defines the regional distribution of Alaria esculenta (Fredersdorf et al., 2009). The southern limit of Alaria esculenta has been defined at the 20°C isotherm (Munda & Lüning, 1977; Fredersdorf et al., 2009). However, it is more common north of the 16°C isotherm (Munda & Lüning, 1977; Van Den Hoek, 1982). As a result of this upper temperature threshold, Alaria esculenta is largely absent from the southern North Sea and English Channel where summer temperatures exceed 16°C and has already shown signs of contracting its range in the UK as a result of ocean warming (Mieszkowska, 2016). Munda & Lüning (1977) observed that temperatures of 16 to 17°C, sustained over 2 weeks in Helgoland, Germany, were lethal to resident Alaria esculenta. Experimental observations showed that acute exposure to ≥21°C is lethal to Alaria esculenta causing bleaching and disintegration (Sundene, 1962; Fredersdorf et al., 2009). At its northern range edge (Svalbard), it is a prominent macroalga on sublittoral fringe bedrock. At these northern latitudes, average summer temperature can reach 5°C, with an average annual sea temperature of 3°C (1980-2014, Beszczynska-Möller & Dye, 2013). Experimental observations conducted by Fredersdorf et al. (2009) found the optimal temperature for sporophyte photosynthesis was within the range of 13 to 17°C but the optimal temperature for Alaria esculenta germination was 2 to 12°C (Fredersdorf et al., 2009). Alaria esculenta is nearing its southern limits in the UK, with this species only occurring as far south as Brittany, France. Sea surface temperatures (SST) around the UK currently fall between 6 to 19°C (Huthnance, 2010). The available evidence suggests that the effects of ocean warming may occur throughout the year. If winter temperatures exceed 12°C this is likely to inhibit germination, whilst summer temperatures greater than 20°C will cause mortality of Alaria esculenta. Yesson et al. (2015) reported no significant change in Alaria esculenta abundance in the UK from 1974 to 2010, and no relationship between abundance and summer and winter sea surface temperatures. Despite this, they noted the contrast between their findings and those of previous research that reported declines in Alaria esculenta around the UK and Ireland, and suggested that if temperatures increase in the future, then abundances could change. Mytilus edulisMytilus edulis is a eurytopic species found in a wide temperature range from mild, subtropical regions to areas that frequently experience freezing conditions and are vulnerable to ice scour (Seed & Suchanek, 1992). In the north Atlantic, this species occurs from Norway to the coast of Spain. In the western Atlantic, Mytilus edulis has been observed to be expanding its range pole-wards and has reappeared in Svalbard, due to an increase in sea temperature in that region (Berge et al., 2005), whilst its equatorial limits have contracted approximately 350 km north of its previous southern limits in Cape Hatteras, North Carolina, due to increases in water temperature beyond the lethal limit (Jones et al., 2009). Wells & Gray (1960) suggested that the mean summer water temperatures of 26.6 °C set the southern range limit. Gonzalez & Yevich (1976) found that Mytilus edulis could not tolerate sustained temperatures of 27°C, and feeding stopped after 25°C. Pearce (1969) found that whilst some populations of Mytilus edulis could survive at 27°C for over a month, none of these populations could survive temperatures of 28°C for more than four days. Read & Cummings (1967) estimated the upper tolerance limit to be 27°C, and Chapple et al. (1998) found that Mytilus edulis could not acclimate to temperatures above 28.5°C. Almada-Villela et al. (1982) found that growth significantly declined in juvenile Mytilus edulis as temperatures increased above 20°C. Similarly, Hiebenthal et al. (2013) found that the growth rate decreased by 60% as temperatures increased from 20 - 25°C and resulted in 25% mortality under experimental conditions. Incze et al. (1980) found that Mytilus edulis growth decreased at 20°C and mortality occurred at 25°C, although mortality occurred at lower temperatures when phytoplankton abundance was low, suggesting that mortality occurred through a combination of reducing food source at a time of metabolic stress. Lethal water temperatures appear to vary between areas (Tsuchiya, 1983) and it appears that tolerance varies, depending on the temperature range to which the individuals are acclimatised (Kittner & Riisgaard, 2005). After acclimation of individuals of Mytilus edulis to 18°C, Kittner & Riisgaard (2005) observed that the filtration rates were at their maximum between 8.3 and 20°C and below this at 6°C the mussels closed their valves. However, after acclimation at 11°C for five days, the mussels maintained the high filtration rates down to 4°C. Hence, given time, mussels can acclimatise, shifting their temperature tolerance. Rising air temperatures can also lead to significant mortality in Mytilus edulis. Intertidal ecosystems are likely to be more negatively impacted than subtidal ecosystems, due to their increased daily and seasonal variations in temperatures (Jones et al., 2009). Tsuchiya (1983) documented the mass mortality of Mytilus edulis in August 1981 due to air temperatures of 34°C that resulted in mussel tissue temperatures over 40°C. In one hour, 50% of the Mytilus edulis from the upper 75% of the shore had died. It could not be concluded from this study whether the mortality was due to high temperatures, desiccation or a combination of the two. Under experimental conditions, exposure to air temperatures greater than 30°C led to significant mortality (Jones et al., 2009), suggesting this may be an upper temperature threshold for this species. At the upper range of a mussel’s tolerance limit, heat shock proteins are produced, indicating high stress levels (Jones et al., 2010). After a single day at 30°C, heat shock proteins were still present over 14 days later, although at a reduced level. Increased temperatures can also affect reproduction in Mytilus edulis (Myrand et al., 2000). In shallow lagoons, mortality began in late July at the end of a major spawning event when temperatures peaked at >20°C. These mussels had a low energetic content post-spawning and had stopped shell growth. The high temperatures likely caused mortality due to the reduced condition of the mussels post-spawning (Myrand et al., 2000). Gamete production does not appear to be affected by temperature (Suchanek, 1985). Temperature changes may also lead to indirect effects. For example, an increase in temperature increases the mussels’ susceptibility to pathogens (Vibrio tubiashii) in the presence of relatively low concentrations of copper (Parry & Pipe, 2004). Increased temperatures may also allow for range expansion of parasites or pathogens which will have a negative impact upon the health of the mussels if they become infected. There is evidence that increases in temperature will also give a competitive advantage to invasive species. For example, in the Dutch Wadden Sea mild winters favour Magallana gigas recruitment while cold winters favour Mytilus edulis (Deiderich, 2005). Sensitivity AssessmentAlaria esculenta is competitively inferior to Laminaria digitata in the northeast Atlantic (Hawkins & Harkin, 1985) where it is confined to more exposed shores and can colonize sheltered environments only if Laminaria digitata is removed. As temperatures rise to up to 20°C, it is expected that the competitive ability of this species will decrease further, and Alaria esculenta will be lost, with more warm-adapted algae taking their place. Brodie et al. (2014) predict that Alaria esculenta will be completely lost from Boreal habitats by the end of this century, whilst all kelp species will be lost from the Lusitanian region, replaced by smaller, fleshy algae. Mytilus edulis is a eurythermal species, and the maximum upper thermal limit of this species appears to generally be somewhere between 25 to 28°C, above which this species experiences mortality, with tolerance related to exposure. As ocean warming will occur gradually, across the course of this century, it is expected that this species will be able to withstand these increases in temperature. As this species is intertidal, it will also have to cope with increases air temperature. In July, temperatures can reach up to an average of 25°C in the south of the UK, although the highest temperature recorded 1961-2010 was 38.5°C (Perry & Golding, 2011). If air temperatures rise by 3, 4, and 6°C by the end of the century (middle and high emission and extreme scenarios, respectively), this could lead to temperatures reaching average summer high temperatures of between 28 to 31°C. Sea surface temperatures around the UK are currently between 6 to 19°C (Huthnance, 2010). Under the middle emission scenario, Alaria esculenta is likely to be lost from most of the UK, although it may manage to maintain some populations in Scotland, where current summer temperatures often reach 14°C, leading to potential summer temperatures of 17°C. Therefore, resistance is assessed as ‘Low’ and resilience as ‘Very Low’, as the loss is likely to be a long-term decline, due to the long-term nature of ocean warming. Therefore, this biotope is assessed as having ‘High’ sensitivity to ocean warming under a middle emission scenario. For the high emission scenario and extreme scenario, sea temperatures may rise by 4 to 5°C to give potential southern summer temperatures of 23 to 24°C and northern summer temperatures of 18 to 19°C. Under these scenarios, it is likely that Alaria esculenta will be lost almost completely from the UK. Therefore, resistance is assessed as ‘None’, and resilience is assessed as ‘Very low’. Overall, this biotope is assessed as having ‘High’ sensitivity to ocean warming for the high emission scenario and the extreme scenario. | NoneHelp | Very LowHelp | HighHelp |
Global warming (high) [Show more]Global warming (high)High emission scenario (by the end of this century 2081-2100) benchmark of:
EvidenceAlaria esculentaThe distribution of seaweeds is climatically defined (Kain, 1979, Van Den Hoek, 1982, Breeman, 1990, Lüning, 1990). Northern boundaries are set by winter temperatures that are lethal or summer temperatures too low for growth and/or reproduction, whilst southern limits are set by high lethal summer temperatures or winter temperatures too high for induction of a crucial step in the life cycle (Breeman, 1990). Kelps have a high dependence on ocean temperatures, which makes them highly vulnerable to ocean warming (Assis et al., 2014). As temperatures increase, populations found towards the upper limit of their temperature range may be adversely affected by warming as physiological thresholds are exceeded (Wiens, 2016). Thermal stress can lead to mortality and consequent population-level effects, such as decreased abundance, altered size structure, local extinction and range contractions (Smale, 2020). Alaria esculenta is a polar to cold-temperate species that has been recorded from Brittany, France to Northern Norway (Birkett et al., 1998b). Sea temperature regulates metabolism and reproduction and defines the regional distribution of Alaria esculenta (Fredersdorf et al., 2009). The southern limit of Alaria esculenta has been defined at the 20°C isotherm (Munda & Lüning, 1977; Fredersdorf et al., 2009). However, it is more common north of the 16°C isotherm (Munda & Lüning, 1977; Van Den Hoek, 1982). As a result of this upper temperature threshold, Alaria esculenta is largely absent from the southern North Sea and English Channel where summer temperatures exceed 16°C and has already shown signs of contracting its range in the UK as a result of ocean warming (Mieszkowska, 2016). Munda & Lüning (1977) observed that temperatures of 16 to 17°C, sustained over 2 weeks in Helgoland, Germany, were lethal to resident Alaria esculenta. Experimental observations showed that acute exposure to ≥21°C is lethal to Alaria esculenta causing bleaching and disintegration (Sundene, 1962; Fredersdorf et al., 2009). At its northern range edge (Svalbard), it is a prominent macroalga on sublittoral fringe bedrock. At these northern latitudes, average summer temperature can reach 5°C, with an average annual sea temperature of 3°C (1980-2014, Beszczynska-Möller & Dye, 2013). Experimental observations conducted by Fredersdorf et al. (2009) found the optimal temperature for sporophyte photosynthesis was within the range of 13 to 17°C but the optimal temperature for Alaria esculenta germination was 2 to 12°C (Fredersdorf et al., 2009). Alaria esculenta is nearing its southern limits in the UK, with this species only occurring as far south as Brittany, France. Sea surface temperatures (SST) around the UK currently fall between 6 to 19°C (Huthnance, 2010). The available evidence suggests that the effects of ocean warming may occur throughout the year. If winter temperatures exceed 12°C this is likely to inhibit germination, whilst summer temperatures greater than 20°C will cause mortality of Alaria esculenta. Yesson et al. (2015) reported no significant change in Alaria esculenta abundance in the UK from 1974 to 2010, and no relationship between abundance and summer and winter sea surface temperatures. Despite this, they noted the contrast between their findings and those of previous research that reported declines in Alaria esculenta around the UK and Ireland, and suggested that if temperatures increase in the future, then abundances could change. Mytilus edulisMytilus edulis is a eurytopic species found in a wide temperature range from mild, subtropical regions to areas that frequently experience freezing conditions and are vulnerable to ice scour (Seed & Suchanek, 1992). In the north Atlantic, this species occurs from Norway to the coast of Spain. In the western Atlantic, Mytilus edulis has been observed to be expanding its range pole-wards and has reappeared in Svalbard, due to an increase in sea temperature in that region (Berge et al., 2005), whilst its equatorial limits have contracted approximately 350 km north of its previous southern limits in Cape Hatteras, North Carolina, due to increases in water temperature beyond the lethal limit (Jones et al., 2009). Wells & Gray (1960) suggested that the mean summer water temperatures of 26.6 °C set the southern range limit. Gonzalez & Yevich (1976) found that Mytilus edulis could not tolerate sustained temperatures of 27°C, and feeding stopped after 25°C. Pearce (1969) found that whilst some populations of Mytilus edulis could survive at 27°C for over a month, none of these populations could survive temperatures of 28°C for more than four days. Read & Cummings (1967) estimated the upper tolerance limit to be 27°C, and Chapple et al. (1998) found that Mytilus edulis could not acclimate to temperatures above 28.5°C. Almada-Villela et al. (1982) found that growth significantly declined in juvenile Mytilus edulis as temperatures increased above 20°C. Similarly, Hiebenthal et al. (2013) found that the growth rate decreased by 60% as temperatures increased from 20 - 25°C and resulted in 25% mortality under experimental conditions. Incze et al. (1980) found that Mytilus edulis growth decreased at 20°C and mortality occurred at 25°C, although mortality occurred at lower temperatures when phytoplankton abundance was low, suggesting that mortality occurred through a combination of reducing food source at a time of metabolic stress. Lethal water temperatures appear to vary between areas (Tsuchiya, 1983) and it appears that tolerance varies, depending on the temperature range to which the individuals are acclimatised (Kittner & Riisgaard, 2005). After acclimation of individuals of Mytilus edulis to 18°C, Kittner & Riisgaard (2005) observed that the filtration rates were at their maximum between 8.3 and 20°C and below this at 6°C the mussels closed their valves. However, after acclimation at 11°C for five days, the mussels maintained the high filtration rates down to 4°C. Hence, given time, mussels can acclimatise, shifting their temperature tolerance. Rising air temperatures can also lead to significant mortality in Mytilus edulis. Intertidal ecosystems are likely to be more negatively impacted than subtidal ecosystems, due to their increased daily and seasonal variations in temperatures (Jones et al., 2009). Tsuchiya (1983) documented the mass mortality of Mytilus edulis in August 1981 due to air temperatures of 34°C that resulted in mussel tissue temperatures over 40°C. In one hour, 50% of the Mytilus edulis from the upper 75% of the shore had died. It could not be concluded from this study whether the mortality was due to high temperatures, desiccation or a combination of the two. Under experimental conditions, exposure to air temperatures greater than 30°C led to significant mortality (Jones et al., 2009), suggesting this may be an upper temperature threshold for this species. At the upper range of a mussel’s tolerance limit, heat shock proteins are produced, indicating high stress levels (Jones et al., 2010). After a single day at 30°C, heat shock proteins were still present over 14 days later, although at a reduced level. Increased temperatures can also affect reproduction in Mytilus edulis (Myrand et al., 2000). In shallow lagoons, mortality began in late July at the end of a major spawning event when temperatures peaked at >20°C. These mussels had a low energetic content post-spawning and had stopped shell growth. The high temperatures likely caused mortality due to the reduced condition of the mussels post-spawning (Myrand et al., 2000). Gamete production does not appear to be affected by temperature (Suchanek, 1985). Temperature changes may also lead to indirect effects. For example, an increase in temperature increases the mussels’ susceptibility to pathogens (Vibrio tubiashii) in the presence of relatively low concentrations of copper (Parry & Pipe, 2004). Increased temperatures may also allow for range expansion of parasites or pathogens which will have a negative impact upon the health of the mussels if they become infected. There is evidence that increases in temperature will also give a competitive advantage to invasive species. For example, in the Dutch Wadden Sea mild winters favour Magallana gigas recruitment while cold winters favour Mytilus edulis (Deiderich, 2005). Sensitivity AssessmentAlaria esculenta is competitively inferior to Laminaria digitata in the northeast Atlantic (Hawkins & Harkin, 1985) where it is confined to more exposed shores and can colonize sheltered environments only if Laminaria digitata is removed. As temperatures rise to up to 20°C, it is expected that the competitive ability of this species will decrease further, and Alaria esculenta will be lost, with more warm-adapted algae taking their place. Brodie et al. (2014) predict that Alaria esculenta will be completely lost from Boreal habitats by the end of this century, whilst all kelp species will be lost from the Lusitanian region, replaced by smaller, fleshy algae. Mytilus edulis is a eurythermal species, and the maximum upper thermal limit of this species appears to generally be somewhere between 25 to 28°C, above which this species experiences mortality, with tolerance related to exposure. As ocean warming will occur gradually, across the course of this century, it is expected that this species will be able to withstand these increases in temperature. As this species is intertidal, it will also have to cope with increases air temperature. In July, temperatures can reach up to an average of 25°C in the south of the UK, although the highest temperature recorded 1961-2010 was 38.5°C (Perry & Golding, 2011). If air temperatures rise by 3, 4, and 6°C by the end of the century (middle and high emission and extreme scenarios, respectively), this could lead to temperatures reaching average summer high temperatures of between 28 to 31°C. Sea surface temperatures around the UK are currently between 6 to 19°C (Huthnance, 2010). Under the middle emission scenario, Alaria esculenta is likely to be lost from most of the UK, although it may manage to maintain some populations in Scotland, where current summer temperatures often reach 14°C, leading to potential summer temperatures of 17°C. Therefore, resistance is assessed as ‘Low’ and resilience as ‘Very Low’, as the loss is likely to be a long-term decline, due to the long-term nature of ocean warming. Therefore, this biotope is assessed as having ‘High’ sensitivity to ocean warming under a middle emission scenario. For the high emission scenario and extreme scenario, sea temperatures may rise by 4 to 5°C to give potential southern summer temperatures of 23 to 24°C and northern summer temperatures of 18 to 19°C. Under these scenarios, it is likely that Alaria esculenta will be lost almost completely from the UK. Therefore, resistance is assessed as ‘None’, and resilience is assessed as ‘Very low’. Overall, this biotope is assessed as having ‘High’ sensitivity to ocean warming for the high emission scenario and the extreme scenario. | NoneHelp | Very LowHelp | HighHelp |
Global warming (middle) [Show more]Global warming (middle)Middle emission scenario (by the end of this century 2081-2100) benchmark of:
EvidenceAlaria esculentaThe distribution of seaweeds is climatically defined (Kain, 1979, Van Den Hoek, 1982, Breeman, 1990, Lüning, 1990). Northern boundaries are set by winter temperatures that are lethal or summer temperatures too low for growth and/or reproduction, whilst southern limits are set by high lethal summer temperatures or winter temperatures too high for induction of a crucial step in the life cycle (Breeman, 1990). Kelps have a high dependence on ocean temperatures, which makes them highly vulnerable to ocean warming (Assis et al., 2014). As temperatures increase, populations found towards the upper limit of their temperature range may be adversely affected by warming as physiological thresholds are exceeded (Wiens, 2016). Thermal stress can lead to mortality and consequent population-level effects, such as decreased abundance, altered size structure, local extinction and range contractions (Smale, 2020). Alaria esculenta is a polar to cold-temperate species that has been recorded from Brittany, France to Northern Norway (Birkett et al., 1998b). Sea temperature regulates metabolism and reproduction and defines the regional distribution of Alaria esculenta (Fredersdorf et al., 2009). The southern limit of Alaria esculenta has been defined at the 20°C isotherm (Munda & Lüning, 1977; Fredersdorf et al., 2009). However, it is more common north of the 16°C isotherm (Munda & Lüning, 1977; Van Den Hoek, 1982). As a result of this upper temperature threshold, Alaria esculenta is largely absent from the southern North Sea and English Channel where summer temperatures exceed 16°C and has already shown signs of contracting its range in the UK as a result of ocean warming (Mieszkowska, 2016). Munda & Lüning (1977) observed that temperatures of 16 to 17°C, sustained over 2 weeks in Helgoland, Germany, were lethal to resident Alaria esculenta. Experimental observations showed that acute exposure to ≥21°C is lethal to Alaria esculenta causing bleaching and disintegration (Sundene, 1962; Fredersdorf et al., 2009). At its northern range edge (Svalbard), it is a prominent macroalga on sublittoral fringe bedrock. At these northern latitudes, average summer temperature can reach 5°C, with an average annual sea temperature of 3°C (1980-2014, Beszczynska-Möller & Dye, 2013). Experimental observations conducted by Fredersdorf et al. (2009) found the optimal temperature for sporophyte photosynthesis was within the range of 13 to 17°C but the optimal temperature for Alaria esculenta germination was 2 to 12°C (Fredersdorf et al., 2009). Alaria esculenta is nearing its southern limits in the UK, with this species only occurring as far south as Brittany, France. Sea surface temperatures (SST) around the UK currently fall between 6 to 19°C (Huthnance, 2010). The available evidence suggests that the effects of ocean warming may occur throughout the year. If winter temperatures exceed 12°C this is likely to inhibit germination, whilst summer temperatures greater than 20°C will cause mortality of Alaria esculenta. Yesson et al. (2015) reported no significant change in Alaria esculenta abundance in the UK from 1974 to 2010, and no relationship between abundance and summer and winter sea surface temperatures. Despite this, they noted the contrast between their findings and those of previous research that reported declines in Alaria esculenta around the UK and Ireland, and suggested that if temperatures increase in the future, then abundances could change. Mytilus edulisMytilus edulis is a eurytopic species found in a wide temperature range from mild, subtropical regions to areas that frequently experience freezing conditions and are vulnerable to ice scour (Seed & Suchanek, 1992). In the north Atlantic, this species occurs from Norway to the coast of Spain. In the western Atlantic, Mytilus edulis has been observed to be expanding its range pole-wards and has reappeared in Svalbard, due to an increase in sea temperature in that region (Berge et al., 2005), whilst its equatorial limits have contracted approximately 350 km north of its previous southern limits in Cape Hatteras, North Carolina, due to increases in water temperature beyond the lethal limit (Jones et al., 2009). Wells & Gray (1960) suggested that the mean summer water temperatures of 26.6 °C set the southern range limit. Gonzalez & Yevich (1976) found that Mytilus edulis could not tolerate sustained temperatures of 27°C, and feeding stopped after 25°C. Pearce (1969) found that whilst some populations of Mytilus edulis could survive at 27°C for over a month, none of these populations could survive temperatures of 28°C for more than four days. Read & Cummings (1967) estimated the upper tolerance limit to be 27°C, and Chapple et al. (1998) found that Mytilus edulis could not acclimate to temperatures above 28.5°C. Almada-Villela et al. (1982) found that growth significantly declined in juvenile Mytilus edulis as temperatures increased above 20°C. Similarly, Hiebenthal et al. (2013) found that the growth rate decreased by 60% as temperatures increased from 20 - 25°C and resulted in 25% mortality under experimental conditions. Incze et al. (1980) found that Mytilus edulis growth decreased at 20°C and mortality occurred at 25°C, although mortality occurred at lower temperatures when phytoplankton abundance was low, suggesting that mortality occurred through a combination of reducing food source at a time of metabolic stress. Lethal water temperatures appear to vary between areas (Tsuchiya, 1983) and it appears that tolerance varies, depending on the temperature range to which the individuals are acclimatised (Kittner & Riisgaard, 2005). After acclimation of individuals of Mytilus edulis to 18°C, Kittner & Riisgaard (2005) observed that the filtration rates were at their maximum between 8.3 and 20°C and below this at 6°C the mussels closed their valves. However, after acclimation at 11°C for five days, the mussels maintained the high filtration rates down to 4°C. Hence, given time, mussels can acclimatise, shifting their temperature tolerance. Rising air temperatures can also lead to significant mortality in Mytilus edulis. Intertidal ecosystems are likely to be more negatively impacted than subtidal ecosystems, due to their increased daily and seasonal variations in temperatures (Jones et al., 2009). Tsuchiya (1983) documented the mass mortality of Mytilus edulis in August 1981 due to air temperatures of 34°C that resulted in mussel tissue temperatures over 40°C. In one hour, 50% of the Mytilus edulis from the upper 75% of the shore had died. It could not be concluded from this study whether the mortality was due to high temperatures, desiccation or a combination of the two. Under experimental conditions, exposure to air temperatures greater than 30°C led to significant mortality (Jones et al., 2009), suggesting this may be an upper temperature threshold for this species. At the upper range of a mussel’s tolerance limit, heat shock proteins are produced, indicating high stress levels (Jones et al., 2010). After a single day at 30°C, heat shock proteins were still present over 14 days later, although at a reduced level. Increased temperatures can also affect reproduction in Mytilus edulis (Myrand et al., 2000). In shallow lagoons, mortality began in late July at the end of a major spawning event when temperatures peaked at >20°C. These mussels had a low energetic content post-spawning and had stopped shell growth. The high temperatures likely caused mortality due to the reduced condition of the mussels post-spawning (Myrand et al., 2000). Gamete production does not appear to be affected by temperature (Suchanek, 1985). Temperature changes may also lead to indirect effects. For example, an increase in temperature increases the mussels’ susceptibility to pathogens (Vibrio tubiashii) in the presence of relatively low concentrations of copper (Parry & Pipe, 2004). Increased temperatures may also allow for range expansion of parasites or pathogens which will have a negative impact upon the health of the mussels if they become infected. There is evidence that increases in temperature will also give a competitive advantage to invasive species. For example, in the Dutch Wadden Sea mild winters favour Magallana gigas recruitment while cold winters favour Mytilus edulis (Deiderich, 2005). Sensitivity AssessmentAlaria esculenta is competitively inferior to Laminaria digitata in the northeast Atlantic (Hawkins & Harkin, 1985) where it is confined to more exposed shores and can colonize sheltered environments only if Laminaria digitata is removed. As temperatures rise to up to 20°C, it is expected that the competitive ability of this species will decrease further, and Alaria esculenta will be lost, with more warm-adapted algae taking their place. Brodie et al. (2014) predict that Alaria esculenta will be completely lost from Boreal habitats by the end of this century, whilst all kelp species will be lost from the Lusitanian region, replaced by smaller, fleshy algae. Mytilus edulis is a eurythermal species, and the maximum upper thermal limit of this species appears to generally be somewhere between 25 to 28°C, above which this species experiences mortality, with tolerance related to exposure. As ocean warming will occur gradually, across the course of this century, it is expected that this species will be able to withstand these increases in temperature. As this species is intertidal, it will also have to cope with increases air temperature. In July, temperatures can reach up to an average of 25°C in the south of the UK, although the highest temperature recorded 1961-2010 was 38.5°C (Perry & Golding, 2011). If air temperatures rise by 3, 4, and 6°C by the end of the century (middle and high emission and extreme scenarios, respectively), this could lead to temperatures reaching average summer high temperatures of between 28 to 31°C. Sea surface temperatures around the UK are currently between 6 to 19°C (Huthnance, 2010). Under the middle emission scenario, Alaria esculenta is likely to be lost from most of the UK, although it may manage to maintain some populations in Scotland, where current summer temperatures often reach 14°C, leading to potential summer temperatures of 17°C. Therefore, resistance is assessed as ‘Low’ and resilience as ‘Very Low’, as the loss is likely to be a long-term decline, due to the long-term nature of ocean warming. Therefore, this biotope is assessed as having ‘High’ sensitivity to ocean warming under a middle emission scenario. For the high emission scenario and extreme scenario, sea temperatures may rise by 4 to 5°C to give potential southern summer temperatures of 23 to 24°C and northern summer temperatures of 18 to 19°C. Under these scenarios, it is likely that Alaria esculenta will be lost almost completely from the UK. Therefore, resistance is assessed as ‘None’, and resilience is assessed as ‘Very low’. Overall, this biotope is assessed as having ‘High’ sensitivity to ocean warming for the high emission scenario and the extreme scenario. | LowHelp | Very LowHelp | HighHelp |
Marine heatwaves (high) [Show more]Marine heatwaves (high)High emission scenario benchmark: A marine heatwave occurring every two years, with a mean duration of 120 days, and a maximum intensity of 3.5°C (Marine heatwave pressure definitions). EvidenceAlaria esculentaLebrun et al. (2025) studied marine heatwave (MHW) effects on three kelp species including Alaria esculenta. In their mesocosm experiment, water flow was supplied directly from the ocean, ensuring that the control treatment reflected natural conditions. Control temperatures ranged from approx. 7.5 to 10°C. Additional treatments included a constant high-temperature treatment (HT; +1.8°C above control), a single 13-day MHW treatment (1MH; +2.8°C above control), and a treatment simulating two consecutive 5-day MHWs (2MH; +3.9°C above control). No mortality was reported, but physiological responses varied. Net photosynthetic rates declined significantly between the beginning and end of the experiment in all treatments, with a significant decline occurring by the midpoint of the experiment in the HT treatment. Photosynthetic efficiency (FV/FM) remained above 0.7 throughout, indicating good physiological condition. Chlorophyll-a content differed significantly between the beginning and end of the experiment only in the 2MH treatment, while significant differences in C:N ratios were detected only between the 1MH and 2MH treatments at the end of the experiment. Growth rates did not differ among treatments. Overall, these findings suggest that Alaria esculenta remained physiologically healthy and maintained growth under the simulated MHW conditions, although some changes in photosynthetic performance, pigmentation, and C:N ratios occurred. Mytilus edulisMarine heatwaves due to increased air-sea heat flux are predicted to occur more frequently, at an increased intensity and last for longer by the end of this century under both middle and high emission scenarios (Frölicher et al., 2018). Intertidal populations of Mytilus edulis may be particularly sensitive to marine heatwaves. When submerged, a mussel’s body temperature closely approximates that of the surrounding water, whereas when emerged, body temperatures can become much higher than the surrounding air or substratum (Zippay & Helmuth, 2012). In the southern portion of its range in the USA, intertidal populations of Mytilus edulis have experienced catastrophic mortality directly associated with summer high temperatures of up to 32°C, with populations shifting their range 350 km northwards of their previous range (Jones et al., 2009). Transcriptomic and proteomic studies across multiple regions indicate that adult mussels can tolerate short-term warming to at least 27 to 30°C with limited cellular stress responses. Greenland populations showed minimal transcriptional disruption even at 32°C, indicating a broad capacity for acclimation across thermal histories (mussels were collected at 27, 19, and 3°C; Clark et al., 2021). Similarly, mussels from the remote, sub-Antarctic Kerguelen Archipelago exposed to rapid warming from 7.5 to 20°C exhibited a typical but controlled stress response consistent with conserved protein homeostasis mechanisms rather than acute physiological failure (Bultelle et al., 2021). However, a number of experimental studies indicate that survival declines rapidly once upper thermal thresholds are exceeded, particularly under sustained exposure. Complete mortality has been observed after 3 to 32 days at 30°C, with faster mortality at higher temperatures and declining condition index prior to death (Kamermans & Saurel, 2022). Air temperatures tend to be more variable and extreme than seawater temperatures (Helmuth et al., 2002). While the south of the UK has a mean summer daily high temperature of 21°C, temperatures can often reach ≥30°C (Met Office, 2016). Temperature loggers on the west coast of Scotland recorded intertidal temperatures on the high shore exceeding 40°C in seven of the 11 years it was monitored (Burrows, 2017), which shows the extreme temperatures that intertidal species have to cope with, at present. Furthermore, when exposed to high daytime temperatures, internal body temperature can far exceed air temperatures. For example, when Mytilus edulis was exposed to air temperatures of up to 34°C on the shore, body temperatures of the mussels increased to 46°C, leading to mortality (Tsuchiya, 1983). Evidence from recent extreme heat events in north-west Europe demonstrates that mussels in UK-relevant biotopes can experience body temperatures substantially exceeding ambient seawater temperatures during calm, sunny conditions. Real-world heatwave observations show that intertidal mussel body temperatures frequently exceed 30°C for multiple consecutive days, with localised mass mortality recorded despite relatively moderate climatic heatwave conditions (Seuront et al., 2019; Talevi et al., 2023). The thermal tolerance of Mytilus edulis decreases under repeated heat stress, therefore this species is likely to be especially sensitive to both marine and aerial heatwaves (Seuront et al., 2019). Although some individuals and populations exhibit remarkable tolerance and recovery capacity, including enhanced thermal limits following prior heatwave exposure (King et al., 2024), cumulative heat stress can reduce feeding, condition and survival, particularly in shallow intertidal settings (Dereuder et al., 2025; Fly et al., 2015). In Japan, in 1981, mass mortality of Mytilus edulis occurred along a rocky shore as a result of unusually high temperatures, whilst another species of mussel (Mytilisepta virgatus) that occurred in the zone above Mytilus edulis exhibited much greater levels of heat tolerance and low mortality (Tsuchiya, 1983). Mytilus edulis is thought to be particularly susceptible to high temperatures and heatwaves in the summer, due to the low energy reserves of the organism after spawning (Tremblay et al., 1998, Myrand et al., 2000). Experimental marine heatwave simulations involving repeated +5°C warming events increased valve micro-closure frequency, indicating heightened stress, with some behavioural and molecular effects persisting beyond the recovery period (Grimmelpont et al., 2024). Field-based studies suggest that survival during extreme heat events is strongly influenced by microhabitat and biological context, with shell-associated endolithic microbial communities providing a measurable thermal buffering effect of up to 3.2°C and enhancing survival during the 2022 English Channel heatwave, particularly on the high shore where thermal pressure was greatest (Zardi et al., 2024). Dynamic and constant heatwave experiments further indicate that survival outcomes depend strongly on thermal regime. Vajedsamiei et al. (2024) found that under constant heatwave conditions, survival dropped to zero within seven days at 29°C and within 30 days at 28°C, whereas fluctuating (“dynamic”) heatwave regimes allowed partial survival at similar mean temperatures, highlighting the mitigating role of thermal variability. These findings suggest that while Mytilus edulis can tolerate brief exposure to extreme temperatures, sustained or repeated exposure leads to rapid mortality. Furthermore, evidence from both laboratory simulations and real-world heatwave events indicates that repeated exposure to elevated temperatures can progressively erode thermal tolerance, even when individual exposure events are sub-lethal. Repeated daily heat stress experiments reproducing body temperature profiles recorded during the 2018 English Channel heatwave demonstrated that thermal tolerance consistently declined with successive exposures, leading to increased mortality under otherwise moderate climatic conditions (Seuront et al., 2019). Elevated temperature can exacerbate the effects of other environmental pressures even where warming alone causes limited mortality. In a field-based experiment on the south coast of the UK, Greatorex & Knights (2023) recorded 6% mortality over eight weeks at both control (15°C) and elevated (20°C) temperatures. However, mortality increased to 23% when elevated temperature was combined with simulated ocean acidification, while no mortality occurred under acidification alone. Experimental work under controlled laboratory conditions supports this interaction. Li et al. (2015) exposed adult mussels to temperatures of 19, 22 and 25°C for two months and found that elevated temperature intensified the effects of ocean acidification, resulting in reduced calcification, lower shell calcium content, altered Ca/Mg ratios and downregulation of biomineralisation-related genes. Nutrient enrichment and thermal stress together have produced variable mortality responses depending on exposure timing (Carrier-Belleau et al., 2024). Sensitivity AssessmentUnder the middle emission scenario, if heatwaves occurred every three years, with a maximum intensity of 2°C for 80 days by the end of this century, this could lead to summer sea temperatures reaching up to 24°C in southern England and 19°C in Scotland. Under the middle emission scenario, Alaria esculenta is likely to be lost from the southern parts of the UK (see Global warming pressure). Any remaining populations of Alaria esculenta are likely to suffer severe mortality as a result of a heatwave of this magnitude. Mytilus edulis is thought to have an upper thermal limit of 25 to 28°C in water, although growth decreases at temperatures over 20°C. In addition, intertidal examples of this biotope may be exposed to air temperatures exceeding 30°C in this global warming scenario. Therefore, resistance has been assessed as ‘None’. As a further heatwave is likely to affect this habitat before full recovery, resilience has been assessed as ‘Low’. Therefore, this biotope is assessed as having ‘High’ sensitivity to marine heatwaves under the middle emission scenario. Under the high emission scenario, if heatwaves occur every two years by the end of this century, reaching a maximum intensity of 3.5°C for 120 days, this could lead to the heatwave lasting the entire summer with temperatures reaching up to 26.5°C in southern England and 21.5°C in Scotland. Intertidal examples of this biotope may experience air temperatures exceeding 30°C across much of the UK. Under the high emission scenario, Alaria esculenta is likely to be almost wiped out in the UK. Therefore, resistance has been assessed as ‘None’. As widespread mortality may lead to a lack of viable sporophytes for recruitment, resilience has been assessed as ‘Very low.’ Therefore, this biotope is assessed as having ‘High’ sensitivity to marine heatwaves under the high emission scenario. | NoneHelp | Very LowHelp | HighHelp |
Marine heatwaves (middle) [Show more]Marine heatwaves (middle)Middle emission scenario benchmark: A marine heatwave occurring every three years, with a mean duration of 80 days, with a maximum intensity of 2°C. EvidenceAlaria esculentaLebrun et al. (2025) studied marine heatwave (MHW) effects on three kelp species including Alaria esculenta. In their mesocosm experiment, water flow was supplied directly from the ocean, ensuring that the control treatment reflected natural conditions. Control temperatures ranged from approx. 7.5 to 10°C. Additional treatments included a constant high-temperature treatment (HT; +1.8°C above control), a single 13-day MHW treatment (1MH; +2.8°C above control), and a treatment simulating two consecutive 5-day MHWs (2MH; +3.9°C above control). No mortality was reported, but physiological responses varied. Net photosynthetic rates declined significantly between the beginning and end of the experiment in all treatments, with a significant decline occurring by the midpoint of the experiment in the HT treatment. Photosynthetic efficiency (FV/FM) remained above 0.7 throughout, indicating good physiological condition. Chlorophyll-a content differed significantly between the beginning and end of the experiment only in the 2MH treatment, while significant differences in C:N ratios were detected only between the 1MH and 2MH treatments at the end of the experiment. Growth rates did not differ among treatments. Overall, these findings suggest that Alaria esculenta remained physiologically healthy and maintained growth under the simulated MHW conditions, although some changes in photosynthetic performance, pigmentation, and C:N ratios occurred. Mytilus edulisMarine heatwaves due to increased air-sea heat flux are predicted to occur more frequently, at an increased intensity and last for longer by the end of this century under both middle and high emission scenarios (Frölicher et al., 2018). Intertidal populations of Mytilus edulis may be particularly sensitive to marine heatwaves. When submerged, a mussel’s body temperature closely approximates that of the surrounding water, whereas when emerged, body temperatures can become much higher than the surrounding air or substratum (Zippay & Helmuth, 2012). In the southern portion of its range in the USA, intertidal populations of Mytilus edulis have experienced catastrophic mortality directly associated with summer high temperatures of up to 32°C, with populations shifting their range 350 km northwards of their previous range (Jones et al., 2009). Transcriptomic and proteomic studies across multiple regions indicate that adult mussels can tolerate short-term warming to at least 27 to 30°C with limited cellular stress responses. Greenland populations showed minimal transcriptional disruption even at 32°C, indicating a broad capacity for acclimation across thermal histories (mussels were collected at 27, 19, and 3°C; Clark et al., 2021). Similarly, mussels from the remote, sub-Antarctic Kerguelen Archipelago exposed to rapid warming from 7.5 to 20°C exhibited a typical but controlled stress response consistent with conserved protein homeostasis mechanisms rather than acute physiological failure (Bultelle et al., 2021). However, a number of experimental studies indicate that survival declines rapidly once upper thermal thresholds are exceeded, particularly under sustained exposure. Complete mortality has been observed after 3 to 32 days at 30°C, with faster mortality at higher temperatures and declining condition index prior to death (Kamermans & Saurel, 2022). Air temperatures tend to be more variable and extreme than seawater temperatures (Helmuth et al., 2002). While the south of the UK has a mean summer daily high temperature of 21°C, temperatures can often reach ≥30°C (Met Office, 2016). Temperature loggers on the west coast of Scotland recorded intertidal temperatures on the high shore exceeding 40°C in seven of the 11 years it was monitored (Burrows, 2017), which shows the extreme temperatures that intertidal species have to cope with, at present. Furthermore, when exposed to high daytime temperatures, internal body temperature can far exceed air temperatures. For example, when Mytilus edulis was exposed to air temperatures of up to 34°C on the shore, body temperatures of the mussels increased to 46°C, leading to mortality (Tsuchiya, 1983). Evidence from recent extreme heat events in north-west Europe demonstrates that mussels in UK-relevant biotopes can experience body temperatures substantially exceeding ambient seawater temperatures during calm, sunny conditions. Real-world heatwave observations show that intertidal mussel body temperatures frequently exceed 30°C for multiple consecutive days, with localised mass mortality recorded despite relatively moderate climatic heatwave conditions (Seuront et al., 2019; Talevi et al., 2023). The thermal tolerance of Mytilus edulis decreases under repeated heat stress, therefore this species is likely to be especially sensitive to both marine and aerial heatwaves (Seuront et al., 2019). Although some individuals and populations exhibit remarkable tolerance and recovery capacity, including enhanced thermal limits following prior heatwave exposure (King et al., 2024), cumulative heat stress can reduce feeding, condition and survival, particularly in shallow intertidal settings (Dereuder et al., 2025; Fly et al., 2015). In Japan, in 1981, mass mortality of Mytilus edulis occurred along a rocky shore as a result of unusually high temperatures, whilst another species of mussel (Mytilisepta virgatus) that occurred in the zone above Mytilus edulis exhibited much greater levels of heat tolerance and low mortality (Tsuchiya, 1983). Mytilus edulis is thought to be particularly susceptible to high temperatures and heatwaves in the summer, due to the low energy reserves of the organism after spawning (Tremblay et al., 1998, Myrand et al., 2000). Experimental marine heatwave simulations involving repeated +5°C warming events increased valve micro-closure frequency, indicating heightened stress, with some behavioural and molecular effects persisting beyond the recovery period (Grimmelpont et al., 2024). Field-based studies suggest that survival during extreme heat events is strongly influenced by microhabitat and biological context, with shell-associated endolithic microbial communities providing a measurable thermal buffering effect of up to 3.2°C and enhancing survival during the 2022 English Channel heatwave, particularly on the high shore where thermal pressure was greatest (Zardi et al., 2024). Dynamic and constant heatwave experiments further indicate that survival outcomes depend strongly on thermal regime. Vajedsamiei et al. (2024) found that under constant heatwave conditions, survival dropped to zero within seven days at 29°C and within 30 days at 28°C, whereas fluctuating (“dynamic”) heatwave regimes allowed partial survival at similar mean temperatures, highlighting the mitigating role of thermal variability. These findings suggest that while Mytilus edulis can tolerate brief exposure to extreme temperatures, sustained or repeated exposure leads to rapid mortality. Furthermore, evidence from both laboratory simulations and real-world heatwave events indicates that repeated exposure to elevated temperatures can progressively erode thermal tolerance, even when individual exposure events are sub-lethal. Repeated daily heat stress experiments reproducing body temperature profiles recorded during the 2018 English Channel heatwave demonstrated that thermal tolerance consistently declined with successive exposures, leading to increased mortality under otherwise moderate climatic conditions (Seuront et al., 2019). Elevated temperature can exacerbate the effects of other environmental pressures even where warming alone causes limited mortality. In a field-based experiment on the south coast of the UK, Greatorex & Knights (2023) recorded 6% mortality over eight weeks at both control (15°C) and elevated (20°C) temperatures. However, mortality increased to 23% when elevated temperature was combined with simulated ocean acidification, while no mortality occurred under acidification alone. Experimental work under controlled laboratory conditions supports this interaction. Li et al. (2015) exposed adult mussels to temperatures of 19, 22 and 25°C for two months and found that elevated temperature intensified the effects of ocean acidification, resulting in reduced calcification, lower shell calcium content, altered Ca/Mg ratios and downregulation of biomineralisation-related genes. Nutrient enrichment and thermal stress together have produced variable mortality responses depending on exposure timing (Carrier-Belleau et al., 2024). Sensitivity AssessmentUnder the middle emission scenario, if heatwaves occurred every three years, with a maximum intensity of 2°C for 80 days by the end of this century, this could lead to summer sea temperatures reaching up to 24°C in southern England and 19°C in Scotland. Under the middle emission scenario, Alaria esculenta is likely to be lost from the southern parts of the UK (see Global warming pressure). Any remaining populations of Alaria esculenta are likely to suffer severe mortality as a result of a heatwave of this magnitude. Mytilus edulis is thought to have an upper thermal limit of 25 to 28°C in water, although growth decreases at temperatures over 20°C. In addition, intertidal examples of this biotope may be exposed to air temperatures exceeding 30°C in this global warming scenario. Therefore, resistance has been assessed as ‘None’. As a further heatwave is likely to affect this habitat before full recovery, resilience has been assessed as ‘Low’. Therefore, this biotope is assessed as having ‘High’ sensitivity to marine heatwaves under the middle emission scenario. Under the high emission scenario, if heatwaves occur every two years by the end of this century, reaching a maximum intensity of 3.5°C for 120 days, this could lead to the heatwave lasting the entire summer with temperatures reaching up to 26.5°C in southern England and 21.5°C in Scotland. Intertidal examples of this biotope may experience air temperatures exceeding 30°C across much of the UK. Under the high emission scenario, Alaria esculenta is likely to be almost wiped out in the UK. Therefore, resistance has been assessed as ‘None’. As widespread mortality may lead to a lack of viable sporophytes for recruitment, resilience has been assessed as ‘Very low.’ Therefore, this biotope is assessed as having ‘High’ sensitivity to marine heatwaves under the high emission scenario. | NoneHelp | LowHelp | HighHelp |
Ocean acidification (high) [Show more]Ocean acidification (high)High emission scenario benchmark: a further decrease in pH of 0.35 (annual mean) and corresponding 120% increase in H+ ions, seasonal aragonite saturation of 20% of UK coastal waters and North Sea bottom waters, and the aragonite saturation horizon in the NE Atlantic, off the continental shelf, occurring at a depth of 400 m by the end of this century 2081-2100 (Ocean acidification pressure definitions). EvidenceIncreasing levels of CO2 in the atmosphere have led to the average pH of sea surface waters dropping from 8.25 in the 1700s to 8.14 in the 1990s (Jacobson, 2005), with it expected to drop up to a further 0.35 units by the end of this century, dependent on the emission scenario. Marine autotrophs will generally benefit from ocean acidification, through an increase in the availability of aqueous CO2 for photosynthesis (Koch et al., 2013). Most species of kelp appear to be under-saturated in respect to carbon dioxide, although they can generally utilise HCO3 and have external carbonic anhydrase for extracellular dehydration of HCO3 to CO2 (Koch et al., 2013). Under experimental conditions, Iñiguez et al. (2016a) found that although photosynthesis remained stable in Alaria esculenta in response to increasing CO2, and the growth rate increased. Similarly, Gordillo et al. (2015) found heightened growth rates in Alaria esculenta when exposed to increased CO2, although this increase was not significant and less pronounced than in Saccharina lattisima. Research on other kelp species has revealed a positive or neutral effect of ocean acidification (Roleda et al., 2012, Fernández et al., 2015, Nunes et al., 2015, Iñiguez et al., 2016a, b), except for one study, which found that ocean acidification negatively impacted photosynthesis and growth in the southern hemisphere species, Ecklonia radiata (Britton et al., 2016). In general, it is thought that calcifying invertebrates will be more sensitive to ocean acidification than non-calcifying invertebrates, which appear to have a more mixed response (Hofmann et al., 2010), although bivalves generally appear to be tolerant to a decrease in pH (Kroeker et al., 2011, Garrard et al., 2014). Mytilus edulis is a calcified organism but it is unlikely this species will be significantly negatively impacted by ocean acidification, because acidification does not appear to lead to mortality, even at levels which far exceed levels of ocean acidification expected for the end of this century (e.g. Berge et al., 2006, Melzner et al., 2011). For example, levels of growth in Mytilus edulis were maintained at pH 7.6 -7.7, and growth did decrease under pH levels < 7.4 (Berge et al., 2006, Melzner et al., 2011). The calcified shell of Mytilus edulis consists of an outer calcite layer and an inner aragonite layer (Fitzer et al., 2015). When cultured at levels of acidification expected for the end of this century under both the middle (550 ppm) and high (1000 ppm) emission scenario, results showed that Mytilus edulis shells became more brittle (Fitzer et al., 2015). There was no impact of ocean acidification on the production or strength of the byssal threads (Dickey et al., 2018). Beesley et al. (2008) found that the health of Mytilus edulis decreased as a result of 60 days exposure to increased CO2, which they suggested was due to the elevated concentration of calcium ions in the haemolymph. Sun et al. (2017) found that ocean acidification damaged the ultrastructure of haemocytes and led to a reduction in phagocytosis. Corallina officinalis is a highly calcified, erect, red algae. Results of experimental CO2 enrichment suggest that this species could be significantly negatively affected by future ocean acidification. Hofmann et al. (2012) found that growth and photosynthesis decreased as a result of a 0.3 unit decrease in pH. Further investigation showed that skeletal CaCO3 decreased with increasing CO2 at levels expected for both the middle emission and high emission scenarios, although this decrease was small (< 2%) (Hofmann et al., 2013). Yildiz et al. (2013) showed that although CaCO3 decreased in Corallina officinalis as a result of ocean acidification, photosynthesis increased. When ocean acidification was combined with an increase in UV radiation, which led to an increase in growth rate. They summarised that a decrease in CaCO3 content may not be negative but may lead to this species absorbing and using light differently. Brodie et al. (2014) report Corallina species to be more resilient to ocean acidification than other calcified algae species, although competition from flesh algal species that benefit from high CO2 may indirectly cause the loss of calcified species from biotopes. Similarly, observations have indicated Corallinales to be adversely affected at locations where CO2 gradients occur naturally, with evidence of Corallinales being outcompeted by heterokont algae at Mediterranean CO2 seeps (Martin & Hall-Spencer, 2017). Sensitivity assessment. Kelp forests occur in a naturally variable pH habitat, with diel fluctuations of 0.3 - 0.45 pH units (Krause-Jensen et al., 2015, Britton et al., 2016), and boundary layer pH fluctuation of up to 0.8 units (Krause-Jensen et al., 2015). Alaria esculenta is not expected to suffer negative impacts from future acidification, and whilst calcium carbonate content of Corallina officinalis may reduce as a result of acidification, this species is expected to survive future CO2 enrichment of the oceans. In addition, Mytilus edulis is unlikely to be significantly negatively impacted by ocean acidification. Therefore, under both the middle and high emission scenario resistance is assessed as ‘High', and resilience as ‘High’, leading to a sensitivity of ‘Not sensitive’. | MediumHelp | HighHelp | LowHelp |
Ocean acidification (middle) [Show more]Ocean acidification (middle)Middle emission scenario benchmark: a further decrease in pH of 0.15 (annual mean) and a corresponding 35% increase in H+ ions with no coastal aragonite undersaturation and the aragonite saturation horizon in the NE Atlantic, off the continental shelf, at a depth of 800 m by the end of this century, 2081-2100. EvidenceIncreasing levels of CO2 in the atmosphere have led to the average pH of sea surface waters dropping from 8.25 in the 1700s to 8.14 in the 1990s (Jacobson, 2005), with it expected to drop up to a further 0.35 units by the end of this century, dependent on the emission scenario. Marine autotrophs will generally benefit from ocean acidification, through an increase in the availability of aqueous CO2 for photosynthesis (Koch et al., 2013). Most species of kelp appear to be under-saturated in respect to carbon dioxide, although they can generally utilise HCO3 and have external carbonic anhydrase for extracellular dehydration of HCO3 to CO2 (Koch et al., 2013). Under experimental conditions, Iñiguez et al. (2016a) found that although photosynthesis remained stable in Alaria esculenta in response to increasing CO2, and the growth rate increased. Similarly, Gordillo et al. (2015) found heightened growth rates in Alaria esculenta when exposed to increased CO2, although this increase was not significant and less pronounced than in Saccharina lattisima. Research on other kelp species has revealed a positive or neutral effect of ocean acidification (Roleda et al., 2012, Fernández et al., 2015, Nunes et al., 2015, Iñiguez et al., 2016a, b), except for one study, which found that ocean acidification negatively impacted photosynthesis and growth in the southern hemisphere species, Ecklonia radiata (Britton et al., 2016). In general, it is thought that calcifying invertebrates will be more sensitive to ocean acidification than non-calcifying invertebrates, which appear to have a more mixed response (Hofmann et al., 2010), although bivalves generally appear to be tolerant to a decrease in pH (Kroeker et al., 2011, Garrard et al., 2014). Mytilus edulis is a calcified organism but it is unlikely this species will be significantly negatively impacted by ocean acidification, because acidification does not appear to lead to mortality, even at levels which far exceed levels of ocean acidification expected for the end of this century (e.g. Berge et al., 2006, Melzner et al., 2011). For example, levels of growth in Mytilus edulis were maintained at pH 7.6 -7.7, and growth did decrease under pH levels < 7.4 (Berge et al., 2006, Melzner et al., 2011). The calcified shell of Mytilus edulis consists of an outer calcite layer and an inner aragonite layer (Fitzer et al., 2015). When cultured at levels of acidification expected for the end of this century under both the middle (550 ppm) and high (1000 ppm) emission scenario, results showed that Mytilus edulis shells became more brittle (Fitzer et al., 2015). There was no impact of ocean acidification on the production or strength of the byssal threads (Dickey et al., 2018). Beesley et al. (2008) found that the health of Mytilus edulis decreased as a result of 60 days exposure to increased CO2, which they suggested was due to the elevated concentration of calcium ions in the haemolymph. Sun et al. (2017) found that ocean acidification damaged the ultrastructure of haemocytes and led to a reduction in phagocytosis. Corallina officinalis is a highly calcified, erect, red algae. Results of experimental CO2 enrichment suggest that this species could be significantly negatively affected by future ocean acidification. Hofmann et al. (2012) found that growth and photosynthesis decreased as a result of a 0.3 unit decrease in pH. Further investigation showed that skeletal CaCO3 decreased with increasing CO2 at levels expected for both the middle emission and high emission scenarios, although this decrease was small (< 2%) (Hofmann et al., 2013). Yildiz et al. (2013) showed that although CaCO3 decreased in Corallina officinalis as a result of ocean acidification, photosynthesis increased. When ocean acidification was combined with an increase in UV radiation, which led to an increase in growth rate. They summarised that a decrease in CaCO3 content may not be negative but may lead to this species absorbing and using light differently. Brodie et al. (2014) report Corallina species to be more resilient to ocean acidification than other calcified algae species, although competition from flesh algal species that benefit from high CO2 may indirectly cause the loss of calcified species from biotopes. Similarly, observations have indicated Corallinales to be adversely affected at locations where CO2 gradients occur naturally, with evidence of Corallinales being outcompeted by heterokont algae at Mediterranean CO2 seeps (Martin & Hall-Spencer, 2017). Sensitivity assessment. Kelp forests occur in a naturally variable pH habitat, with diel fluctuations of 0.3 - 0.45 pH units (Krause-Jensen et al., 2015, Britton et al., 2016), and boundary layer pH fluctuation of up to 0.8 units (Krause-Jensen et al., 2015). Alaria esculenta is not expected to suffer negative impacts from future acidification, and whilst calcium carbonate content of Corallina officinalis may reduce as a result of acidification, this species is expected to survive future CO2 enrichment of the oceans. In addition, Mytilus edulis is unlikely to be significantly negatively impacted by ocean acidification. Therefore, under both the middle and high emission scenario resistance is assessed as ‘High', and resilience as ‘High’, leading to a sensitivity of ‘Not sensitive’. | HighHelp | HighHelp | Not sensitiveHelp |
Sea level rise (extreme) [Show more]Sea level rise (extreme)Extreme scenario benchmark: a 107 cm rise in average UK sea-level by the end of this century (2018-2100) (Sea-level rise pressure definitions). EvidenceSea-level rise is occurring through a combination of thermal expansion and ice melt. Sea levels have risen 1-3 mm/yr in the last century (Cazenave & Nerem, 2004, Church et al., 2004, Church & White, 2006). Sea-level rise is expected to lead to substantial loss of intertidal habitats. Rocky shores backed by cliffs constitute about 80% of oceanic coastlines globally and in Britain, 42% of the coastline is hard rock, with many areas having cliffs behind the shore (Jackson & McIlvenny, 2011). Jackson & McIlvenny (2011) predicted that under a 30 cm sea-level rise, between 10 - 27% of the extent of intertidal rocky shores in Scotland would be lost, whilst under a 190 cm sea-level rise, between 26 - 50% would be lost. Using a modelling-based approach, Kaplanis et al. (2019) found that in San Diego County loss of intertidal habitat would be most extreme within the first metre of sea-level rise, with 29.9% of intertidal rocky shore lost as a result of a 20 cm sea-level rise, and 77.7% as a result of a 100 cm sea-level rise. Sensitivity assessment. This biotope IR.HIR.KFaR.Ala.Myt is found on very exposed fringe bedrock on the lower shore and shallow subtidal, and therefore an increase in sea level height of 50, 70 and 107 cm could have severe repercussions for the extent of this biotope. Beds may be able to expand their range and migrate upwards to compensate for sea-level rise, if not constrained by lack of suitable habitat (IPCC, 2019). In this assessment we have assessed on a worst-case-scenario basis, assuming that landward migration is not possible, which is likely to lead to the depth distribution of Alaria esculenta and Mytilus edulis shrinking significantly in response to a 50, 70 or 107 cm sea-level rise, without the possibility of recovery. Alaria esculenta is generally limited to a depth of 1-2 m, as below this depth it is usually outcompeted by Laminaria hyperborea. As depth increases due to sea-level rise, Laminaria hyperborea is likely to extend its distribution shorewards. Under the middle emission, high emission and extreme scenarios (50, 70 and 107 cm sea-level rise), it is expected that between 25 - 75% of this biotope is likely to be lost. Therefore, for all three scenarios, resistance has been assessed as ‘Low’, and resilience as ‘Very low’, and sensitivity is assessed as ‘High’. | LowHelp | Very LowHelp | HighHelp |
Sea level rise (high) [Show more]Sea level rise (high)High emission scenario benchmark: a 70 cm rise in average UK sea-level by the end of this century (2018-2100). EvidenceSea-level rise is occurring through a combination of thermal expansion and ice melt. Sea levels have risen 1-3 mm/yr in the last century (Cazenave & Nerem, 2004, Church et al., 2004, Church & White, 2006). Sea-level rise is expected to lead to substantial loss of intertidal habitats. Rocky shores backed by cliffs constitute about 80% of oceanic coastlines globally and in Britain, 42% of the coastline is hard rock, with many areas having cliffs behind the shore (Jackson & McIlvenny, 2011). Jackson & McIlvenny (2011) predicted that under a 30 cm sea-level rise, between 10 - 27% of the extent of intertidal rocky shores in Scotland would be lost, whilst under a 190 cm sea-level rise, between 26 - 50% would be lost. Using a modelling-based approach, Kaplanis et al. (2019) found that in San Diego County loss of intertidal habitat would be most extreme within the first metre of sea-level rise, with 29.9% of intertidal rocky shore lost as a result of a 20 cm sea-level rise, and 77.7% as a result of a 100 cm sea-level rise. Sensitivity assessment. This biotope IR.HIR.KFaR.Ala.Myt is found on very exposed fringe bedrock on the lower shore and shallow subtidal, and therefore an increase in sea level height of 50, 70 and 107 cm could have severe repercussions for the extent of this biotope. Beds may be able to expand their range and migrate upwards to compensate for sea-level rise, if not constrained by lack of suitable habitat (IPCC, 2019). In this assessment we have assessed on a worst-case-scenario basis, assuming that landward migration is not possible, which is likely to lead to the depth distribution of Alaria esculenta and Mytilus edulis shrinking significantly in response to a 50, 70 or 107 cm sea-level rise, without the possibility of recovery. Alaria esculenta is generally limited to a depth of 1-2 m, as below this depth it is usually outcompeted by Laminaria hyperborea. As depth increases due to sea-level rise, Laminaria hyperborea is likely to extend its distribution shorewards. Under the middle emission, high emission and extreme scenarios (50, 70 and 107 cm sea-level rise), it is expected that between 25 - 75% of this biotope is likely to be lost. Therefore, for all three scenarios, resistance has been assessed as ‘Low’, and resilience as ‘Very low’, and sensitivity is assessed as ‘High’. | LowHelp | Very LowHelp | HighHelp |
Sea level rise (middle) [Show more]Sea level rise (middle)Middle emission scenario benchmark: a 50 cm rise in average UK sea-level by the end of this century (2081-2100). EvidenceSea-level rise is occurring through a combination of thermal expansion and ice melt. Sea levels have risen 1-3 mm/yr in the last century (Cazenave & Nerem, 2004, Church et al., 2004, Church & White, 2006). Sea-level rise is expected to lead to substantial loss of intertidal habitats. Rocky shores backed by cliffs constitute about 80% of oceanic coastlines globally and in Britain, 42% of the coastline is hard rock, with many areas having cliffs behind the shore (Jackson & McIlvenny, 2011). Jackson & McIlvenny (2011) predicted that under a 30 cm sea-level rise, between 10 - 27% of the extent of intertidal rocky shores in Scotland would be lost, whilst under a 190 cm sea-level rise, between 26 - 50% would be lost. Using a modelling-based approach, Kaplanis et al. (2019) found that in San Diego County loss of intertidal habitat would be most extreme within the first metre of sea-level rise, with 29.9% of intertidal rocky shore lost as a result of a 20 cm sea-level rise, and 77.7% as a result of a 100 cm sea-level rise. Sensitivity assessment. This biotope IR.HIR.KFaR.Ala.Myt is found on very exposed fringe bedrock on the lower shore and shallow subtidal, and therefore an increase in sea level height of 50, 70 and 107 cm could have severe repercussions for the extent of this biotope. Beds may be able to expand their range and migrate upwards to compensate for sea-level rise, if not constrained by lack of suitable habitat (IPCC, 2019). In this assessment we have assessed on a worst-case-scenario basis, assuming that landward migration is not possible, which is likely to lead to the depth distribution of Alaria esculenta and Mytilus edulis shrinking significantly in response to a 50, 70 or 107 cm sea-level rise, without the possibility of recovery. Alaria esculenta is generally limited to a depth of 1-2 m, as below this depth it is usually outcompeted by Laminaria hyperborea. As depth increases due to sea-level rise, Laminaria hyperborea is likely to extend its distribution shorewards. Under the middle emission, high emission and extreme scenarios (50, 70 and 107 cm sea-level rise), it is expected that between 25 - 75% of this biotope is likely to be lost. Therefore, for all three scenarios, resistance has been assessed as ‘Low’, and resilience as ‘Very low’, and sensitivity is assessed as ‘High’. | LowHelp | Very LowHelp | HighHelp |
Hydrological Pressures
Use [show more] / [show less] to open/close text displayed
| Resistance | Resilience | Sensitivity | |
Temperature increase (local) [Show more]Temperature increase (local)Benchmark. A 5°C increase in temperature for one month, or 2°C for one year (Temperature change pressure definition). EvidenceAlaria esculentaAlaria esculenta is a northern/boreal species that has been recorded from Brittany, France to Northern Norway (Birkett et al., 1998). Its approximate mid-range is within southern Norway (60° to 65° North) (Birkett et al., 1998), so these biotopes are in Alaria esculenta’s southern range. Throughout the UK, northern to southern Sea Surface Temperature (SST) ranges from 8 to 16°C in summer and 6 to 13°C in winter (Beszczynska-Möller & Dye, 2013). Sea temperature regulates Alaria esculenta metabolism and reproduction (Fredersdorf et al., 2009). Their southern limit has been defined at the 20°C isotherm (Munda & Lüning, 1977; Fredersdorf et al., 2009), but it is common north of the 16°C isotherm (Munda & Lüning, 1977). As a result of this upper temperature threshold, Alaria esculenta is largely absent from the southern North Sea and English Channel where summer temperatures can exceed 16°C. According to OBIS (2026), Alaria esculenta occurs in waters ranging from -5 to 15°C, with most records in the 10 to 15°C range. Much of the research on Alaria esculenta responses to increased temperatures was based on Arctic populations where temperatures are far cooler than those experienced by this biotope in the UK. The temperature treatments used in these studies are reflective of the current and predicted future temperatures (under global warming scenarios) of the study region. As this biotope occurs throughout the UK, caution is needed when basing assessments on evidence from colder Arctic regions, where characteristic species may have different physiological responses and thermal tolerances to populations occurring around the UK where Alaria esculenta are living closer to the upper limit of their thermal tolerance. Munda & Lüning (1977) observed temperatures of 16 to 17°C sustained over two weeks in Helgoland, Germany, were lethal to resident Alaria esculenta. Experimental observations showed that acute exposure to ≥21°C is lethal to Alaria esculenta causing bleaching and disintegration (Sundene, 1962; Fredersdorf et al., 2009). Experimental observations conducted by Fredersdorf et al. (2009) found the optimal temperature for sporophyte photosynthesis was within the range of 13 to 17°C. However, the optimal temperatures for Alaria esculenta germination is 2 to 12°C (Fredersdorf et al., 2009). Park et al. (2017) reported higher growth rates at 10 to 15°C than at 5°C in Alaria esculenta gametophytes sourced from Arctic waters. In addition, they reported gametophyte mortality at 20°C. Zacher et al. (2019) found that in Arctic populations, gametogenesis and sporophyte growth was reduced at 15°C compared to 9 to 10°C. They also found that co-cultivation with Laminaria digitata enhanced growth. Sporophytes show rapid recovery of growth and photosynthetic activity after the return of light following polar night, where kelps spend months in total darkness, but this can be diminished by elevated temperatures by as little as 4°C (Gordillo et al., 2022; Cobos et al., 2026). Martins et al. (2022) investigated whether photoperiod conditions during gametophyte development influence the response of Alaria esculenta sporophytes to temperature. Sporophyte growth was highest at 6°C and declined steadily with increasing temperature, with minimal growth at 21 to 22°C. The photoperiod experienced during the gametophyte stage influenced subsequent sporophyte performance, particularly at 6°C, where growth increased under shorter day lengths. However, elevated temperatures generally reduced growth across all photoperiod treatments. These findings demonstrate that warming strongly limits Alaria esculenta growth and can interact with environmental conditions experienced during earlier life stages to affect later performance. Park et al. (2017) examined the thermal tolerance of Arctic Alaria esculenta gametophytes from Spitsbergen by culturing them at 5, 10, 15, and 20°C. Gametophytes survived and grew best at 10 to 15°C, with greater germling size and cell numbers than at the control temperature (5°C), while all individuals died at 20°C. Photosynthetic performance remained stable across 5 to 15°C but collapsed at 20°C. These results suggest that Arctic Alaria esculenta can maintain growth and photosynthetic function at temperatures 5 to 10°C above those currently experienced in its natural habitat, although temperatures of 20°C exceed its thermal tolerance. A 5°C increase in temperature was enough to result in an approximate 50% loss of Alaria esculenta biomass over simulated Arctic winter conditions where kelps spend months in total darkness (Gordillo et al., 2022). Kelps lost 21% more biomass during the prolonged darkness at 8°C than those kept at 3°C. Towards the end of the dark period, Alaria esculenta produced new blade tissue in the 3°C treatment, which continued to grow for two months after light returned. However, in the 8°C treatment, only the holdfast and midrib were left, and growth was unable to resume. In a similar experiment, Cobos et al. (2026) also found that elevated temperatures negatively affected Alaria esculenta during the polar night. In the 2-week light period following the dark period, Alaria esculenta growth resumed in both 1 and 5°C treatments, but more so in the cold treatment. These studies show that warming can have a strong negative effect on Alaria esculenta even in colder and darker areas, and this effect can persist even after light levels return to normal. Some studies have shown that the effects of temperature on Alaria esculenta can vary depending on other pressures. Silva et al. (2022) showed that warming partially offset the negative effects of high light on gametophyte density under low-nutrient conditions. However, under high-nutrient conditions, warming intensified the negative effects of high light. Moreover, Gordillo et al. (2016) showed that higher CO₂ levels partially offset some negative physiological effects of warming. Furthermore, Zacher et al. (2016) showed that warming by itself increased Alaria esculenta germination and sporophyte growth and that warming can partially offset the negative effects of grazing and sedimentation. Yesson et al. (2015) reported no significant change in Alaria esculenta abundance in the UK from 1974 to 2010, and no relationship between abundance and summer and winter sea surface temperatures. Despite this, they noted the contrast between their findings and those of previous research that reported declines in Alaria esculenta around the UK and Ireland, and suggested that if temperatures increase in the future, then abundances could change. Lebrun et al. (2025) studied marine heatwave (MHW) effects on three kelp species including Alaria esculenta. In their mesocosm experiment, water flow was supplied directly from the ocean, ensuring that the control treatment reflected natural conditions. Control temperatures ranged from approx. 7.5 to 10°C. Additional treatments included a constant high-temperature treatment (HT; +1.8°C above control), a single 13-day MHW treatment (1MH; +2.8°C above control), and a treatment simulating two consecutive 5-day MHWs (2MH; +3.9°C above control). No mortality was reported, but physiological responses varied. Net photosynthetic rates declined significantly between the beginning and end of the experiment in all treatments, with a significant decline occurring by the midpoint of the experiment in the HT treatment. Photosynthetic efficiency (FV/FM) remained above 0.7 throughout, indicating good physiological condition. Chlorophyll-a content differed significantly between the beginning and end of the experiment only in the 2MH treatment, while significant differences in C:N ratios were detected only between the 1MH and 2MH treatments at the end of the experiment. Growth rates did not differ among treatments. Overall, these findings suggest that Alaria esculenta remained physiologically healthy and maintained growth under the simulated MHW conditions, although some changes in photosynthetic performance, pigmentation, and C:N ratios occurred. Mytilus edulisLocal Mytilus edulis populations may be acclimated to prevailing temperature regimes and could therefore exhibit different tolerances from populations exposed to different salinity conditions. Consequently, caution should be exercised when inferring tolerances across regions. Mytilus edulis is a eurytopic species that occurs across a broad temperature range, from mild subtropical regions to areas that frequently experience freezing conditions and ice scour (Seed & Suchanek, 1992). In recent years, Mytilus edulis has expanded its range poleward and reappeared in Svalbard due to increasing sea temperatures (Berge et al., 2005), while its equatorial range limits have contracted because water temperatures now exceed its lethal threshold (Jones et al., 2010). In British waters, 29°C has been reported as the upper sustained thermal tolerance limit for Mytilus edulis (Read & Cumming, 1967; Almada-Villela et al., 1982), although European mussels are thought to rarely experience temperatures above 25°C (Seed & Suchanek, 1992). According to OBIS (2026), Mytilus edulis occurs in temperatures ranging from 5 to 20°C, with most records between 10 and 15°C. Experimental and field evidence indicates that adult Mytilus edulis possess considerable thermal plasticity and acclimation capacity. Long-term observations in the White Sea detected no significant change in heart rate despite an approx. 4°C increase in summer seawater temperature (Bakhmet et al., 2019). Controlled laboratory experiments further showed that Mytilus edulis has a higher thermal tolerance and lower, more stable heart rate responses than the closely related Mytilus trossulus. Mortality in Mytilus edulis was negligible during progressive warming trials, despite temperatures increasing at 2°C/hour from 1.8 to 28.8°C (Bakhmet et al., 2022). Studies from multiple regions indicate that adult mussels can tolerate short-term warming to at least 27 to 30°C with limited cellular stress responses. Greenland populations exhibited minimal transcriptional disruption even at 32°C, suggesting a broad capacity for acclimation across contrasting thermal histories (mussels were collected from environments of 27, 19, and 3°C; Clark et al., 2021). Similarly, mussels from the remote sub-Antarctic Kerguelen Archipelago exposed to rapid warming from 7.5 to 20°C displayed a typical but controlled stress response, consistent with conserved protein homeostasis mechanisms rather than acute physiological failure (Bultelle et al., 2021). Archival shell records from the Belgian coast further suggest long-term acclimation or adaptation to increasing thermal variability, with no clear reduction in shell growth despite the greater energetic demands associated with warming (Telesca et al., 2021). Tsuchiya (1983) documented mass mortality of Mytilus edulis in Mutsu Bay, northern Japan when air temperatures of 34°C caused mussel tissue temperatures to exceed 40°C. Within one hour, 50% of Mytilus edulis individuals occupying the upper 75% of the shore had died. It was unclear whether mortality resulted from high temperatures, desiccation, or a combination of both factors. Lethal temperature thresholds appear to vary among regions (Tsuchiya, 1983), although thermal tolerance is influenced by the temperature range to which individuals are acclimated (Kittner & Riisgaard, 2005). Following acclimation to 18°C, Mytilus edulis exhibited maximum filtration rates between 8.3 and 20°C, whereas at 6°C the mussels closed their valves (Kittner & Riisgaard, 2005). However, after five days of acclimation at 11°C, high filtration rates were maintained down to 4°C, demonstrating the species' capacity to adjust its thermal tolerance through acclimation. Barrett et al. (2022) examined gene expression responses under combined warming (30 and 33°C) and reduced salinity (15 vs 23 PSU) and found that similar physiological pathways were activated across all treatments, with progressively stronger upregulation as stressors accumulated. This pattern suggests that while Mytilus edulis is highly resilient to heat stress and can acclimate efficiently to reduced salinity, combined stressors increasingly push individuals towards physiological limits, particularly under more extreme hyposaline conditions (5 PSU), where strong expression of stress and osmoregulatory marker genes was observed. Long-term evidence indicates that moderate warming can enhance growth under some conditions, but sustained temperature increases are associated with declines in condition and biomass at broader spatial and temporal scales. Growth rates of Mytilus edulis in the Wadden Sea were positively correlated with temperature over a 40-year period within a relatively narrow thermal range (11.2 to 14.4°C), suggesting that mild warming may be beneficial (Beukema et al., 2017). In contrast, Scottish rocky shore monitoring provides no evidence of temperature-driven declines in Mytilus edulis at recent levels of warming. As part of the MarClim project, the thermal affinity of Mytilus edulis was assessed alongside population trends around Scotland, with analyses from 2020 to 2022 finding no consistent relationship between species thermal affinity, geographic range position, and whether populations increased or declined between survey periods, despite measurable warming of Scottish coastal waters since 2014 to 2015 (Burrows et al., 2020). However, mussel body condition declined linearly with increasing temperature over a five-month experimental period spanning 4.8 to 8.2°C, indicating energetic constraints under sustained warming (Melzner et al., 2020). Regional declines in mussel abundance have been documented in rapidly warming areas such as the Gulf of Maine, where populations have declined by more than 60% over the past 40 years, coinciding with increasing temperates of >0.2°C/year (Sorte et al., 2017; Matoo et al., 2021). This interpretation is consistent with a synthesis by Metcalf (2019) which identified sustained increases in sea surface temperature (>2°C over approx. 20 years) as the primary driver of the widespread decline of blue mussel populations in the Gulf of Maine. In the Northeast Atlantic, population-scale modelling suggests that while individual growth potential may increase slightly under future climate scenarios (RCP 8.5 - the IPCC’s “worst case” scenario), overall biomass is likely to decline due to altered recruitment phenology and spatially heterogeneous responses to warming, including a total halt in recruitment during summer (Thomas & Bacher, 2018; Thomas et al., 2020). Increased temperatures can affect reproduction in Mytilus edulis (Myrand et al., 2000). In shallow lagoons, mortality began in late July at the end of a major spawning event when temperatures peaked at >20°C. These mussels had a low energetic content post-spawning and had stopped shell growth. It is likely that the high temperatures caused mortality due to the reduced condition of the mussels post-spawning (Myrand et al., 2000). Gamete production does not appear to be affected by temperature (Suchanek, 1985). More recent evidence indicates that reproductive responses to temperature are non-linear and context dependent. Oliveira et al. (2021) showed that relative fecundity was strongly influenced by the number of days with seawater temperatures exceeding 14°C during the preceding four months. The highest positive effect occurred at approx. 80 warm days, while relative fecundity declined sharply when the number of warm days exceeded 100. Average sea surface temperature also influenced fecundity, but only when temperatures exceeded 16°C. The authors cautioned that predictive models based on linear temperature-fecundity relationships may overestimate the ability of Mytilus edulis to cope with future warming scenarios. Experimental studies indicate that survival declines rapidly once upper thermal thresholds are exceeded, particularly under sustained exposure. Complete mortality has been observed after 3 to 32 days at 30°C, with faster mortality at higher temperatures and declining condition index prior to death (Kamermans & Saurel, 2022). Laboratory mortality experiments also demonstrate strong interactions between temperature and salinity, with low salinity substantially reducing upper thermal tolerance; exposure to air temperatures of 30 to 36°C resulted in sharply increased mortality under hyposaline conditions compared to full salinity treatments (Nielsen et al., 2021). Dynamic and constant heatwave experiments further indicate that survival outcomes depend strongly on thermal regime. Vajedsamiei et al. (2024) found that under constant heatwave conditions, survival dropped to zero within seven days at 29°C and within 30 days at 28°C, whereas fluctuating (“dynamic”) heatwave regimes allowed partial survival at similar mean temperatures, highlighting the mitigating role of thermal variability. These findings suggest that while Mytilus edulis can tolerate brief exposure to extreme temperatures, sustained or repeated exposure leads to rapid mortality. Furthermore, evidence from both laboratory simulations and real-world heatwave events indicates that repeated exposure to elevated temperatures can progressively erode thermal tolerance, even when individual exposure events are sublethal. Repeated daily heat stress experiments reproducing body temperature profiles recorded during the 2018 English Channel heatwave demonstrated that thermal tolerance consistently declined with successive exposures, leading to increased mortality under otherwise moderate climatic conditions (Seuront et al., 2019). Experimental marine heatwave simulations involving repeated +5°C warming events increased valve micro-closure frequency, indicating heightened stress, with some behavioural and molecular effects persisting beyond the recovery period (Grimmelpont et al., 2024). Field-based studies suggest that survival during extreme heat events is strongly influenced by microhabitat and biological context, with shell-associated endolithic microbial communities providing a measurable thermal buffering effect of up to 3.2°C and enhancing survival during the 2022 English Channel heatwave, particularly on the high shore where thermal pressure was greatest (Zardi et al., 2024). Early life stages appear to be more sensitive to elevated temperatures. Laboratory studies have shown increasing larval abnormalities and developmental arrest with rising temperatures, with complete developmental failure occurring at 24°C (Boukadida et al., 2021). Juvenile mussels exposed to short-term warming up to 24°C exhibited 37% higher mortality than controls, although surviving individuals showed compensatory increases in shell and tissue growth (Guillou et al., 2023). Studies indicate that extreme thermal events early in life can alter cohort genetic composition, favouring heat-tolerant genotypes while reducing overall performance and tissue mass (Nascimento-Schulze et al., 2025). Recruitment experiments simulating future thermal regimes demonstrated that recruitment success may decline by more than 96% under +4°C warming, even where surviving recruits exhibit enhanced thermal recovery capacity (Vajedsamiei, Wahl et al., 2021). Burial experiments demonstrated significantly higher mortality under elevated (+5°C) temperatures, particularly in organically enriched fine sediments, likely due to increased bacterial activity and metabolic demand under hypoxic conditions (Cottrell et al., 2016). Experiments combining warming and ocean acidification have shown substantially lower survival than warming alone (Voet et al., 2022), while the combined effects of nutrient enrichment and thermal stress produced variable mortality responses depending on exposure timing (Carrier-Belleau et al., 2024). Long-term hazard analyses from the Wadden Sea identified increased failure rates of newly formed mussel beds under combined elevated temperature, low salinity, and reduced oxygen conditions, even where hypoxia alone had no detectable effect (Johansson et al., 2024). Greatorex & Knights (2023) recorded 6% mortality over eight weeks at both control (15°C) and elevated (20°C) temperatures. However, mortality increased to 23% when elevated temperature was combined with simulated ocean acidification, whereas acidification alone caused no mortality. Moreover, Li et al. (2015) exposed adult mussels to temperatures of 19, 22, and 25°C for two months and found that elevated temperature intensified the effects of ocean acidification, resulting in reduced calcification, lower shell calcium content, altered Ca/Mg ratios, and downregulation of biomineralization-related genes. Power stations can increase local sea temperatures by up to 15°C (Cole et al., 1999), although these impacts are local. Nevertheless, as mussels are among the most problematic biofouling organisms at power station water intakes, they are clearly capable of persisting under such conditions (Whitehouse et al., 1985; Thompson et al., 2000). Evidence from recent extreme heat events in north-west Europe demonstrates that mussels in UK-relevant biotopes can experience body temperatures substantially higher than ambient seawater temperatures during calm, sunny conditions. Heatwave observations show that intertidal mussel body temperatures frequently exceed 30°C for several consecutive days, with localised mass mortality recorded despite relatively moderate climatic heatwave conditions (Seuront et al., 2019; Talevi et al., 2023). Sensitivity AssessmentThe available evidence suggests that the effects of an increase in temperature would be seasonally variable. A 5°C increase in temperature for one month during the summer may cause significant mortality and reproductive failure in Alaria esculenta, while a 2°C increase in temperature for one year may limit germination. Resistance is therefore ‘None’, while resilience is ‘High’, and sensitivity is ‘Medium’ for KFaR.Ala.Myt. | NoneHelp | HighHelp | MediumHelp |
Temperature decrease (local) [Show more]Temperature decrease (local)Benchmark. A 5°C decrease in temperature for one month, or 2°C for one year (Temperature change pressure definition). EvidenceAlaria esculentaAlaria esculenta is a northern/boreal species that has been recorded from Brittany, France to Northern Norway (Birkett et al., 1998). Sea temperature has been cited as an influential abiotic stressor; responsible for regulating metabolism and reproduction, plus defining the regional distribution of Alaria esculenta (Fredersdorf et al., 2009). At Alaria esculenta’s northern range edge (Svalbard) it is a prominent macroalgae on sub-littoral fringe bedrock. At these latitudes, average summer temperature can reach 5°C, and average annual sea temperature 3°C (1980 to 2014, Beszczynska-Möller & Dye, 2013). Experimental observations conducted by Fredersdorf et al., (2009) found the optimal temperature for sporophyte photosynthesis was within the range of 13 to 17°C, however, the optimal temperatures for Alaria esculenta germination are 2 to12°C (Fredersdorf et al., 2009). According to OBIS (2026), Alaria esculenta occurs in waters ranging from -5 to 15°C, with most records in the 10 to 15°C range. Alaria esculenta has an approximate mid-range within southern Norway (60° to 65° North) (Birkett et al., 1998), and as such UK biotopes have a southerly distribution when considering the geographic distribution of Alaria esculenta. Throughout the UK northern to southern Sea Surface Temperature (SST) ranges from 8 to 16°C in summer and 6 to 13°C in winter (Beszczynska-Möller & Dye, 2013). Mytilus edulisMytilus edulis is a eurytopic species found in a wide temperature range from mild, subtropical regions to areas which frequently experience freezing conditions and are vulnerable to ice scour (Seed & Suchanek 1992). The lower lethal limit of Mytilus edulis depends on the length of time exposed to a low temperature and the frequency of exposure (Bourget, 1983). Williams (1970) observed that Mytilus edulis tolerated a tissue temperature as low as -10°C. In a laboratory experiment, Bourget (1983) showed that the 24-hour median lethal temperature in Mytilus edulis was -16°C for large mussels (>3 cm) and -12.5°C for juveniles (<1.5 cm). However, when exposed to reduced temperatures for only 16 hours, the median lethal temperature of large mussels decreased to -20°C. It was also reported that mussels exposed to sub lethal temperatures cyclically, e.g. -8°C every 12.4 hours for 3 to 4 days, suffered significant damage likely to lead to death (Bourget, 1983), which suggested that while Mytilus edulis could tolerate occasional sharp frost events it was not likely to survive prolonged periods of very low temperatures. During the cold winter of 1962/63, Mytilus edulis was reported to have experienced relatively few effects with only 30% mortality being recorded from the south-east coast of England (Whitstable area) and only about 2% mortality reported from Rhosilli in South Wales (Crisp, 1964). Crisp (1964) also noted that the mortality was mainly from predation on the individuals that were weakened by the low temperatures rather than the temperature itself. It is thought that the use of nucleating agents in the haemolymph and the maintenance of a high osmotic concentration in the mantle fluid during periods of winter isolation allows Mytilus edulis to tolerate such low temperatures (Aunaas et al., 1988). According to OBIS (2026), Mytilus edulis occurs in temperatures ranging from 5 to 20°C, with most records in the 10 to 15°C range. After acclimation of individuals of Mytilus edulis to 18°C, Kittner & Riisgaard (2005) observed that the filtrations rates were at their maximum between 8.3 and 20°C and below this at 6°C the mussels closed their valves. However, after being acclimated at 11°C for five days, the mussels maintained the high filtration rates down to 4°C. Hence, given time, mussels can acclimatise and shifting their temperature tolerance. Filtration in Mytilus edulis was observed to continue down to -1°C, with high absorption efficiencies (53 to 81%) (Loo, 1992). Field and laboratory studies demonstrate that Mytilus edulis maintains active metabolism and physiological function at very low temperatures, supporting its ability to withstand temperature decreases at the benchmark. In natural winter conditions (-1.8 to -0.6°C), Mytilus edulis maintained heart rates of 3 to 8 bpm under thick ice, with metabolic activity remaining stable throughout the winter-spring period, indicating that individuals do not enter a dormant state even at sub-zero temperatures (Bakhmet, 2017; Bakhmet et al., 2019). Laboratory studies across latitudinal gradients further demonstrate strong physiological plasticity, with Arctic and sub-Arctic populations maintaining active metabolic rates at -1°C and surviving air temperatures down to -13°C, exceeding the tolerance of temperate populations (Thyrring et al., 2015; Thyrring et al., 2019). Even in newly established high-Arctic populations, shell growth and behavioural rhythms continued annually despite extremely low temperatures (Tran et al., 2020), while temperate populations maintain effective feeding rates as water temperature declines from approx. 18 to 5°C (Rosa et al., 2024). Collectively, these studies demonstrate strong physiological plasticity and cold tolerance, indicating that UK Mytilus edulis populations are likely to withstand the magnitude of acute or chronic local temperature decreases considered at the benchmark. Early life stages are similarly resilient, with mussel settlement documented in Antarctic waters where winter minima reached -1.9°C, following accidental introduction via shipping traffic from much warmer regions with annual temperature ranges analogous to the UK (Cárdenas et al., 2020). While low spring temperatures can sometimes reduce recruitment locally, long-term monitoring in the south-west Baltic indicates that population-level recovery depends on subsequent conditions and larval connectivity rather than cold exposure alone (Franz et al., 2019). Cold temperature effects may instead be expressed through changes in reproductive timing rather than direct mortality: in Newfoundland, mussels from deeper, colder sites (mean annual temperature 4.36 ± 5.1°C) maintained high reproductive indices for longer into the summer than mussels from shallower, slightly warmer sites (5.81 ± 6.3°C), indicating that lower and more stable thermal regimes do not inhibit, and may prolong, reproductive readiness (Murray et al., 2019). Shell growth is not expected to be majorly influenced by low temperatures. Bayne (1976) demonstrated that between 10 and 20°C water temperature had little effect on the scope for growth, similar to the findings of Page & Hubbard (1987), who found that a temperature range of 10 to 18°C did not influence growth rate. In addition, Loo (1992) recorded growth rates of up to 0.7% at temperatures as low as -1°C, with an excess of seston, a rate higher than the same author recorded in mussel culture in Sweden (Loo & Rosenberg, 1983). They concluded that food availability was more of a limiting factor to growth than temperature (Loo, 1992). Tsuchiya (1983) documented mass mortality of Mytilus edulis in Mutsu Bay, northern Japan when air temperatures of 34°C caused mussel tissue temperatures to exceed 40°C. Within one hour, 50% of Mytilus edulis individuals occupying the upper 75% of the shore had died. It was unclear whether mortality resulted from high temperatures, desiccation, or a combination of both factors. Lethal temperature thresholds appear to vary among regions (Tsuchiya, 1983), although thermal tolerance is influenced by the temperature range to which individuals are acclimated (Kittner & Riisgaard, 2005). Following acclimation to 18°C, Mytilus edulis exhibited maximum filtration rates between 8.3 and 20°C, whereas at 6°C the mussels closed their valves (Kittner & Riisgaard, 2005). However, after five days of acclimation at 11°C, high filtration rates were maintained down to 4°C, demonstrating the species' capacity to adjust its thermal tolerance through acclimation. Filtration has also been observed at temperatures as low as -1°C, with high absorption efficiencies of 53 to 81% (Loo, 1992). Sensitivity AssessmentA 5°C decrease in temperature for one month or a 2°C decrease for one year is unlikely to significantly affect populations of the characterising species. Resistance is therefore ‘High’, resilience is ‘High’, and sensitivity is assessed as ‘Not Sensitive’. | HighHelp | HighHelp | Not sensitiveHelp |
Salinity increase (local) [Show more]Salinity increase (local)Benchmark. An increase in one MNCR salinity category above the usual range of the biotope or habitat (Salinity regime change pressure definition). EvidenceThe biotope has only been recorded from conditions of full salinity (Connor et al., 2004; JNCC, 2015, 2022). Intertidal examples of these biotopes will naturally experience fluctuations in salinity where evaporation increases salinity and inputs of rainwater reduces salinity. Species found in the intertidal likely have some form of behavioural or physiological adaptations to changes in salinity. Lüning (1990) suggest that kelps are stenohaline, their general tolerance to salinity as a phenotypic group covering 16 to 50 PSU over a 24-hour period. Optimal growth probably occurs between 30 to 35 PSU (MNCR category: Full Salinity) and growth rates are likely to be affected by periodic salinity stress. Alaria esculentaAccording to OBIS (2026), Alaria esculenta occurs in waters ranging from 15 to 40 PSU, with most records in the 30 to 35 PSU range. Karsten (2007) tested the photosynthetic ability of Alaria esculenta under acute 2 and 5-day exposures to salinity treatments ranging from 5 to 60 PSU. A control experiment was also carried at 34 PSU. Between 10 to 50 PSU, Alaria esculenta showed high photosynthetic ability at 83 to 94% of the control. Hypersaline treatments with 55 to 60 PSU led to a 30% reduction in photosynthetic ability, approx. 70% of the control level. At 5 PSU, Alaria esculenta showed a low photosynthetic ability at 15.8% of the control. After 5 days at 5 PSU, all Alaria esculenta specimens were bleached and none survived. Karsten (2007) suggested that Alaria esculenta photosynthetic ability is highly affected by acute exposure to hyposaline conditions (<10 PSU). The effect of long-term salinity changes (>5 days) or the effect of salinity >60 PSU on Alaria esculenta’s photosynthetic ability was not tested. The experiment was conducted in the Arctic, and the authors suggest that at extremely low water temperatures (1 to 5°C) macroalgal acclimation to rapid salinity changes could be slower than at temperate latitudes. It is therefore possible that Alaria esculenta maybe be able to acclimate to salinity changes more effectively and quicker in UK waters, however evidence for this is limited. Mytilus edulisMytilus edulis is found in a wide range of salinities from variable salinity areas (18 to 35 PSU) such as estuaries and intertidal areas to areas of more constant salinity (30 to 35 PSU) in the sublittoral (Connor et al., 2004). Furthermore, mussels in rock pools are likely to experience hypersaline conditions on hot days (Terry et al., 2024). Newell (1979) recorded salinities as high as 42 PSU in intertidal rock pools, suggesting that Mytilus edulis can tolerate hypersaline conditions. According to OBIS (2026), Mytilus edulis occurs in salinities ranging from 5 to 40 PSU. Over 57,000 records showed Mytilus edulis in the 5 to 10 PSU range, followed by over 52,000 records in the 30 to 35 PSU range. OBIS (2026) have no records of Mytilus edulis below 5 PSU. The number of records in the remaining salinity ranges (10 to 30 and 35 to 40 PSU) varied between 1,000 and 8,000. Sensitivity AssessmentBoth characteristic species have been shown to tolerate salinities above 40 PSU, with Alaria esculenta showing photosynthesis in experiments with salinities up to 50 PSU (Karsten, 2007) and Mytilus edulis tolerating salinities up to 42 PSU (Newell, 1979), all of which are within the range of the pressure benchmark level. However, this biotope has been recorded exclusively in full salinity (30 to 40 PSU) (Connor et al., 2004; JNCC, 2022). Therefore, a change from full to hypersaline conditions (>40 PSU) for a year could result in changes to the biotope. As a precaution, a resistance of ‘Medium’ is suggested, with a resilience of ‘High’ and a resultant sensitivity of ‘Low’. However, in the absence of direct evidence, the overall confidence in the assessment is 'Low'. | MediumHelp | HighHelp | LowHelp |
Salinity decrease (local) [Show more]Salinity decrease (local)Benchmark. A decrease in one MNCR salinity category above the usual range of the biotope or habitat (Salinity regime change pressure definition detail). EvidenceThe biotope has only been recorded from conditions of full salinity (Connor et al., 2004; JNCC, 2015, 2022). Intertidal examples of these biotopes will naturally experience fluctuations in salinity where evaporation increases salinity and inputs of rainwater reduces salinity. Species found in the intertidal likely have some form of behavioural or physiological adaptations to changes in salinity. Lüning (1990) suggest that kelps are stenohaline, their general tolerance to salinity as a phenotypic group covering 16 to 50 PSU over a 24-hour period. Optimal growth probably occurs between 30 to 35 PSU (MNCR category: Full Salinity) and growth rates are likely to be affected by periodic salinity stress. Alaria esculentaAccording to OBIS (2026), Alaria esculenta occurs in waters ranging from 15 to 40 PSU, with most records in the 30 to 35 PSU range. Karsten (2007) tested the photosynthetic ability of Alaria esculenta under acute 2 and 5-day exposures to salinity treatments ranging from 5 to 60 PSU. A control experiment was also carried at 34 PSU. Between 10 to 50 PSU, Alaria esculenta showed high photosynthetic ability at 83 to 94% of the control. Hypersaline treatments with 55 to 60 PSU led to a 30% reduction in photosynthetic ability, approx. 70% of the control level. At 5 PSU, Alaria esculenta showed a low photosynthetic ability at 15.8% of the control. After 5 days at 5 PSU, all Alaria esculenta specimens were bleached and none survived. Karsten (2007) suggested that Alaria esculenta photosynthetic ability is highly affected by acute exposure to hyposaline conditions (<10 PSU). The effect of long-term salinity changes (>5 days) or the effect of salinity >60 PSU on Alaria esculenta’s photosynthetic ability was not tested. The experiment was conducted in the Arctic, and the authors suggest that at extremely low water temperatures (1 to 5°C) macroalgal acclimation to rapid salinity changes could be slower than at temperate latitudes. It is therefore possible that Alaria esculenta maybe be able to acclimate to salinity changes more effectively and quicker in UK waters, however evidence for this is limited. Moreover, Sundene (1962) found that Alaria esculenta sporophytes grew poorly below 25 PSU. Lebrun et al. (2024) investigated the combined effects of warming, salinity, and light on four kelp species, including Alaria esculenta. For six weeks, kelps collected from Kongsfjorden, Norway, were exposed to an unmanipulated control treatment which had ambient seawater flowing into the tank at roughly 5.3°C, 33.8 PSU, with an irradiance of 47.8 µmol photons/m2/s, and three additional treatments: T1 = moderate warming (+3.3°C), reduced salinity (-2.5 PSU, and reduced light (-25% irradiance); T2 = stronger warming (+5.3°C), greater salinity reduction (-5 PSU), and lower light (-40% irradiance); and T3 = stronger warming alone (+5.3°C) without changes in salinity or irradiance. These conditions were chosen to reflect future global warming scenarios in which warming increases ice-melt, causing an addition of freshwater and suspended particles into the ocean. Chlorophyll-a declined in the control, reflecting normal seasonal changes, and showed similar patterns in T1 and T3. However, chlorophyll-a remained significantly higher in T2 (stronger warming with reduced salinity and light). Growth rates and carbon:nitrogen ratios were stable across the experiment. These results suggest that Alaria esculenta could potentially be resistant to the combined effects of global warming, reduced salinity, and reduced light. Mytilus edulisMytilus edulis is found in a wide range of salinities from variable salinity areas (18 to 35 PSU) such as estuaries and intertidal areas to areas of more constant salinity (30 to 35 PSU) in the sublittoral (Connor et al., 2004). In addition, Mytilus edulis thrives in brackish lagoons and estuaries, although, this is probably due to the abundance of food in these environments rather than the salinity (Seed & Suchanek, 1992). Moreover, Mytilus edulis was recorded to grow in a dwarf form in the Baltic Sea where the average salinity was 6.5 PSU (Riisgård et al., 2013). According to OBIS (2026), Mytilus edulis occurs in salinities ranging from 5 to 40 PSU. Over 57,000 records showed Mytilus edulis in the 5 to 10 PSU range, followed by over 52,000 records in the 30 to 35 PSU range. OBIS (2026) have no records of Mytilus edulis below 5 PSU. The number of records in the remaining salinity ranges (10 to 30 and 35 to 40 PSU) varied between 1,000 and 8,000. Mytilus edulis exhibits a defined behavioural response to reducing salinity, initially only closing its siphons to maintain the salinity of the water in its mantle cavity, which allows some gaseous exchange and therefore maintains aerobic metabolism for longer. If the salinity continues to fall the valves close tightly (Davenport, 1979; Rankin & Davenport, 1981). In the long-term (weeks) Mytilus edulis can acclimate to lower salinities (Almada-Villela, 1984; Seed & Suchanek 1992; Holt et al., 1998). Almada-Villela (1984) reported that the growth rate of individuals exposed to only 13 PSU reduced to almost zero but had recovered to over 80% of control animals within one month. Observed differences in growth are due to physiological and/or genetic adaptation to salinity. Experimental evidence demonstrates that Mytilus edulis can tolerate sustained reductions in salinity and can acclimate physiologically over short to medium timescales, albeit with measurable metabolic costs. Mytilus edulis is an osmoconformer and maintains its tissue fluids iso-osmotic (equal ionic strength) with the surrounding medium by mobilisation and adjustment of the tissue fluid concentration of free amino acids (e.g. taurine, glycine and alanine) (Bayne, 1976; Newell, 1989). But mobilizing amino acids may result in loss of protein, increased nitrogen excretion and reduced growth. Koehn (1983) and Koehn & Hilbish (1987) reported a genetic basis to adaptation to salinity. Decreased salinity has physiological effects on Mytilus edulis, decreasing the heart rate (Bahmet et al., 2005), reducing filtration rates (Riisgård et al., 2013), reducing growth rate (Gruffydd et al., 1984) and reducing the immune function (Bussell et al., 2008). Both Bahmet et al. (2005) and Riisgård et al. (2013) noted that filtration and heart rates return to normal within a number of days acclimation or a return to the original salinity. However, Riisgård et al. (2013) observed that mussels from an average of 17 PSU found it harder to acclimate between the salinity extremes than those from an average of 6.5 PSU. This observation may mean that mussels in a variable/ lower salinity environment are more able to tolerate change than those found at fully marine salinities. A sharp salinity change also induces a behavioural response to close the shell (Riisgård et al., 201) to maintain the salinity within the mantle cavity. In extreme low salinities, e.g. resulting from storm runoff, large numbers of mussels may be killed (Keith Hiscock pers. comm.). However, Bailey et al. (1996) observed very few mortalities when exposing Mytilus edulis to a range of salinities as low as 0 PSU for two weeks at a range of temperatures. It was also noted that there was a fast recovery rate. Bamber (2018) showed that mussels exposed to a sustained reduction in salinity from approx. 34 to 25 PSU over five days did not close their valves, and phagocytic activity was enhanced in individuals held at reduced salinity, suggesting maintained physiological function rather than acute stress. At the tissue and molecular level, exposure to reduced salinity induces membrane remodelling and tissue-specific metabolic responses that reflect plasticity rather than failure (Guinle et al., 2025). Clearance rates decreased under hyposaline conditions, condition indices declined, and lipid and gene expression profiles indicated energetic trade-offs associated with maintaining cellular integrity (Guinle et al., 2025). Similarly, Barrett et al. (2022) found that while low salinity (15 PSU) elicited progressive upregulation of stress- and osmoregulation-related genes, core physiological processes remained active, with marked stress responses only at very low salinities (5 PSU), indicating that functional limits occur well below typical UK coastal conditions. Responses to reduced salinity vary among life stages. May et al. (2017) reported substantial variation in metabolic responses to low salinity (20 PSU versus 32 PSU) across larval stages and tissue types, indicating that early life stages may be more sensitive than adults, but also that no single uniform response characterizes the species. Field observations from Scottish mussel farms indicate that early post-settlement stages may experience high mortality under moderately reduced salinity conditions. Spat mortality of up to 68.3% over 11 weeks was recorded at a site where salinity ranged from 21 to 27 PSU, compared with 28 to 32 PSU at a nearby control site, with peaks in mortality coinciding with the lowest salinity values (Broughton et al., 2019). Local adaptation further modifies tolerance. Both larvae and adults generally perform best at salinities similar to their native environment (Knöbel et al., 2021; Landes et al., 2015). Landes et al. (2015) reported highest growth rates and condition indices at intermediate salinities (approx. 25 to 30 PSU), while frequent salinity fluctuations reduced growth, indicating that stability may be as important as absolute salinity. Together, these studies indicate that Mytilus edulis can acclimate to sustained salinity reductions, but that energetic costs, life stage, and prior exposure influence performance. At the population and mussel bed scales, reduced salinity does not necessarily constrain persistence and may, in some contexts, enhance survival through indirect ecological mechanisms. In the Wadden Sea, natural mussel populations exhibited higher spat survival at lower salinity (approx. 20.7 PSU) than at higher salinity (approx. 24 PSU), likely due to reduced predation pressure from Asterias rubens, which is less tolerant of brackish conditions (Capelle et al., 2017). Long-term survival analyses of subtidal mussel beds similarly showed that beds in less-saline areas had survival rates comparable to intertidal beds, whereas beds in more saline subtidal areas experienced significantly lower persistence, again likely reflecting predation effects (Troost et al., 2022). Bed survival was also positively related to bed size, indicating that population structure and density interact with environmental conditions to influence resilience (Troost et al., 2022). However, extreme or combined stressors can exceed acclimation capacity. Johansson et al. (2024) reported increased hazard ratios for mussel bed persistence when salinity dropped below approx. 20.5 PSU for at least one day, indicating that short-term extreme freshening events can negatively affect bed survival even where moderate reductions are tolerated. Reduced salinity can also lower tolerance to additional stressors: Lysenko et al. (2015) found that mussels exposed to reduced salinity (15 PSU) had a diminished capacity to cope with crude oil contamination, while Nielsen et al. (2021) demonstrated that low salinity substantially reduced upper thermal tolerance, with mortality under heat stress increasing sharply at salinities of 5 to 15 PSU compared to 23 PSU. These findings indicate that, while Mytilus edulis can acclimate to salinity reductions in isolation, reduced salinity can interact synergistically with other pressures to increase vulnerability. Sensitivity AssessmentIR.HIR.KFaR.Ala plus associated sub-biotopes have been recorded exclusively in full salinity (30 to 40 PSU) (Connor et al., 2004; JNCC 2022). Karsten (2007) suggests that at salinities ranging from 10 to 50 PSU, Alaria esculenta photosynthetic ability was high. However, their experiment duration was only 5 days while the pressure benchmark duration is 1 year. At 5 PSU, Alaria esculenta showed a dramatic decline in photosynthetic ability and after 5 days specimens bleached and did not survive. Sundene (1962) noted that Alaria esculenta sporophytes grew poorly below 25 PSU. A decrease of one MNCR salinity scale to “Reduced” (18 to 30 PSU) may reduce growth rates but not cause mortality. Most of the evidence on Mytilus edulis considered short-term (days to weeks) impacts of changes in salinity. In short term exposures to reduced salinity, in which Mytilus edulis was shown to be capable of acclimation to changes in salinity, but experience energetic costs depending on prior exposure and life stage. Larval stages are more sensitive to reduced salinity than adults. Also, an acute (significant, rapid) drop in salinity is likely to be more detrimental than gradual change. Due to the evidence of physiological effects of reduced salinity on Alaria esculenta and Mytilus edulis over short timescales, and since KFaR.Ala biotopes are only found in full salinity, a precautionary resistance of ‘Medium’ is suggested with ‘High’ resilience and ‘Low’ sensitivity. | MediumHelp | HighHelp | LowHelp |
Water flow (tidal current) changes (local) [Show more]Water flow (tidal current) changes (local)Benchmark. A change in peak mean spring bed flow velocity of between 0.1 m/s and 0.2 m/s for more than one year (Water flow pressure definition). EvidenceAlaria esculenta dominates the sublittoral fringe in areas exposed to severe wave action or where water surges along the sides of gullies/steep bedrock faces (Lewis, 1964; Connor et al., 2004). The high wave exposure that defines IR.HIR.KFaR.AlaAnCrSp & IR.HIR.KFaR.Ala plus associated sub-biotopes damages other laminarians and generally excludes them. In less wave exposed locations Alaria esculenta is outcompeted by other Laminarians, e.g. Laminaria digitata and Laminaria hyperborea (Connor et al., 2004). This biotope is recorded within moderately strong (0.5 to 1.5 m/sec) to weak (<0.5m/sec) tidal streams. Therefore, elevated tidal flows (>3 m/sec) may increase Alaria esculenta dislodgement (Birkett et al., 1998). Increased tidal flow may remove fronds of Corallina officinalis, although calcification is thought to be an adaptation to mechanical damage (Littler & Kauker, 1984). Increases in water flow rate may facilitate the colonization of filter-feeding organisms within the understorey and IR.HIR.KFaR.Ala.Myt may dominate over IR.HIR.KFaR.Ala.Ldig. Decreases in water flow are likely to have the opposite effect (Connor et al. 2004). Changes in the water flow regimes under kelp canopies can modify larval supply and settlement (Eckman, 1983) and affect the growth and survival of Mytilus edulis (Eckman & Duggins, 1991). Mytilus edulis settlement has been found significantly higher near Alaria esculenta and is thought to increase beneath the canopy (Bégin et al., 2004). Therefore, any loss of Alaria esculenta, due to changes to local water movements, may affect Mytilus edulis recruitment. Mytilus edulisBlue mussels are active suspension feeders generating currents by beating cilia and are therefore not entirely dependent on water flow to supply food (organic particulates and phytoplankton). Therefore, they can survive in very sheltered areas, but water flow (due to tides, currents or wave action) can enhance the supply of food, carried from outside the area or resuspended into the water column. The growth rate of Mytilus edulis in relation to water flow was investigated by Langan & Howell (1994). They found that the growth rate over 24 days was 0.1, 1.8, 2.0, 1.9 and 1.5 mm at flow rates of 0, 0.01, 0.02, 0.04 and 0.08 m/s respectively. The only growth rate found to be significantly different was at zero flow. However, the pattern did follow that predicted by the “inhalant pumping speed” hypothesis that suggested maximal growth at water speeds of about 0.02 m/s and decreased growth rates at higher and lower speeds (Langan & Howell, 1994). Higher current speed brings food to the bottom layers of the water column, and hence near to the mussels, at a higher rate (Frechette et al., 1989). Frechette et al. (1989) developed a model based on measurements in the St. Lawrence River estuary (Québec). The model suggested that Mytilus edulis consumption rate depends on the flow of water. Widdows et al. (2002) found that there was no change in filtration rate of Mytilus edulis between 0.05 and 0.8 m/s. They noted that their finding contradicted earlier work that found a marked decline in filtration rates from 0.05 to 0.25 m/s (Newell, 1999; cited in Widdows et al., 2002) but suggested that the difference might be caused in differences in population studied, as the earlier work was based in the USA and their study used mussels from the Exe estuary in the UK. Widdows et al. (2002) also noted that above 0.8 m/s the filtration rate declined mainly because the mussels became detached from the substratum in the experimental flume tank. Widdows et al. (2002) noted that their results were consistent with field observations, as mussels show preferential settlement and growth in areas of high flow, such as the mouth of estuaries and at the base of power station cooling systems (Jenner et al., 1998). They also reported that Jenner et al. (1998; cited in Widdows et al., 2002) observed that biofouling of cooling water systems by mussels was only reduced significantly when mean current speeds reached 1.8 to 2.2 m/s and mussel biofouling was absent at >2.9 m/s. Increased flow rate increases the risk of mussel clumps being detached from the bed and transported elsewhere (Dare, 1976). Widdows et al. (2002) found that low-density mussel beds formed small clumps with a lower mass ratio of mussels attached to the substratum to increase anchorage. It is the strength of the byssal attachment that determines the mussel’s ability to withstand increases in flow rate. Flow rate itself has been shown to influence the strength and number of byssus threads that are produced by Mytilus edulis and other Mytilus spp., with mussels in areas of higher flow rate demonstrating stronger attachment (Dolmer & Svane, 1994; Alfaro, 2006). Dolmer & Svane (1994) estimated the potential strength of attachment for Mytilus edulis in both still water and flows of 1.94 m/sec, by counting the number of established byssus threads and measuring the strength of attachment of individual detached byssus threads. In still water the strength of the attachment was 21% of the potential strength whilst at 19.4 cm/sec it was 81% of the potential strength, suggesting that Mytilus edulis can adapt the strength of its attachment based on flow rate. Young (1985) demonstrated that byssus thread production and attachment increased with increasing water agitation. She observed the strengthening of byssal attachments by 25% within eight hours of a storm commencing and an ability to withstand surges up to 16 m/s. However, it was concluded that sudden surges may leave the mussels susceptible to being swept away (Young, 1985) as they need time to react to the increased velocity to increase the attachment strength. Mytilus edulis beds could therefore adapt to changes in water flow at the pressure benchmark. Individuals attached to solid substrata (rock) are likely to display more resistance than individuals attached to boulders, cobbles or sediment. For example, mussel reefs in the Wash, Morecambe Bay and the Wadden Sea are vulnerable to destruction by storms and tidal surges (Holt et al., 1998). Widdows et al. (2002) examined mussel beds in the mouth of the Exe estuary and along the coast at Exmouth. In flume tank studies between 0.1 and 0.35 m/s, the resuspension rate of sediment in mussel beds on sandy substrata was four and five times higher for areas with 25% and 50% mussel cover compared to bare sediment due to the increased turbulence and scouring around the mussels. However, at high mussel densities (100% cover) the beds remained stable (up to 0.35 m/s), with resuspension being about three times lower than areas with 0% cover, due to the high number of byssal attachments between individuals (Widdows et al., 2002). Where mussel beds occurred on pebble and sand substrata (mixed substrata) sediment erosion was lower than that of the 100% cover on the sandy substrata regardless of mussel density. Low density mussel beds formed small clumps with a lower mass ratio of mussels attached to the substratum to increase anchorage. In low density beds, increased scour resulted in some mussels detaching from the bed and in areas with 50% cover the erosion of the bed resulted in the burial of a large proportion of the mussels. The mussels returned to the surface afterwards and recovered in 1 to 2 days. Widdows et al. (2002) also noted a linear relationship between mussel bed density and sediment stability on cohesive mud substratum, taken from Cleethorpes, and exposed to currents of 0.15 to 0.45 m/s. Again, increased mussel cover increased sediment stability. Widdows et al. (2002) found that the mussel bed at Exmouth experienced a peak flow of 0.9 m/s before and after high water, which only reduced to 0.2 m/s at slack water. Capelle et al. (2019) provided experimental evidence that these density- and substratum-dependent effects also operate during the establishment phase of Mytilus edulis beds on soft sediments. In high-energy mudflat environments (mean flow velocity approx. 0.6 m/s), 100% of juveniles were dislodged in the absence of shell material on the substratum, whereas the addition of shells significantly reduced dislodgement. Increased mussel density further reduced losses, indicating that early bed stability on sedimentary substrata is strongly influenced by both substratum roughness and conspecific density. Water flow also affects the settlement behaviour of larvae. Alfaro (2005) observed that larvae settling in a low water flow environment can first settle and then detach and reattach displaying exploratory behaviour before finally settling and strengthening their byssus threads. However, larvae settling in high flow environments did not display this exploratory behaviour. Pernet et al. (2003) found that at high velocities, larvae of Mytilus spp. could not exercise much settlement preference. It was thought that when contact with suitable substratum is made the larvae probably secure a firm attachment. Demmer et al. (2022) showed that these flow-related constraints can extend beyond immediate settlement behaviour to influence local recruitment potential. Larval dispersal modelling of Mytilus edulis populations along the North Wales coast indicated low levels of self-recruitment at sites exposed to strong tidal currents, with peak velocities of approx. 2 m/s. This suggests that in high-flow environments, recovery of mussel beds following disturbance may be increasingly dependent on larval supply from adjacent populations rather than local retention. Long-term monitoring further indicates that relatively small differences in water flow can influence recruitment success over interannual timescales. Franz et al. (2019) analysed eleven years of settlement panel data from the south-western Baltic Sea, during which Mytilus edulis declined almost completely, and reported a negative relationship between mussel coverage and mean water current speed, within a relatively low flow range ( approx. 0 to 7 cm/s, 0 to 0.07 m/s). Reduced settlement was most evident where elevated current speeds coincided with unfavourable spring temperatures, indicating that flow effects on recruitment may interact with other environmental drivers rather than acting in isolation. Movement of larvae from low shear velocities, where they use their foot to settle, to high shear velocities where they use their byssal thread to settle was observed by Dobretsov & Wahl (2008). Sensitivity AssessmentThe biotope occurs from weak to moderately strong tidal flow. Hence, the characteristic species will probably not be affected by a change of 0.1 to 0.2 m/s in peak mean spring bed flow velocity. Therefore, resistance is assessed as ‘High’, resilience as ‘High’, and the biotope is assessed as ‘Not Sensitive’ at the benchmark level. Prolonged increase in flow could result in loss of the biotope due to reduced local recruitment and competition from other species. | HighHelp | HighHelp | Not sensitiveHelp |
Emergence regime changes [Show more]Emergence regime changesBenchmark. 1) A change in the time covered or not covered by the sea for a period of ≥1 year, or 2) an increase in relative sea level or decrease in high water level for ≥1 year. (Emergence regime change pressure definition). EvidenceAn increase in emergence will result in an increased risk of desiccation. Increased immersion may allow IR.HIR.KFaR.Ala biotopes to extend higher up the shore. However, Alaria esculenta forests will come under increased competition with Laminaria hyperborea in the shallow infralittoral. In this scenario IR.HIR.KFaR.Ala biotope distribution may shift on the shore, but the biotope structure will remain. Alaria esculenta may extend into the lower eulittoral in extremely wave exposed conditions. However, these marginal populations have a reduced age range in comparison to subtidal populations due to desiccation increasing mortality of Alaria esculenta at low tide. An increase in desiccation is likely to remove Alaria esculenta. The resultant loss of canopy would expose Corallina officinalis turf and macrofaunal crust to desiccation and/or damage by high light intensity (bleaching). Hawkins & Harkin (1985) noted that encrusting corallines and Corallina officinalis often die when their protective algal canopy is removed. Severe damage was noted in Corallina officinalis as a result of unusually hot and sunny weather in the UK summer 1983 (Hawkins & Hartnoll, 1985). Mytilus edulis beds are found across a wide range of shore heights, from the strandline down to the shallow sublittoral (Connor et al., 2004). Their upper limits are controlled by temperature and desiccation (Suchanek, 1978; Seed & Suchanek, 1992; Holt et al., 1998), while their lower limits are determined by predation, competition (Suchanek, 1978), and sand burial (Daly & Mathieson, 1977). Mussels occurring higher on the shore exhibit slower growth rates (Buschbaum & Saier, 2001) due to reduced feeding time and decreased food availability. It has been estimated that the point of zero growth occurs at 55% emergence (Baird, 1966), although this value may vary depending on local exposure conditions (Baird, 1966; Holt et al., 1998). However, increasing shore height increases mussel longevity due to reduced predation pressure (Seed & Suchanek, 1992; Holt et al., 1998), resulting in a broader range of age classes on the upper shore. The lower limit of Mytilus beds is primarily determined by predation from Asterias rubens and Carcinus maenas, which may increase as emergence decreases, potentially lowering the bed's lower limit or reducing the number of size classes and the age of mussels present at the lower edge of the bed (Saier, 2002). Sensitivity AssessmentResistance to this pressure is considered ‘Low’ with ‘High’ resilience, resulting in ‘Low’ sensitivity. | LowHelp | HighHelp | LowHelp |
Wave exposure changes (local) [Show more]Wave exposure changes (local)Benchmark. A change in near shore significant wave height of >3% but <5% for more than one year (Wave action pressure definition). EvidenceAlaria esculenta dominates the sublittoral fringe in areas exposed to severe wave action or where water surges along the sides of gullies (Lewis, 1964). A decrease in local wave height will increase spatial competition from other laminarians (Connor et al., 2004; JNCC, 2022). Increased wave exposure may remove fronds of Corallina officinalis, but calcification is thought to an adaptation to mechanical damage (Littler & Kauker 1984) and the fronds grow as a compact (short) turf in wave exposed conditions. IR.HIR.KFaR.Ala and its sub-biotopes occur in high energy sites from very exposed to moderately exposed. The sub-biotopes are separated based on wave exposure. KFar.Ala.Myt occurs predominantly on sub-littoral fringe bedrock in very exposed conditions. In extremely wave exposed conditions KFaR.Ala.Myt can extend to 15 m below chart datum where Alaria esculenta replaces Laminaria hyperborea as the assemblage dominant, but as depth increases Tubularia spp. becomes more abundant and Mytilus abundance decreases (Bégin et al., 2004, Connor et al., 2004; JNCC, 2022). KFaR.Ala.Ldig occurs predominately at very exposed to moderately wave exposed sites, where Laminaria digitata can spatially compete with Alaria esculenta, and represents an intermediate community between more exposed KFaR.Ala.Myt and pure Laminaria digitata (Ldig) (Connor et al., 2004; JNCC, 2022). Mytilus edulisA number of studies and reports have assessed the effects of water flows on blue mussel beds, but few were directly relevant to clumps of mussels. Mytilus edulis is able to increase the strength of their attachment to the substratum in more turbulent conditions (Price, 1982; Young, 1985). Young (1985) demonstrated an increase in strength of the byssal attachment by 25% within 8 hours of a storm commencing. When comparing mussels in areas of high flow rate and low flow rate those at a higher flow rate exhibit stronger attachments than those in the areas of lower flow (Dolmer & Svane, 1994; Alfaro, 2006). Dolmer & Svane (1994) found that in still water the strength of the attachment was 21% of the potential strength whilst at 1.94 m/sec it was 81% of the potential strength. Alfaro (2006) also noted that the individuals kept at higher water flows produce more byssal threads. The increased energy used for byssus production in the high flow environments may reduce the energy that is available for other biological activities. Whilst this clearly demonstrates the ability of mussels to adapt to the various conditions to avoid dislodgement, the mussels are unlikely to adapt instantly and a sudden increase in flow is likely to result in dislodgement (Young, 1985). Recent studies suggest that increased wave exposure does not necessarily result in reduced growth or performance of Mytilus edulis. Bergström et al. (2024) reported higher growth rates at more wave exposed sites in Sweden, indicating that increased water movement may enhance food delivery under some conditions. Similarly, Lukić et al. (2024) found no effect of wave exposure on growth rates in a 13-week mesocosm experiment conducted in Norway, where wave levels reflected local summer wind conditions (2.5 to 5 m/s). Widdows et al. (2002) examined mussel beds in the mouth of the Exe estuary and along the coast at Exmouth. Where the mussel beds occurred on sandy substratum the re-suspension rate was four and five times higher for areas with 25% and 50% mussel cover compared to bare sediment due to the increased turbulence and scouring around the mussels. In low density beds, this increased scour resulted in some mussels detaching from the bed and in areas with 50% cover the erosion of the bed resulted in the burial of a large proportion of the mussels. The mussels returned to the surface after 1 to 2 days and recovered. However, at high densities (100% cover) the beds remained stable, with re-suspension being about three times lower than areas with 0% cover, due to the high number of byssal attachments between individuals (Widdows et al., 2002). Where mussel beds occurred on pebble and sand substratum (mixed substratum) sediment erosion was lower than that of the 100% cover on the sandy substratum regardless of density despite experiencing flows of 0.9 m/s. The low-density mussel beds were observed to form small clumps with a lower mass ratio of mussels attached to the substratum to increase anchorage. Widdows et al. (2002) suggest that 100% mussel cover on sandy substrata reduces the risk of dislodgement. However, Harger & Landenberger (1971) suggest that growth in mussel beds results in fewer mussels being attached to the substratum and therefore strong seas can “roll up the whole mass of mud and mussels like a carpet and break it to pieces on the foreshore”. It was also noted that on gravelly substratum, single layer mussel beds incurred less damage in storm conditions than heavier multi-layered beds. Large-scale destruction of mussel beds has been reported in many areas such as the Wash, Morecambe Bay and the Wadden Sea (Holt et al., 1998). It appears that because of high wave exposure and destruction, reefs found in wave exposed areas are likely to be more dynamic (Nehls & Thiel, 1993). Furthermore, increased wave exposure leads to a higher risk of damage from drift logs (or other flotsam), which once they have destroyed a patch of mussels, leave the mussels around that patch at a higher risk of erosion (Seed & Suchanek, 1992). Mussels with high abundance of epizoic and epiphytic (e.g. barnacles and macroalgae) growing on mussels are also more susceptible to removal in areas of high wave exposure due to increased drag caused by these fouling organisms (Suchanek, 1985; Seed & Suchanek, 1992). However, mussel beds are prevalent in areas of high wave exposure suggesting a high resilience despite the destruction. Blue mussels display a high resistance to increases in water flow, but the oscillatory water movement that occurs on shores of higher wave exposure is likely to have a higher impact due to the ‘to and fro’ motion which is more likely to weaken the attachments. Westerbom & Jattu (2006) found that in subtidal mussel beds, mussel densities increased with increasing wave exposure. The highest biomass was found in areas of intermediate exposure, potentially due to the larger mussels being removed at high wave exposure levels. It was suggested that the lower densities found in more sheltered areas were due to low recruitment, early post-recruitment mortality, increased predation or stagnant settlement on rocks. Furthermore, it was also noted that high sedimentation, which is more prevalent in sheltered areas, as there is less energy for re-suspension, prevents colonization and result in the death of small mussels that are living close to the sediment surface by smothering and the clogging up of their feeding apparatus (Westerbom & Jattu, 2006). Therefore, colonization of new space in sheltered areas could be slow, particularly in areas where there is a low availability of adult mussels. An increase in wave exposure may increase density in subtidal beds (Westerbom & Jattu, 2006) unless there is a very sudden storm surge. Mussels on sedimentary substrata are exposed to a higher risk of dislodgement (Widdows et al., 2002). A decrease in wave exposure is likely to result in increased sedimentation and reduced densities (Westerbom & Jattu, 2006) although the risk of dislodgement will be greatly reduced creating more stable beds (Nehls & Thiel, 1993). The above evidence is variable as different studies have examined beds that differ in habitat, wave exposure, substratum and mussel density. However general trends can be seen. In rocky habitats, increased wave exposure allows mussel to dominate and form beds, especially where the rock surface has a low slope. Where the beds are patchy or damaged (from natural or human activities) they are more susceptible to further damage as a result of wave action or storms (Seed & Suchanek, 1992; Brosnan & Crumrine, 1994). Multi-layered mussel beds are less susceptible to damage, especially where only the surface layer is removed. It has been noted that the build-up of mussel mud (pseudofaeces) under the bed can reduce the attachment of the bed to the underlying substratum. But in areas of wave exposure, the flow of water through the bed will probably prevent the ‘mussel mud’ accumulating. On sedimentary habitats, which themselves occur in wave sheltered environments, the mussel beds stabilise the sediment surface (Widdows et al., 2002), especially at high percentage cover, although at low cover (e.g. in patchy beds) turbulent flow caused by the mussels may increase erosion of the sediment. Capelle et al. (2019) showed that on mudflats exposed to relatively high hydrodynamic energy (water flow of 0.6 m/s), 100% of juvenile Mytilus edulis were dislodged in the absence of shell material, whereas the addition of shell and increased mussel density significantly reduced losses. This suggests that on soft sediments, newly established or patchy beds may be more vulnerable to increased wave action. Coarse and mixed sediments were more stable, although Widdows et al. (2002) also noted that cohesive muds were also stabilised by mussel beds. Nevertheless, strong wave action or storms can roll up an entire bed or section of a bed (Harger & Landenberger, 1971), and presumably remove patches of mussels, and that multi-layered bed suffer more damage. In sedimentary wave sheltered habitats, the build-up of mussel muds may reduce attachment to the substratum and increase the susceptibility of the bed to wave action (Seed & Suchanek, 1992). The growth of other organisms on the mussels themselves, will increase drag and hence increase the possibility of damage due to wave action. In sheltered conditions, large macroalgae (e.g. kelps, fucoids) growing on mussels may result in removal of clumps of mussels. Sensitivity AssessmentThis biotope already occurs at the highest level of exposure, so it is unlikely that an increase in wave exposure would affect it. However, the abundance of Mytilus might decrease under wave action. A decrease in wave exposure could favour a transition from KFaR.Ala.Myt to KFaR.Ala.Ldig. However, it is also unlikely that any of these biotopes would be affected within a year (as per the pressure benchmark) unless the canopy were removed by another pressure, as kelp lifespans are longer than a year. Therefore, at the pressure benchmark level, this biotope is considered to have ‘High’ resistance to this pressure, with ‘High’ resilience by default (no disturbance to recover from) and is therefore ‘Not Sensitive’. Note: Kain (1975) demonstrated that recruitment rates vary with wave exposure in several kelp species including those that characterise these biotopes. It is therefore possible that a decrease in wave exposure for more than one year could change the relative abundances of Alaria esculenta and Laminaria digitata, resulting in a change in biotope. However, a change on this scale is beyond that of the pressure benchmark. | HighHelp | HighHelp | Not sensitiveHelp |
Chemical Pressures
Use [show more] / [show less] to open/close text displayed
| Resistance | Resilience | Sensitivity | |
Transition elements & organo-metal contamination [Show more]Transition elements & organo-metal contaminationBenchmark. Exposure of marine species or habitat to one or more relevant Transitional metal or organometal (e.g. TBT) contaminants via uncontrolled releases or incidental spills (Transitional metals and organometals pressure definition). EvidenceThis pressure is Not Assessed but evidence is presented where available. Very few studies have investigated whether these contaminants are harmful to kelp. Most studies on this topic instead focus on implications for human health and other trophic levels in kelp forest ecosystems. Several transition elements have been detected in Alaria esculenta tissues, including arsenic (As), cadmium (Cd), chromium (Cr), copper (Cu), lead (Pb), mercury (Hg), and nickel (Ni) (Roleda et al., 2019; Kreissig et al., 2021; Da Silva Junior et al., 2023; Jönsson & Nordberg, 2024), but their harmful effects on Alaria esculenta were not investigated. Cereja et al. (2026) studied the effects of copper on the golden kelp Laminaria ochroleuca and Mytilus edulis. They found that Laminaria ochroleuca significantly reduces copper (Cu) concentrations in the surrounding water. This effect was strong enough to increase Mytilus edulis survival compared to the treatment without Laminaria ochroleuca. However, this also resulted in a decrease in chlorophyll-a concentration, an increase in phaeophytin, and tissue bleaching, indicating physiological stress. After 15 days of exposure, Cu accumulation led to kelp mortality (Cereja et al., 2026). Johnston & Roberts (2009) conducted a meta-analysis, which reviewed 216 papers to assess how a variety of contaminants (including metal contamination) affected six marine habitats (including intertidal and subtidal reefs). A 30 to 50% reduction in species diversity and richness was identified from all habitats exposed to the contaminant types. Johnston & Roberts (2009) also highlighted that macroalgal communities are relatively tolerant to contamination, but that metal- and nutrient-impacted intertidal communities can have low diversity assemblages which are dominated by opportunistic and fast-growing species (Johnston & Roberts, 2009 and references therein). Mercury (organic > inorganic) is highly toxic to macrophytes (Bryan 1984; Cole et al. 1999). Mercury and copper were lethal at 0.05 mg/l and 0.1 mg/l respectively and toxic at 0.05 mg/l and 0.01 mg/l respectively in Laminaria hyperborea. Zinc and cadmium were lethal at 5 mg/l and 10 mg/l respectively. The presence of alginates in kelp tissue is thought to sequester heavy metals in a biologically unavailable form. It is likely that laminarians such as Alaria esculenta are relatively tolerant of heavy metals except at high concentrations at high levels. For a Rapid Evidence Assessment on the effects of 'Transitional elements & organometal' contaminants on Mytilus spp., see the full 'Mytilus evidence review'. | Not Assessed (NA)Help | Not assessed (NA)Help | Not assessed (NA)Help |
Hydrocarbon & PAH contamination [Show more]Hydrocarbon & PAH contaminationBenchmark. Exposure of marine species or habitat to one or more relevant hydrocarbon or polyaromatic hydrocarbon (PAH) contaminants via uncontrolled releases or incidental spills (Hydrocarbon & PAH pressure definition). EvidenceThis pressure is Not Assessed but evidence is presented where available. The mucilaginous coating on kelp fronds is thought to protect them from coatings of oil. Hydrocarbons in solution reduce photosynthesis and may be algicidal. Reduction in photosynthesis is dependent on the type of oil, its concentration and length of exposure, oil-water mixture and irradiance in experimental trials (Lobban & Harrison, 1994). Subtidal populations are only exposed to oil emulsions or oil adsorbed particles. Kelps are relatively insensitive to dispersants (Birkett et al. 1998) e.g. Laminaria digitata exposed to diesel oil at 0.130 mg/l reduced growth by 50% in a 2-year experiment. No growth inhibition was noted at 0.03 mg/l and the plants recovered completely in oil free conditions. Corallina officinalis, however, exhibited dramatic bleaching after the Sea Empress oil spill and died after the Torrey Canyon spill (Crump et al. 1999; Smith 1968). Encrusting corallines and Corallina officinalis recovered from the Sea Empress spill quickly, bleaching only affecting the fronds or surface of crustose forms. Grazing gastropods, e.g. limpets are highly intolerant of oil spillage and if not killed are narcotinized and washed offshore and/or consumed by predators. The lower littoral populations are likely to be most vulnerable to oil spill and sublittoral fringe would be particularly affected at low tide. Although Alara esculenta may not be affected severely, the articulated coralline turf may be lost but recover quickly although the red algae may be intolerant. Grazers such as limpets, barnacles and meiofaunal crustaceans may also be lost from the community. For a Rapid Evidence Assessment on the effects of 'Hydrocarbons and PAH' contaminants on Mytilus spp., see the full 'Mytilus evidence review'. | Not Assessed (NA)Help | Not assessed (NA)Help | Not assessed (NA)Help |
Synthetic compound contamination [Show more]Synthetic compound contaminationBenchmark. Exposure of marine species or habitat to one or more synthetic compound contaminants via uncontrolled releases or incidental spills (Synthetic compound contamination pressure definition). EvidenceThis pressure is Not Assessed but evidence is presented where available. There is currently Insufficient Evidence of harmful effects of synthetic compound contamination in the kelps that characterise this biotope. Studies that investigate the presence of these compounds in seafood, including kelps, focus on implications for human health (see Alvarez-Munoz et al., 2015) rather than their effects on the species or ecosystems themselves. However, Anacleto et al. (2017) did investigate the effects of a range of pollutants on Laminaria digitata health but found no significant reduction in photosynthetic activity in response to pesticides (diflubenzuron and lindane). Cole et al. 1999 suggest that macrophytes are generally intolerant of herbicides such as atrazine, simazine, diuron and linuron e.g. atrazine was lethal to Laminaria hyperborea sporophytes at 1mg/l and suppressed growth at 0.01 mg/l (Hopkin & Kain, 1978). Smith (1968) noted that Corallina officinalis was killed in areas of heavy spraying after the Torrey Canyon oil spill and affected at 6 m depth in areas of high wave action. High water specimens were more affected than low water specimens, presumably because they are emersed for longer and had more contact with oil and dispersants. Hiscock & Hoare (1975) noted that almost all red algal species and many animal species were absent from Amlwch Bay in North Wales adjacent to an acidified halogenated effluent. Red algae have also been found to be sensitive to oil spill dispersants (O'Brien & Dixon, 1976). Gastropods are known to be highly sensitive to endocrine disrupters such as TBT. Crustaceans (e.g. amphipods, isopods, ostracods, copepods and barnacles) are also susceptible to endocrine disruption by synthetic chemicals. It is therefore likely that some taxa within this biotope, especially grazing invertebrates and meiofauna will be intolerant of synthetic chemical contamination. For a Rapid Evidence Assessment on the effects of 'Synthetic compound' contaminants on Mytilus spp., see the full 'Mytilus evidence review'. | Not Assessed (NA)Help | Not assessed (NA)Help | Not assessed (NA)Help |
Radionuclide contamination [Show more]Radionuclide contaminationBenchmark. An increase in 10µGy/h above background levels (Radionuclides contamination pressure definition). EvidenceNo evidence | No evidence (NEv)Help | Not relevant (NR)Help | No evidence (NEv)Help |
Introduction of other substances [Show more]Introduction of other substancesBenchmark. Exposure of marine species or habitat to one or more relevant "other" substances (solid, liquid or gas) contaminants via uncontrolled releases or incidental spills (Introduction of other substances pressure definition). EvidenceThis pressure is Not assessed. | Not Assessed (NA)Help | Not assessed (NA)Help | Not assessed (NA)Help |
De-oxygenation [Show more]De-oxygenationBenchmark. Exposure to dissolved oxygen concentration of less than or equal to 2 mg/l for one week (a change from WFD poor status to bad status) (deoxygenation pressure definition). EvidenceReduced oxygen concentrations have been shown to inhibit both photosynthesis and respiration in macroalgae (Kinne, 1977). Despite this, macroalgae are thought to buffer the environmental conditions of low oxygen, thereby acting as a refuge for organisms in oxygen depleted regions especially if the oxygen depletion is short-term (Frieder et al., 2012). A rapid recovery from a state of low oxygen is expected if the conditions are transient, which is likely given the wave exposure levels of IR.HIR.KFaR.Ala and its sub-biotopes. If dissolved oxygen concentrations drop below 4 mg/l, negative effects on these organisms may occur, with more severe adverse effects expected below 2 mg/l (Cole et al., 1999). Reduced oxygen levels are likely to inhibit photosynthesis and respiration but not cause a loss of the macroalgae population directly. However, small invertebrate epifauna may be lost, causing a reduction in species richness. Mytilus edulis is capable of anaerobic metabolism. In aerial exposure (emersion) the mussel closes its valves, resulting in a low rate of oxygen exchange and consumption, and conservation of energy (Widdows et al., 1979a; De Zwaan & Mathieu 1992). Mytilus edulis is regarded as euryoxic, tolerant of a wide range of oxygen concentrations including zero (Zandee et al., 1986; Wang & Widdows, 1991; Gosling, 1992; De Zwaan & Mathieu, 1992; Diaz & Rosenberg, 1995; Gray et al., 2002). Theede et al., (1969) reported LD50of 35 days for Mytilus edulis exposed to 0.21 mg/l O2 at 10°C, which was reduced to 25 days with the addition of sulphide (50 mg/l Na2S·9H2O). Jorgensen (1980) observed, by diving, the effects of hypoxia (0.2 to 1 mg/l) on benthic macrofauna in marine areas in Sweden over a 3 to 4-week period. Mussels were observed to close their shell valves in response to hypoxia and survived for 1 to 2 weeks before dying (Cole et al., 1999; Jorgensen, 1980). All life stages show high levels of tolerance to low oxygen levels. Mytilus edulis larvae, for example, are tolerant down to 1.0ml/l, and although the growth of late stage larvae is depressed in hypoxic condition, the settlement behaviour does not seem to be affected (Diaz & Rosenberg 1995). Based on the available evidence Mytilus edulis are considered to be resistant to periods of hypoxia and anoxia although sublethal effects on feeding and growth may be expected. Experimental studies demonstrate that exposure to hypoxia at concentrations around the benchmark can induce substantial sublethal physiological and molecular responses in Mytilus edulis, even where mortality does not occur. Tang & Riisgård (2018) showed that respiration rates declined gradually as dissolved oxygen decreased from 9 to 2 mg O₂/L, with only a approx. 25% reduction in respiration despite a 78% decline in oxygen availability, while filtration rates remained high. However, at concentrations below approx. 2 mg O₂/L mussels progressively closed their valves, resulting in rapid reductions in both filtration and respiration rates, indicating a shift away from normal aerobic metabolism and an energy-conserving response. Short-term hypoxia also triggers pronounced cellular and transcriptional responses. Hall et al. (2023) reported major changes in whole-mussel transcriptomes within the first four hours of hypoxia exposure, particularly in pathways associated with metabolism, cellular organisation and environmental sensing. In juvenile mussels, hypoxia caused significant under-expression of transcripts associated with byssal thread production, suggesting reduced attachment capacity and an increased risk of detachment under physically dynamic conditions. At the cellular level, severe hypoxia and subsequent reoxygenation trigger strong stress responses associated with cell damage and repair: Falfushynska et al. (2020) found that exposure to hypoxia for one to six days activated molecular pathways linked to programmed cell death, with responses further amplified during reoxygenation, indicating that recovery from hypoxia can itself place additional physiological stress on mussels. Mitochondrial responses underpin much of this species’ hypoxia tolerance. Short-term hypoxia-reoxygenation experiments indicate that Mytilus edulis possesses intrinsic mitochondrial mechanisms that mitigate oxidative damage and maintain respiratory efficiency during oxygen stress (Sokolov et al., 2021), although additional evidence suggests that hypoxia-reoxygenation also induces mitochondrial injury requiring activation of protective processes such as mitophagy (the selective removal of damaged mitochondria) and protein degradation to maintain cellular function (Steffen et al., 2020). Together, these studies indicate that while adult mussels tolerate hypoxia through metabolic plasticity, this tolerance is associated with energetic costs and cellular stress responses. The duration and severity of hypoxic exposure strongly influence outcomes. Sustained hypoxia below approx. 0.7 to 0.8 mg O₂/l for 16 days resulted in a marked decline in survival, with survival dropping from approx. 80% to <38% under prolonged exposure (Li et al., 2022), indicating thresholds beyond which tolerance is exceeded. At less severe concentrations, longer exposures can still impair condition and recovery. Kamermans & Saurel (2022) reported reduced body condition indices under low oxygen saturation (30 to 50%) compared to normoxia, while Mredul et al. (2024) showed that a seven-day exposure to approx. 2 mg O₂/l inhibited normal post-spawning mitochondrial recovery, suggesting potential for increased post-spawning mortality. Hypoxia can also interact with other pressures to exacerbate negative effects. Nielsen et al. (2021) showed that reduced salinity lowered tolerance to heat stress, with substantially higher mortality under combined low oxygen and elevated temperature conditions compared to single-stressor exposures. Field-based evidence supports these experimental findings. Analysis of long-term data from the Wadden Sea (1993 to 2022) found no relationship between short hypoxic events (<2 mg O₂/l) and mussel bed longevity in isolation, but reported increased hazard ratios where hypoxia coincided with elevated temperature (>6.9°C) and reduced salinity (< 20.5 PSU) (Johansson et al., 2024). Together, these studies indicate that while Mytilus edulis can generally tolerate hypoxia alone, reduced oxygen availability can increase vulnerability to other pressures. Sensitivity also varies among life stages and across generations. Hypoxia had little effect on fertilization success or larval shell length but increased embryo deformity rates, with partial mitigation where parents were previously acclimated to hypoxia, indicating transgenerational plasticity but incomplete buffering of effects (Kong et al., 2019). Sensitivity AssessmentNo evidence of mortality was found in any characteristic species. Sublethal effects were found, such as reduced photosynthesis and respiration in macroalgae, and detrimental behavioural changes in Mytilus edulis such as reduced respiration and feeding activity. However, at the pressure benchmark level (1-week exposure to oxygen concentrations of ≤2 mg/l), resistance and resilience of these biotopes are considered to be ‘High’ and so sensitivity is assessed as ‘Not Sensitive’. | HighHelp | HighHelp | Not sensitiveHelp |
Nutrient enrichment [Show more]Nutrient enrichmentBenchmark. Increased levels of the elements nitrogen, phosphorus, silicon, and iron in the marine environment compared to background concentrations (Nutrient enrichment pressure definition). EvidenceEutrophication is associated with loss of perennial algae and replacement by mussels or opportunistic algae (Fletcher 1996). Johnston & Roberts (2009) conducted a meta-analysis that reviewed 216 papers to assess how a variety of contaminants (including sewage and nutrient loading) affected 6 marine habitats (including intertidal and subtidal reefs). A 30 to 50% reduction in species diversity and richness was identified from all habitats exposed to the contaminant types. Johnston & Roberts (2009) also highlighted that macroalgal communities are relatively tolerant to contamination, but that metal and nutrient impacted intertidal communities can have low diversity assemblages which are dominated by opportunistic and fast-growing species (Johnston & Roberts, 2009 and references therein). Alaria esculentaSilva et al. (2022) demonstrated that nutrient availability influences the response of Alaria esculenta gametophytes to temperature and light. They used a full factorial experiment to test the combined effects of nutrient availability, temperature, and light intensity on Alaria esculenta gametophytes. The experiment crossed three irradiance levels (0.5, 35 and 100 μmol photons m²/s), two temperatures (5°C control and 9°C future-warming treatment), and two nutrient regimes: low nutrients (2 μM N and 0.2 μM P) and an unspecified high-nutrient treatment simulating increased inputs from mixing, river discharge, and permafrost melt. Gametophyte density was generally lower under high nutrient conditions than under low nutrient conditions, regardless of temperature. Under high nutrient conditions, densities were broadly similar across temperatures and low and medium light treatments, while high light resulted in reduced densities, particularly at 9°C. These findings indicate that responses of Alaria esculenta gametophytes to higher nutrient availability may be exacerbated by higher temperatures and light availability. Mytilus edulisNutrient enrichment may impact mussel beds by altering the biomass of phytoplankton and macroalgae. At low levels, nutrient enrichment may stimulate the growth of phytoplankton used as food - a potentially beneficial effect. In the Wadden Sea, where fishing had caused the destruction of the local population of Sabellaria spinulosa, Mytilus edulis was able to colonize, partly because of the increase in coastal eutrophication (Maddock, 2008). This pattern is consistent with longer-term observations from the Wadden Sea, where mussel reefs established during the last century expanded in size and number following the decline of native oyster reefs, with eutrophication considered to have augmented mussel growth and persistence at these sites (Reise et al., 2025). Conversely, Dinesen et al. (2011) observed that a reduction in nutrient loading to comply with the WFD resulted in a decrease of mussel biomass in estuaries. Recent experimental and historical evidence supports the conclusion that moderate nutrient enrichment can enhance food availability and mussel biomass without causing direct negative effects. Carrier-Belleau et al. (2024) exposed transplanted mussels to sustained nutrient enrichment (N = 10.47, P = 1.95, K = 2.20 mmol/day) over periods of 6.5, 10.5 and 15 weeks in a field experiment in Canada and found no effects on chlorophyll-a biomass, microbial activity, oxygen uptake or mussel mortality attributable to nutrient addition alone. Although mortality varied across exposure periods, this was not consistently linked to nutrient enrichment, and mussels showed no evidence of impaired physiological function under elevated nutrient supply. Long-term historical reconstructions from the Wadden Sea similarly indicate that periods of elevated nutrient availability were associated with widespread distribution and high biomass of Mytilus edulis, with Reise & Buschbaum (2017, cited in Ricklefs et al., 2020) identifying eutrophication-driven food availability as a key factor underlying mussel stock recovery and expansion during the mid- to late-20th century. Analyses of archived material from the Baltic Sea indicate that reductions in nutrient loading between 1993 and 2016 were associated with declines in mussel size, biomass and condition, consistent with food limitation following mitigation of eutrophication (Liénart et al., 2021). High levels of enrichment may stimulate algal blooms and macroalgal growth. The growth of macrophytes on the mussel beds may result in increased drag on the mussel bed and hence increase susceptibility to damage from wave action and/or storms (see changes in wave exposure pressure). Algal blooms may die off suddenly, causing de-oxygenation (see de-oxygenation pressure) where the algae decompose on the seabed. The thresholds at which these blooms occur depend on site-specific conditions and be mitigated by the degree of mixing and tidal exchange. Some algae have been shown to negatively affect Mytilus edulis when present in high concentrations. For example, blooms of the algae Phaeocystis sp., have been observed to block the mussel's gills when present in high concentrations reducing clearing rates, and at high levels, they caused a complete cessation of clearance (Smaal & Twisk, 1997). Blockage of the gills is also likely to reduce ingestion rates, prevent growth and cause reproductive failure (Holt et al., 1998). Other species known to negatively impact Mytilus edulis are Gyrodinium aureolum (Tangen, 1977; Widdows et al., 1979b) and a non-flagellated chrysophycean alga (Tracey, 1988). The accumulation of toxins from algal blooms has also been linked to outbreaks of paralytic shellfish poisoning resulting in the closure of shellfish beds (Shumway, 1990). However, experimental evidence indicates that such impacts of harmful algal blooms are strongly context-dependent. De Rijcke et al. (2015) showed that short-term (48-hour) exposure of larvae to high concentrations of harmful algae increased immune activity, indicating a physiological response to algal stress rather than direct toxicity at environmentally realistic concentrations. Modelling and field studies suggest that very high phytoplankton biomass may reduce growth through impaired food quality or digestive efficiency when chlorophyll-a concentrations exceed approx. 8 µg/l, although these effects are difficult to separate from covarying environmental drivers such as salinity (Larsen et al., 2018). Evidence from aquaculture-associated environments further suggests that nutrient enrichment can co-occur with additional stressors that affect mussel health. Nippard & Ciocan (2019) reported poor tissue condition and widespread (90% of samples) histological indicators of stress in mussels collected near a salmon farm, including haemocyte infiltration (indicative of immune activation), lipofuscin accumulation (associated with cellular stress and ageing) and possible neoplasms (abnormal tissue growth) in addition to increased parasites. However, these effects were associated with contaminant exposure in farm effluent, including heavy metal exposure, rather than nutrient enrichment alone, highlighting the importance of co-occurring pressures in determining biological responses. Several studies highlight the role of Mytilus edulis as both a responder to and mediator of nutrient enrichment. Mussel beds and farms can remove significant quantities of nitrogen from eutrophic systems through filtration and biodeposition, supporting their use in eutrophication mitigation strategies (Weldrick & Jelinski, 2016; Kotta et al., 2020). While mussels are widely used as bioindicators of nutrient loading, there is little evidence that nutrient enrichment at levels consistent with good ecological status causes direct adverse effects on adult mussels themselves (Reichwaldt & Ghadouani, 2016). Observed declines or degradation of subtidal mussel beds in some regions are more strongly associated with interacting pressures such as fishing disturbance, invasive species and long-term environmental instability rather than nutrient enrichment alone (Ricklefs et al., 2020). Sensitivity AssessmentEvidence shows that Alaria esculenta gametophyte density can be reduced by elevated nutrient levels (Silva et al., 2022), and this effect can be more pronounced in clearer waters with more available light. However, no evidence was found of nutrient loading negatively affecting the sporophyte stage of Alaria esculenta, so it may only affect the recruitment of juveniles rather than the health or survival of mature kelps. Mytilus edulis seems to be resistant to this pressure. As a precaution, due to the effects of elevated nutrients on Alaria esculenta gametophytes, resistance is assessed as ‘Medium’, resilience as ‘High’, and sensitivity as ‘Low’ in a worst-case scenario where elevated nutrient levels persist for over a year. If the pressure is removed within the timescale of Alaria esculenta’s recruitment cycle, the biotope would be considered as ‘Not Sensitive’. Confidence in this assessment is ‘Medium’ due to the lack of further evidence. | MediumHelp | HighHelp | LowHelp |
Organic enrichment [Show more]Organic enrichmentBenchmark. A deposit of 100 gC/m2/yr (Organic enrichment pressure definition). EvidenceOrganic enrichment is associated with eutrophication, increased siltation and turbidity (Fletcher 1996). Eutrophication is associated with loss of perennial algae and replacement by mussels or opportunistic algae (Fletcher 1996). Johnston & Roberts (2009) conducted a meta-analysis that reviewed 216 papers to assess how a variety of contaminants (including sewage and nutrient loading) affected six marine habitats (including intertidal and subtidal reefs). A 30 to 50% reduction in species diversity and richness was identified from all habitats exposed to the contaminant types. Johnston & Roberts (2009) also highlighted that macroalgal communities are relatively tolerant to contamination, but that contaminated intertidal communities can have low diversity assemblages which are dominated by opportunistic and fast-growing species (Johnston & Roberts, 2009 and references therein). Due to the high wave exposure that defines this biotope, it is likely that additional organic input to the system may be dispersed out of the biotope’s local vicinity (Johnston & Roberts, 2009). Increased nutrients may favour Mytilus edulis which may increase cover and abundance. Mytilus edulisMytilus edulis has been recorded in areas around sewage outflows (Akaishi et al. 2007; Lindahl & Kollberg, 2008; Nenonen et al. 2008; Giltrap et al. 2013) suggesting that they are highly tolerant of the increase in organic material that would occur in these areas. A number of studies have also highlighted the ability of Mytilus edulis to utilise the increased volume of organic material available at locations around salmon farms. Reid et al. (2010) noted that Mytilus edulis could absorb organic waste products from a salmon farm with great efficiency. Increased shell length, wet meat weight, and condition index were shown at locations within 200 m from a farm in the Bay of Fundy allowing a reduced time to market (Lander et al., 2012). It has been shown that regardless of the concentration of organic matter Mytilus edulis will maintain its feeding rate by compensating with changes to filtration rate, clearance rates, production of pseudofaeces and absorption efficiencies (Tracey, 1988; Bayne et al., 1993; Hawkins et al., 1996). Tolerance to organic enrichment is context-dependent and may be reduced under conditions where organic material accumulates within sediments and oxygen availability is restricted. Experimental burial of Mytilus edulis beneath organically enriched sediments resulted in significantly elevated mortality within days, particularly under fine sediments with high organic content and elevated temperatures, where mortality exceeded 50% within short burial durations and increased further with prolonged burial, up to 80% after 32 days (Cottrell et al., 2016). The authors suggested that pathogenic infection associated with microbial activity in organically enriched sediments, combined with burial-induced hypoxia and increased metabolic demand at higher temperatures, was a key driver of mortality. These findings indicate that while mussels tolerate elevated organic matter in well-flushed environments, organic enrichment that leads to sediment accumulation, hypoxia or microbial proliferation may have negative effects. Evidence from biomonitoring studies indicates that chronic exposure to organically enriched and contaminated environments may be associated with sublethal health effects. Mussels sampled near a salmon aquaculture site in Loch Creran exhibited a high prevalence of tissue-level indicators of stress, with 90% of tissue samples showing one or more signs of pollutant-induced pathology, including immune cell infiltration, accumulation of cellular waste products associated with stress and ageing, parasitic infection and abnormal tissue growth (Nippard & Ciocan, 2019). While such effects do not necessarily translate into immediate mortality or population decline, they suggest potential longer-term consequences for condition, disease susceptibility and resilience under sustained organic loading. Exposure to certain bloom-forming algae has been shown to elicit physiological responses in early life stages. Short-term exposure of larvae to Pseudo-nitzschia multiseries and Prorocentrum lima at elevated concentrations increased immune activity, indicating a stress response even over brief exposure periods (De Rijcke et al., 2015), for example. At the extreme end of organic enrichment, exceptionally high phytoplankton biomass has been associated with mass mortality events in mussels, attributed to hypoxia and physical clogging of the gills during intense bloom conditions (Richardson et al., 2021). Sensitivity AssessmentThe wave exposure levels of this biotope would likely disperse organic matter away from the biotope. Resistance and resilience are deemed to be ‘High’, so the biotope is deemed to be ‘Not Sensitive’. | HighHelp | HighHelp | Not sensitiveHelp |
Physical Pressures
Use [show more] / [show less] to open/close text displayed
| Resistance | Resilience | Sensitivity | |
Physical loss (to land or freshwater habitat) [Show more]Physical loss (to land or freshwater habitat)Benchmark. A permanent loss of existing saline habitat within the site (Physical loss pressure definition). EvidenceAll marine habitats and benthic species are considered to have a resistance of ‘None’ to this pressure and to be unable to recover from a permanent loss of habitat (resilience is ‘Very Low’). Sensitivity within the direct spatial footprint of this pressure is therefore ‘High’. Although no specific evidence is described confidence in this assessment is ‘High’, due to the incontrovertible nature of this pressure. | NoneHelp | Very LowHelp | HighHelp |
Physical change (to another seabed type) [Show more]Physical change (to another seabed type)Benchmark. Permanent change from sedimentary or soft rock substrata to hard rock or artificial substrata, or vice versa (Physical change in subtratum type pressure definition). EvidenceIf rock substrata were replaced with sedimentary substrata this would represent a fundamental change in habitat type, which Alaria esculenta would not tolerate (Birkett et al., 1998). The biotope would be lost. Sensitivity assessment. Resistance to the pressure is considered ’None‘, and resilience ’Very low‘ or ‘None’. The sensitivity of this biotope to change from hard rock or artificial substrata to sedimentary or soft rock substrata is assessed as ’High’. | NoneHelp | Very LowHelp | HighHelp |
Physical change (to another sediment type) [Show more]Physical change (to another sediment type)Benchmark. Permanent change in one Folk class (based on UK SeaMap simplified classification) (Physical change in sediment type pressure definition). EvidenceNot relevant to hard rock biotopes. | Not relevant (NR)Help | Not relevant (NR)Help | Not relevant (NR)Help |
Habitat structure changes - removal of substratum (extraction) [Show more]Habitat structure changes - removal of substratum (extraction)Benchmark. The extraction of substratum to 30 cm (where substratum includes sediments and soft rock but excludes hard bedrock) (Removal of substratum pressure definition). EvidenceNot relevant to hard rock biotopes. | Not relevant (NR)Help | Not relevant (NR)Help | Not relevant (NR)Help |
Abrasion / disturbance of the surface of the substratum or seabed [Show more]Abrasion / disturbance of the surface of the substratum or seabedBenchmark. Damage to surface features (e.g. species and physical structures within the habitat) (Surface abrasion/disturbance pressure definition). EvidenceAlaria esculentaIf exposed to moorings, groundings, or passing fishing gear, the resultant abrasion may result in the physical removal of a proportion of the Alaria esculenta canopy depending on the scale of the impact, although no evidence of these specific disturbances was found. However, Ronowicz et al. (2022) found morphological differences in Alaria esculenta between 5 and 10 m depth at sites of varying levels of glacial influence. At the site with the most glacial influence (frequent iceberg scour and the highest load of suspended sediment), Alaria esculenta plants were significantly shorter, had reduced biomass, and had less morphological variability within the population. The authors observed no significant difference in these metrics between the non-impacted and intermediate-impacted (high sediment input alone) sites, suggesting that ice scour was the cause of the reduced size of Alaria esculenta at the highest-impacted site. Mytilus edulisActivities resulting in abrasion and disturbance can either directly affect Mytilus edulis by crushing them or indirectly affect them by the weakening or breaking of their byssus threads, making them vulnerable to displacement (Denny, 1987) where they are unlikely to survive (Dare, 1976). In addition, abrasion and sub-surface damage may attract mobile scavengers and predators including fish, crabs, and starfish to feed on exposed, dead and damaged individuals and discards (Kaiser & Spencer, 1994; Ramsay et al., 1998; Groenewold & Fonds, 2000; Bergmann et al., 2002). This effect will increase predation pressure on surviving damaged and intact Mytilus edulis when submerged. A number of activities or events that result in abrasion and disturbance and their impacts on mussel beds are described below, based on the review by Mainwaring et al. (2014). Brosnan & Crumrine (1994) noted that mussels that occupied hard substrata but did not form beds were also adversely affected. Although only at low abundance (2.5% cover), all mussels were removed by trampling within four months. Brosnan & Crumrine (1994) noted that mussels were not common and confined to crevices in heavily trampled sites. Similarly, the mussel bed infauna (e.g. barnacles) was adversely affected and were crushed or lost with the mussels to which they were attached. However, Beauchamp & Gowing (1982) did not observe any differences in mussel density between sites that differed in visitor use. Paine & Levin (1981) examined natural patch dynamics in a Mytilus californianus bed in the USA. They suggested that it may take up to seven years for large barren patches to recover. However, chronic trampling may prevent recovery altogether. This would result in a shift from a mussel-dominated habitat to one dominated by an algal turf or crust (Brosnan & Crumrine, 1994), completely changing the biotope. However, a small period of trampling could allow communities to recover at a similar rate to that of natural disturbance as the effects are similar. The associated epifauna and epiflora suffer the greatest amount of damage as they are the first organisms that a foot makes contact with (Brosnan & Crumrine, 1994). The loss of epifauna and epiflora could initially be of benefit to the mussel bed, despite the obvious decrease in species diversity, as there will be a decrease in drag for the mussels reducing the risk of dislodgement (Witman & Suchanek 1984) and freeing up more energy for growth and reproduction. However, it is likely that after continued trampling this effect will be minimal compared with the increased risk of dislodgement caused by trampling. The collision of objects with the bed, such as wave driven logs (or similar flotsam), is known to cause the removal of patches of mussels from mussel beds (Seed & Suchanek, 1992; Holt et al., 1998). When patches occur in mussel beds a good recruitment could result in a rapid recovery or the patch may increase in size through the weakening of the byssus threads of the remaining mussels leaving them vulnerable to erosion from storm damage (Denny, 1987). Damage in areas of high wave exposure is likely to result in increased erosion and a patchy distribution although recruitment may be high. In sheltered areas, damage may take a lot longer due to limited larval supply, although the frequency of destruction through wave driven logs would be less than in high wave exposure. Similar effects could be observed through the grounding of a vessel, the dropping of an anchor or the laying of a cable, although the scale of damage clearly differs. Shifting sand is known to limit the range of Mytilus edulis through burial and abrasion (Daly & Mathieson, 1977). Sensitivity AssessmentAbrasion from boats and trampling are possible in the sublittoral fringe where KFaR.Ala.Myt occurs. Both characterising species are deemed to have ‘Low’ resistance to abrasion, with ‘High’ resilience and ‘Low’ sensitivity. | LowHelp | HighHelp | LowHelp |
Penetration or disturbance of the substratum subsurface [Show more]Penetration or disturbance of the substratum subsurfaceBenchmark. Damage to sub-surface features (e.g. species and physical structures within the habitat) (Sub-surface penetration pressure definition). EvidenceNot relevant to hard rock biotopes. | Not relevant (NR)Help | Not relevant (NR)Help | Not relevant (NR)Help |
Changes in suspended solids (water clarity) [Show more]Changes in suspended solids (water clarity)Benchmark. A change in one rank on the WFD (Water Framework Directive) scale, e.g. from clear to intermediate for one year (Suspended sediment pressure definition). EvidenceSuspended Particle Matter (SPM) concentration has a linear relationship with sub surface light attenuation (Kd) (Devlin et al., 2008). Light penetration influences the maximum depth at which kelp species can grow, and it has been reported that laminarians grow at depths at which the light levels are reduced to 1% of incident light at the surface. Maximal depth distribution of laminarians varies from 100 m in the Mediterranean to only 6 to 7 m in the silt-laden German Bight. In European Atlantic waters, the depth limit is typically 35 m. The kelp Ecklonia radiata has shown a decrease of 50% photosynthetic activity when turbidity increases by 0.1/m (light attenuation coefficient = 0.1 to 0.2/m; Staehr & Wernberg, 2009). An increase in water turbidity would therefore likely affect the photosynthetic ability of Alaria esculenta and over time, possibly decrease their abundance and density. Alaria esculentaAlaria esculenta is not found in areas of siltation and sediment scour (Birkett et al., 1998). Increased siltation and sediment scour inhibits photosynthesis and algal growth, interfere with spore or larval recruitment plus smother germlings and gametophytes (Fletcher, 1996). However, the high degree of wave exposure that defines this biotope is likely to clear suspended sediments relatively quickly. If low water clarity is persistent and wave exposure decreased, then low energy silted kelp biotopes (IR.LIR.K) may proliferate. Once siltation returns to its pre-disturbance level the biotope is likely to recover its canopy within a year and the rest of the community in no more than five years. Increased turbidity is likely to reduce the depth to which Alaria esculenta can grow. However, an increase of one level in WFD water clarity scale for a period of one year is unlikely to affect the population since Alaria esculenta’s lower limit, is generally determined by competition from other Laminarians rather than light penetration. Melting glaciers in the Arctic due to global warming releases turbid, fresh-melt waters, and inorganic material into the water column. In a study by Ronowicz et al. (2018), this had no effect on Arctic kelps (including Alaria esculenta and Laminaria digitata), but it did significantly affect the composition of faunal communities associated with the holdfast of the kelp. Species richness remained similar across sites and levels of disturbance, but the dominant taxa were different. In the lowest impacted sites, kelp holdfast communities were dominated by Hydrozoa, while the highest impacted sites were dominated by Bryozoa. Ronowicz et al. (2022) investigated Alaria esculenta morphological differences between 5 and 10 m depth at sites of varying levels of glacial influence. At the site with the most glacial influence (frequent iceberg scour and the highest load of suspended sediment), Alaria esculenta plants were significantly shorter, had reduced biomass, and had less morphological variability within the population. The authors observed no significant difference in these metrics between the non-impacted and intermediate-impacted (high sediment input alone) sites, suggesting that ice scour was the cause of the reduced size of Alaria esculenta at the highest-impacted site. Interestingly, the intermediate-impacted site had the greatest overall blade length and biomass values across the three levels of impact. Moreover, these metrics were greater at 10 m depth than at 5 m. While the levels of suspended sediment were not quantified, these morphological adaptations could serve as indirect evidence of resistance to suspended sediments and a reduction of light availability. Mytilus edulisMytilus edulis is often found in areas with high levels of turbidity. For example, the average suspended particulate matter (SPM) concentration at Hastings Shingle Bank was 15 to 20 mg/l in June 2005, reaching 50 mg/l in windier (force 4) conditions, although a concentration of 200 mg/l was recorded at this site during gales (Last et al., 2011). Winter (1972, cited by Moore, 1977) recorded 75% mortality of Mytilus edulis in concentrations of 1.84 to 7.36 mg/l when food was also available. However, a relatively small increase in SPM concentration e.g. from 10 mg/l to 90 mg/l was found to increase growth rates (Hawkins et al., 1996). Concentrations above 250 mg/l have been shown to impair the growth of filter-feeding organisms (Essink, 1999). But Purchon (1937) found that concentrations of particulates as high a 440 mg/l did not affect Mytilus edulis and that mortality only occurred when mud was added to the experiment bringing the concentrations up to 1220 mg/l. The reason for some of the discrepancy between studies may be due to the volume of water used in the experiment. Loosanoff (1962) found that in small quantities of turbid water (due to particulates) the mussel can filter out all of the particulates within a few minutes whereas in volumes >50 gallons per individual the mussel becomes exhausted before the turbidity has been significantly lowered, causing it to close its shell and die. Based on a comprehensive literature review, Moore (1977) concluded that Mytilus edulis displayed a higher tolerance to high SPM concentrations than many other bivalves although the upper limit of this tolerance was not certain. He also hypothesised that the ability of the mussel to clean its shell in such conditions played a vital role in its success along with its pseudofaecal expulsion. Recent evidence further supports the importance of suspended particulate material as a food resource. Field and experimental studies show that detrital and particulate organic matter can constitute a substantial proportion of the diet of Mytilus edulis, contributing at least 16% of ingested material (Both et al., 2020), and in estuarine systems more than 50% of annual food intake (Jung et al., 2019). Growth responses are often positive. In Australia, mussel size and dry mass increased with increasing particulate organic matter concentrations, particularly in shallow environments where detritus availability was high (Bearham et al., 2020). It may be possible for Mytilus edulis to adapt to a permanent increase in SPM by decreasing their gill size and increasing their palp size in areas of high turbidity (Theisen, 1982; Essink, 1999). In areas of variable SPM, it is likely that the gill size would remain the same but the palp would adapt (Essink, 1999). In addition to morphological adjustment, feeding performance itself appears to be flexible. Steeves et al. (2020) demonstrated that capture efficiency, pumping rate and overall ingestion in Mytilus edulis varied both within and between populations along a fjord gradient (reflecting changes in suspended matter and water clarity). Reciprocal transplant experiments showed that these traits can adjust in response to local environmental conditions, indicating short- to medium-term physiological plasticity rather than fixed population-level differences. Whilst the ability to adapt may prevent immediate declines in health, the energetic costs of these adaptations may result in reduced fitness; the extent of which is still to be established. Mytilus edulis uses the circadian clock to determine the opening of the shell gape in nocturnal gape cycles (Ameyaw-Akumfi & Naylor, 1987). Last et al. (2011) investigated the effects on increased SPM concentrations on both the gape pattern and mortality in order to establish the effect that aggregate dredging will have on Mytilus edulis and other benthic invertebrates. Therefore, they tested concentrations similar to those expected within a few hundred meters of an aggregate extraction site. The highest concentration tested using a pVORT (paddle Vortex Resuspension Tanks) was approx. 71 mg/l. They reported a significant reduction of the strength of the nocturnal gape cycle at high suspended sediment loads as well as a change in the gape period. The effects of these changes are not fully known but as it is likely that the gape pattern is a strategy to avoid diurnal predators the change may result in an increased risk of predation. On the other hand, the increased turbidity may reduce predation by visual predators such as fish and birds (Essink, 1999). After continued measurements of the gape cycle for four days post-treatment, Last et al. (2011) observed that the cycle took longer than this to recover from the cycle disruption. Further study is required to determine the length of time required for recovery of this behavioural response (Last et al., 2011). Importantly, suspended material associated with turbidity is not inherently detrimental and often represents a significant energetic subsidy. Across a range of coastal and estuarine systems, particulate organic matter supports growth and condition rather than causing energetic limitation (Bearham et al., 2020; Both et al., 2020; Jung et al., 2019). As such, short-term behavioural disruption under elevated suspended sediment loads does not necessarily translate into reduced growth or population-level impacts. Mytilus edulis may be more sensitive to decreased turbidity where this reflects a decrease in the availability of organic matter and seston. Winter (1972) (cited by Moore, 1977) recorded 75% mortality of Mytilus edulis in concentrations of 1.84 to 7.36 mg/l when food was also available. However, a relatively small increase in SPM concentration e.g. from 10 mg/l to 90 mg/l was found to increase growth rates (Hawkins et al., 1996). Sensitivity AssessmentAn increase in water clarity from clear to intermediate (10 to 100 mg/l) represents a change in light attenuation of approx. 0.67 to 6.7 Kd/m and could result in a significant reduction in photosynthesis of kelps. Therefore, the dominant kelp species may suffer a significant decline and resistance to this pressure is assessed as ‘Low’ as a precaution. Resilience is ‘High’, so sensitivity is ‘Low’. | LowHelp | HighHelp | LowHelp |
Smothering and siltation rate changes (light) [Show more]Smothering and siltation rate changes (light)Benchmark. ‘Light’ deposition of up to 5 cm of fine material added to the seabed in a single discrete event (Smothering pressure definition). EvidenceAlaria esculenta is not found in areas of siltation and sediment scour (Birkett et al. 1998). Increased siltation and sediment scour inhibits photosynthesis and algal growth, interfere with spore or larval recruitment plus smother germlings and gametophytes (Fletcher 1996). However, the high degree of wave exposure that defines this biotope is likely to clear suspended sediments relatively quickly. If low water clarity is persistent and wave exposure decreased, then low energy silted kelp biotopes (IR.LIR.K) may proliferate. Once siltation returns to its pre-effect level the biotope is likely to recover its canopy within a year and the rest of the community in no more than five years. Increased siltation will also increase turbidity. Increased sediment may benefit Mytilus edulis and its abundance may increase in IR.HIR.KFaR.Ala.Myt although large individuals are likely to be removed by wave action. Melting glaciers in the Arctic due to global warming releases turbid, fresh-melt waters and inorganic material into the water column. In a study by Ronowicz et al. (2018), this had no effect on Arctic kelps (including Alaria esculenta and Laminaria digitata), but it did significantly affect the composition of faunal communities associated with the holdfast of the kelp. Species richness remained similar across sites and levels of disturbance, but the dominant taxa were different. In the lowest impacted sites, kelp holdfast communities were dominated by Hydrozoa, while the highest impacted sites were dominated by Bryozoa. Sedimentation has additional negative effects on the zoospores of brown algae, with spores attaching to the only substratum available. Hence, fine sediment could interfere with recruitment, by preventing and deterring spores attachment to a hard substratum; resulting in their subsequent loss due to waves and currents (Devinny & Volse, 1978, Norton, 1978; Bartsch et al., 2008). Field observations reveal that kelp is associated with accelerating sediment deposition and additionally prevent sediments being washed away because of their influence on local water current by increasing drag and thus particulate fall out (Airoldi, 2003 and references therein). However, this sediment is associated with the holdfasts of the kelp and not the fronds. At higher levels of wave exposure, whiplash by kelp is common, and this, in turn, reduces sediment accumulation at these sites (Kennelly 1989; Melville & Connell, 2001; cited in Airoldi, 2003). Alaria esculentaPicard et al. (2022) investigated the effects of different levels of sediment loading on Alaria esculenta zoospores in petri dishes. They placed seawater with different concentrations of sediment into the dishes: 0g (control), 1.5 and 2.5g of sediment in 50 ml seawater, which corresponded to approx. 0, 75, and 100% sediment coverage of the dish surface. The authors stated that the highest sediment level provided 100% cover of the dishes in a single-grain layer, therefore it was estimated that the sediment layer depth was 63 to 125 μm. Dishes were maintained in gently moving seawater and were kept in darkness (to exclude turbidity effects) for 89 hours. At the end of the experiment, attached spore density, gametophyte density, and the proportion of attached spores that had germinated (development ratio) were measured. While sediment levels had an insignificant effect on attached spore density and gametophyte density, the latter still saw a decrease from 14 gametophytes/mm2 in the no sediment treatment to 10 gametophytes/mm2 in the maximum sediment treatment. However, spore development ratio did significantly decline with sediment loading (from 38 to 24% between the no sediment and maximum sediment treatments, respectively). In summary, this study showed that a sediment layer of 63 to 125 μm was enough to significantly reduce the development of gametophytes, and that the impacts of sediment on Alaria esculenta recruitment success occurs after the settlement stage (Picard et al., 2022). Zacher et al. (2016) investigated the combined effects of warming, grazing, and sedimentation on early life stages of Alaria esculenta. In their full factorial experiment, they tested temperatures of 5 and 9°C with and without the grazing gastropod Margarites helicinus, and three levels of sedimentation (no sediment, 1 g, and 10 g per petri dish). They measured the proportion of germinated spores after five days and counted the density of juvenile sporophytes after 14 days. The authors observed a statistically significant interaction between temperature and grazing, but no interaction was observed between sedimentation and the other variables. By itself, however, sedimentation had a significant negative effect on germination. In the 5°C grazed treatment, germination was the same between no sediment and 1g sediment, but it was significantly lower with 10g sediment. The 9°C treatment showed similar patterns with and without grazers as the 5°C ungrazed treatment, where germination declined with increasing levels of sedimentation, but the decline was less pronounced in the 9°C treatments. Sedimentation also negatively affected the density of sporophytes across all temperature and grazing levels. Sporophyte density was zero in all 10g sediment treatments apart from in the grazed treatments. Mytilus edulisMytilus edulis occurs in areas of high suspended particulate matter (SPM) and therefore a level of siltation is expected from the settling of SPM. In addition, the high rate of faecal and pseudofaecal matter production by the mussels naturally results in siltation of the seabed, often resulting in the formation of large mounds beneath the mussel bed. For example, at Morecambe Bay, an accumulation of mussel-mud (faeces, pseudofaeces and washed sand) of 0.4 to 0.5m between May 1968 and September 1971 resulted in the mortality of young mussels (Daly & Mathieson, 1977). In order to survive the mussels needed to keep moving upwards to stay on the surface. Many individuals did not make it to the surface and were smothered by the accumulation of mussel-mud (Daly & Mathieson, 1977), so that whilst Mytilus edulis does have the capacity to vertically migrate through sediment some individuals will not survive. Sand burial has been shown to determine the lower limit of Mytilus edulis beds (Daly & Mathieson, 1977). Burial of Mytilus edulis beds by large scale movements of sand, and resultant mortalities have been reported from Morecambe Bay, the Cumbrian coast and Solway Firth (Holt et al., 1998). Essink (1999) recorded fatal burial depths of 1 to 2 cm for Mytilus edulis and suggested that they had a low tolerance of sedimentation based on investigations by R.Bijkerk (cited by Essink, 1999). Essink (1999) suggested that deposition of sediment (mud or sand) on shallow mussel beds should be avoided. However, Widdows et al. (2002) noted that mussels buried by 6 cm of sandy sediment (caused by resuspension of sediment due to turbulent flow across the bed) were able to move to the surface within one day. Conversely, Condie (2009) (cited by Last et al., 2011) reported that Mytilus edulis was tolerant of repeated burial events. Experimental evidence supports the conclusion that burial to depths relevant to the light smothering benchmark can be tolerated for short periods, but that mortality increases with burial duration, sediment fineness and temperature. Last et al. (2011; reported in Hutchison et al.,2016) exposed Mytilus edulis to sudden burial at depths of 2, 5 and 7 cm using coarse, medium and fine sediments for up to 32 days. Overall mortality across all treatments was relatively low (13%), but increased strongly with duration (from 4% after two days to 44% after 32 days) and was substantially higher in fine sediments (28%) than in coarse sediments (2%), reflecting reduced emergence success (Last et al., 2011; Hutchison et al., 2016). Only 16% of buried mussels died after 16 days compared to almost 50% mortality at 32 days. Mortality also increased sharply with a decrease in particle size and with increases in temperature from 8.0 and 14.5 to 20°C. The ability of a proportion of individuals to emerge from burial was again demonstrated with approx. one quarter of the individuals buried at 2 cm resurfacing. However, at depths of 5 cm and 7 cm no emergence was recorded (Last et al., 2011). The lower mortality when buried in coarse sands may be related to the greater number of individuals who were able to emerge in these conditions and emergence was to be significant for survival (Last et al., 2011). The capacity for vertical migration through accumulating sediment has also been demonstrated under gradual burial scenarios. Hutchison et al. (2020) showed that mussels were able to migrate upwards through coarse, medium and fine sediments deposited at rates of 0.5 to 1.5 cm per day over periods of up to 16 days. However, the proportion of buried individuals increased with both burial rate and duration, with approx. 30% buried at 0.5 cm/day and nearly 95% buried at 1.5 cm/day after 16 days, indicating that sustained or rapid sedimentation can overwhelm this compensatory response. It is unclear whether the same results would be recorded when mussels are joined by byssal threads or whether this would have an impact on survival (Last et al., 2011), although Daly & Mathieson (1977) recorded loose attachments between juvenile mussels during a burial event and some of these were able to surface. It was not clear whether the same ability would be shown by adult mussels in a more densely packed bed. Burial-associated mortality is further influenced by the organic content of the smothering material. Cottrell et al. (2016) demonstrated significantly higher mortality of Mytilus edulis under 5 cm burial when sediments contained elevated organic matter, particularly in fine sediments. Mortality increased rapidly within two days and rose with both organic content and temperature, reaching over 50% in fine sediments with 1% organic matter under summer temperature conditions (20°C). The authors suggested that enhanced microbial activity and pathogenic processes within organically enriched sediments contributed to mortality, particularly under low-oxygen conditions. Sensitivity AssessmentWhile the evidence shows that ‘light’ deposition of up to 5 cm of sediment (as per the pressure benchmark) could have a severe impact on Alaria esculenta, the high degree of wave exposure that typically defines this biotope is likely to clear 5 cm of deposited sediment quickly (within one tidal cycle). If low water clarity is persistent and wave exposure decreased, then low energy silted kelp biotopes (IR.LIR.K) may proliferate. Increased sediment may benefit Mytilus edulis and its abundance may increase although large individuals are likely to be removed by wave action. Therefore, resistance is assessed as ‘High’, resilience as ‘High’ and the biotope is probably ‘Not Sensitive’ at the benchmark level. | HighHelp | HighHelp | Not sensitiveHelp |
Smothering and siltation rate changes (heavy) [Show more]Smothering and siltation rate changes (heavy)Benchmark. ‘Heavy’ deposition of up to 30 cm of fine material added to the seabed in a single discrete event (Smothering pressure definition). EvidenceAlaria esculenta is not found in areas of siltation and sediment scour (Birkett et al., 1998). Increased siltation and sediment scour inhibits photosynthesis and algal growth, interfere with spore or larval recruitment plus smother germlings and gametophytes (Fletcher 1996). However, the high degree of wave exposure that defines this biotope is likely to clear suspended sediments relatively quickly. If low water clarity is persistent and wave exposure decreased, then low energy silted kelp biotopes (IR.LIR.K) may proliferate. Once siltation returns to its pre-effect level the biotope is likely to recover its canopy within a year and the rest of the community in no more than five years. Increased siltation will also increase turbidity. Increased sediment may benefit Mytilus edulis and its abundance may increase in IR.HIR.KFaR.Ala.Myt although large individuals are likely to be removed by wave action. Melting glaciers in the Arctic due to global warming release turbid, fresh-melt waters and inorganic material into the water column. In a study by Ronowicz et al. (2018), this had no effect on arctic kelps (including Laminaria digitata), but it did significantly affect the composition of faunal communities associated with the holdfast of the kelp. Species richness remained similar across sites and levels of disturbance, but the dominant taxa were different. In the lowest impacted sites, kelp holdfast communities were dominated by Hydrozoa, while the highest impacted sites were dominated by Bryozoa. Sedimentation has additional negative effects on the zoospores of brown algae, with spores attaching to the only substratum available. Hence, fine sediment could interfere with recruitment, by preventing and deterring spores attachment to a hard substratum; resulting in their subsequent loss due to waves and currents (Devinny & Volse, 1978, Norton, 1978; Bartsch et al., 2008). Field observations reveal that kelp is associated with accelerating sediment deposition and additionally prevent sediments being washed away because of their influence on local water current by increasing drag and thus particulate fall out (Airoldi, 2003 and references therein). However, this sediment is associated with the holdfasts of the kelp and not the fronds. At higher levels of wave exposure, whiplash by kelp is common, and this, in turn, reduces sediment accumulation at these sites (Kennelly 1989; Melville & Connell, 2001; cited in Airoldi, 2003). Mytilus edulisMytilus edulis occurs in areas of high suspended particulate matter (SPM) and therefore a level of siltation is expected from the settling of SPM. In addition, the high rate of faecal and pseudofaecal matter production by the mussels naturally results in siltation of the seabed, often resulting in the formation of large mounds beneath the mussel bed. For example, at Morecambe Bay, an accumulation of mussel-mud (faeces, pseudofaeces and washed sand) of 0.4 to 0.5 m between May 1968 and September 1971 resulted in the mortality of young mussels (Daly & Mathieson, 1977). In order to survive the mussels needed to keep moving upwards to stay on the surface. Many individuals did not make it to the surface and were smothered by the accumulation of mussel-mud (Daly & Mathieson, 1977), so that whilst Mytilus edulis does have the capacity to vertically migrate through sediment some individuals will not survive. Experimental evidence supports the conclusion that burial to depths relevant to the light smothering benchmark can be tolerated for short periods, but that mortality increases with burial duration, sediment fineness and temperature. Last et al. (2011) exposed Mytilus edulis to sudden burial at depths of 2, 5 and 7 cm using coarse, medium and fine sediments for up to 32 days. Overall mortality across all treatments was relatively low (13%), but increased strongly with duration (from 4% after two days to 44% after 32 days) and was substantially higher in fine sediments (28%) than in coarse sediments (2%), reflecting reduced emergence success. Only 16% of buried mussels died after 16 days compared to almost 50% mortality at 32 days. Mortality also increased sharply with a decrease in particle size and with increases in temperature from 8.0 and 14.5 to 20°C. The ability of a proportion of individuals to emerge from burial was again demonstrated with approx. one quarter of the individuals buried at 2 cm resurfacing. However, at depths of 5 cm and 7 cm no emergence was recorded. The lower mortality when buried in coarse sands may be related to the greater number of individuals who were able to emerge in these conditions and emergence was to be significant for survival (Last et al., 2011). The capacity for vertical migration through accumulating sediment has also been demonstrated under gradual burial scenarios. Hutchison et al. (2020) showed that mussels were able to migrate upwards through coarse, medium and fine sediments deposited at rates of 0.5 to 1.5 cm per day over periods of up to 16 days. However, the proportion of buried individuals increased with both burial rate and duration, with approx. 30% buried at 0.5 cm/day and nearly 95% buried at 1.5 cm/day after 16 days, indicating that sustained or rapid sedimentation can overwhelm this compensatory response. It is unclear whether the same results would be recorded when mussels are joined by byssal threads or whether this would have an impact on survival (Last et al., 2011), although Daly & Mathieson (1977) recorded loose attachments between juvenile mussels during a burial event and some of these were able to surface. It was not clear whether the same ability would be shown by adult mussels in a more densely packed bed. Burial-associated mortality is further influenced by the organic content of the smothering material. Cottrell et al. (2016) demonstrated significantly higher mortality of Mytilus edulis under 5 cm burial when sediments contained elevated organic matter, particularly in fine sediments. Mortality increased rapidly within two days and rose with both organic content and temperature, reaching over 50% in fine sediments with 1% organic matter under summer temperature conditions (20°C). The authors suggested that enhanced microbial activity and pathogenic processes within organically enriched sediments contributed to mortality, particularly under low-oxygen conditions. Sensitivity AssessmentWhile the evidence shows that ‘heavy’ deposition of up to 30 cm of sediment (as per the pressure benchmark) could have a severe impact on Alaria esculenta, the high degree of wave exposure that typically defines this biotope is likely to clear the deposited sediment quickly (within one tidal cycle). If low water clarity is persistent and wave exposure decreased, then low energy silted kelp biotopes (IR.LIR.K) may proliferate. Increased sediment may benefit Mytilus edulis and its abundance may increase although large individuals are likely to be removed by wave action. Therefore, resistance is assessed as ‘High’, resilience as ‘High’ and the biotope is probably ‘Not Sensitive’ at the benchmark level. | HighHelp | HighHelp | Not sensitiveHelp |
Litter [Show more]LitterBenchmark. The introduction of man-made objects able to cause physical harm (surface, water column, seafloor or strandline) (Litter pressure definition). EvidenceNot assessed. | Not Assessed (NA)Help | Not assessed (NA)Help | Not assessed (NA)Help |
Electromagnetic changes [Show more]Electromagnetic changesBenchmark. A local electric field of 1 V/m or a local magnetic field of 10 µT (Electromagnetic pressure definition). EvidenceEvidence on the effect of electromagnetic fields (EMFs) on benthic organisms is still severely lacking. There have been no studies examining the effect of EMFs on macroalgae. Some studies have investigated the effect of anthropogenically induced EMFs on benthic invertebrates at intensities ranging between 2 nT and 40 mT, which is often much higher than in situ measurements from subsea cables. While some report changes to behaviour, physiology, reproduction, development, immunology, cytotoxicity, and orientation, others demonstrate no effect from exposure to the EMF (Albert et al., 2020; Hutchison et al., 2020), depending on the study species and duration and intensity of exposure. Albert et al. (2022) experimentally investigated the effects of magnetic fields comparable to those generated by buried subsea power cables on adult Mytilus edulis. Mussels were exposed to a direct current magnetic field of 300 µT, substantially above the ambient geomagnetic field (approx. 47 µT), reflecting field strengths measured in close proximity to power cables. No significant differences were observed in valve gaping behaviour or filtration rates between exposed and control individuals, indicating no detectable impairment of feeding behaviour under the conditions tested. Sensitivity AssessmentGiven the lack of data at the level of individual biotopes, resistance and resilience to EMFs cannot be robustly assessed. Sensitivity is therefore recorded as ‘Insufficient Evidence’. | Insufficient evidence (IEv)Help | Insufficient evidence (IEv)Help | Help |
Underwater noise changes [Show more]Underwater noise changesBenchmark. MSFD indicator levels (SEL or peak SPL) exceeded for 20% of days in a calendar year. Further detail EvidenceMytilus edulis are sessile as adults but have planktonic larvae and post-larval stages that are potentially more sensitive to environmental stressors, including anthropogenic underwater noise. Evidence indicates that both behavioural and physiological responses can be elicited by exposure to noise across a range of frequencies, intensities, and durations. Studies on larval and early life stages show that exposure to vessel noise at environmentally relevant levels can induce physiological and behavioural effects. Jolivet et al. (2016) reported that low-frequency vessel noise (127 ± 3 dB re 1 µPa between 100 and 1,000 Hz) interacted with food availability to significantly increase larval settlement, while Veillard, Beauclercq, Ghafari et al. (2025) and Veillard, Beauclercq, Palacios et al. (2025) demonstrated that shipping noise during embryogenesis and early post-larval development provoked stress-related metabolic disruption, delayed metamorphosis, and altered energy pathways, potentially reducing larval fitness and affecting subsequent recruitment. In contrast, Aspirault et al. (2023) found no impact on larval feeding behaviour at similar noise levels, while Haque & Kwon (2018) reported near-total larval mortality only under specialized high-frequency ultrasound treatments used for antifouling, which are unlikely to occur under typical shipping conditions. Adult Mytilus edulis respond to underwater noise through partial valve closure, changes in clearance rates, and sublethal oxidative and DNA damage (Hubert et al., 2022; Roberts et al., 2015; Spiga et al., 2016; Wale et al., 2019), although behavioural responses often decay over repeated exposures, indicating some capacity for habituation. Continuous low-frequency noise did not impair byssal thread production in adults (Wang et al., 2024), which may partly explain their persistence in noisy environments. Noise exposure has also been associated with suppression of immune function in adults when combined with bacterial challenge, although no direct mortality was observed (Chapuis et al., 2025). Overall, these studies indicate that underwater noise is unlikely to cause widespread mortality in adult mussels but can induce sublethal physiological stress, behavioural modifications, and, for early life stages, potential delays in development that may influence recruitment success. Sensitivity AssessmentBased on the available evidence, adult Mytilus edulis show a high tolerance to typical underwater noise at the benchmark level, with no significant mortality or reduction in population viability. Sub-lethal effects, including valve closure, altered clearance rates, oxidative stress, and immune modulation, have been observed, but these do not appear to threaten overall population persistence. Larval and post-larval stages may experience developmental delays, metabolic stress, or altered settlement patterns when exposed to sustained or high-intensity noise, which could influence recruitment. However, these effects are unlikely to result in population-level declines under the benchmark exposure, and subsequent reproductive cycles may compensate for temporary recruitment reductions. Resistance and resilience of this biotope is ‘High’, and sensitivity is therefore assessed as ‘Not Sensitive’. | HighHelp | HighHelp | Not sensitiveHelp |
Introduction of light or shading [Show more]Introduction of light or shadingBenchmark. A change in incident light via anthropogenic means (Introduced light or shade pressure definition). EvidenceIt is feasible that localised light sources (e.g. post or harbour side lighting) might increase the length of time available for photosynthesis in shallow examples of the biotope that are in the vicinity. The effects of artificial light on kelp are not yet fully understood, but there is now a growing body of evidence to show that artificial light at night (ALAN) is widespread in the marine environment, with biologically relevant levels of light penetrating to depths of up to 50m (Davies et al., 2020; Smyth et al., 2021). ALAN has been shown to change the timing of Ascophyllum nodosum and Fucus serratus reproduction, with receptacles (the reproductive tissues of fucoid macroalgae) continuing to ripen into the winter months instead of peaking in the summer (Moyse et al., 2025). This change in the timing of reproduction could result in gametes being released during suboptimal conditions, such as winter storms, and therefore reduce fertilisation success. Reduced recruitment may lead to shifts in macroalgal assemblages in favour of species which are less sensitive to ALAN, such as Fucus vesiculosus, which seems to be unaffected (Moyse et al., 2025). ALAN can also vary significantly on small spatial scales and therefore affect some macroalgal forests more than others even if they are close to one another. It is therefore possible that ALAN could cause changes in macroalgal assemblages over time. Shading of the biotope (e.g. by coastal development) could adversely affect the biotope in areas already low in water clarity. This may lead to a decline in Alaria esculenta abundance in shaded areas and a shift in dominance towards shade-tolerant red algae or faunal turfs. Staehr & Wernberg (2009) showed that, across typical coastal water clarity, an increase in the diffuse light attenuation coefficient KD from 0.1 /m to 0.2 /m (representing a shift from clear to slightly more turbid water) can reduce the depth limit of the kelp Ecklonia radiata by around 50%. Alaria esculentaAlaria esculenta gametophytes cultured from sporophytes originating from Spitsbergen, Norway, showed no significant growth and no gametogenesis under natural winter conditions (2°C in complete darkness for 60 days) (Silva et al., 2022). In the first 38 days, gametophyte density decreased by 42%, suggesting a strong lack of resistance to darkness, but density did not continue to decrease for the remaining 22 days of darkness, indicating that gametophyte density was sensitive to darkness only to an extent. Gametophytes did not become fertile after returning to spring conditions (5°C a 12:12-hour light:dark regime for 36 days), suggesting that sporogenesis, reproduction and recruitment must occur during summer or autumn. In their full factorial experiment, Silva et al. (2022) also tested the combined effects of light intensity, temperature, and nutrient availability on Alaria esculenta gametophytes. The experiment crossed three irradiance levels (0.5, 35 and 100 μmol photons m²/s), two temperatures (5°C control and 9°C future-warming treatment), and two nutrient regimes: low nutrients (2 μM N and 0.2 μM P) and an unspecified high-nutrient treatment simulating increased inputs from mixing, river discharge, and permafrost melt. At 5°C under low nutrient conditions, gametophyte density decreased significantly with increasing irradiance. In contrast, at 9°C under low nutrient conditions, densities were similar under low and medium light levels, and higher under high light than at 5°C. Under high nutrient conditions, densities were generally lower overall, but high irradiance still resulted in reduced gametophyte density, particularly at 9°C. These findings indicate that the effects of irradiance may depend on temperature and nutrient availability. Gordillo et al. (2022) observed an approximate 50% loss of Alaria esculenta biomass at 8°C, which was 21% more than the biomass loss of those at 3°C, in an experiment simulating the arctic winter. Towards the end of the dark period, Alaria esculenta produced new blade tissue in the 3°C treatment which continued to grow for two months after light returned. However, in the 8°C treatment, only the holdfast and midrib were left, and growth was unable to resume, so further measurements were not possible. Physiological responses to prolonged darkness included declines in respiration and photosynthetic performance (both of which were more pronounced with warming), chlorophyll-a, and carbon content. Nitrogen content remained unaffected. Similarly, Cobos et al. (2026) simulated a transition out of polar night, where kelps spend two months in total darkness, followed by increasing light exposure. In both 1°C and 5°C treatments, biomass fell to 70 to 80% of the starting fresh weight, while respiration photosynthetic parameters, and pigment concentrations declined similarly. However, the loss of nitrogen in 5°C was double that of the 1°C treatment, while the loss of nitrate reserves was much lower. In addition, carbon content decreased slightly instead of increasing. In the 2-week light period following the dark period, Alaria esculenta growth resumed in both treatments, more so in the cold treatment. The 1°C treatment saw rapid photosynthetic reactivation, positive carbon balance, and a strong growth recovery, while the warming scenario resulted in higher respiration costs, greater nitrogen depletion, loss of photosynthetically active tissue, and a much lower growth recovery. This shows that warming can have a strong negative effect on Alaria esculenta even in colder regions, and this effect can persist even after light levels return to normal. This indicates that recovery after periods of darkness may be rapid under colder conditions and more constrained when darkness is combined with elevated temperature. Ronowicz et al. (2022) found morphological differences between Alaria esculenta plants at 5 and 10 m depth at sites of varying levels of glacial influence. At the site with the most glacial influence (frequent iceberg scour and the highest load of suspended sediment), Alaria esculenta plants were significantly shorter, had reduced biomass, and had less morphological variability within the population. The authors observed no significant difference in these metrics between the non-impacted and intermediate-impacted (high sediment input alone) sites, suggesting that ice scour was the cause of the reduced size of Alaria esculenta at the highest-impacted site. Interestingly, the intermediate-impacted site had the greatest overall blade length and biomass values across the three levels of impact. Moreover, these metrics were greater at 10 m depth than at 5 m. While the levels of suspended sediment were not quantified, these morphological adaptations could serve as indirect evidence of resistance to suspended sediments and a reduction of light availability. The development of Alaria esculenta gametophytes into sporophytes can also vary with the amount of light they receive during the gametophyte stage. Martins et al. (2022) showed that gametophyte growth increased with increasing daylength to a limit. While continuous light with no dark period resulted in faster growth, it also produced abnormal recruits with irregular form and reduced pigmentation. They also found that the direction of photoperiod effects on Alaria esculenta changed with life stage. Sporophytes that developed from the gametophytes under the increased daylengths grew slower than those that were cultured under the reduced daylengths. In addition, temperature was found to have an interactive effect with light. Elevated temperatures reduced growth, therefore exacerbating the effects of suboptimal light regimes experienced during the gametophyte stage. Laeseke et al. (2019) investigated whether Alaria esculenta canopies protect kelp spores from harmful solar radiation in Kongsfjorden, Norway. They measured underwater light at 3 m depth beneath different canopy densities (very dense, dense, intermediate, sparse, and no canopy) and then used these measurements for realistic laboratory simulations. Alaria esculenta zoospores were then exposed to each light regime for 4, 8, 16, or 24 hours at ambient seawater temperature (4°C). Germination remained largely unaffected, so it was concluded that natural radiation conditions in Kongsfjorden are unlikely to severely reduce recruitment, despite some physiological parameters being affected. UV exposure can have an interactive effect with increased CO2 levels in the water column. Gordillo et al. (2015) investigated the combined effects of UV radiation and ocean acidification on Alaria esculenta from Kongsfjorden. The experiment consisted of two levels of light and acidification which were fully crossed: PAR at 30 μmol m²/s with no UV, and PAR with UV supplementation (2 W/m² UVA and 0.2 W/m² UVB); ambient CO2 (pH 8.1 to 8.3) and high elevated CO2 (pH 7.7 to 7.8). Alaria esculenta growth rate increased by 57% in the UV-enriched + elevated CO2 treatment, while the UV-enriched alone and the elevated CO2 alone reduced growth compared to the no-UV + low-CO2 treatment, therefore indicating a synergistic effect. Photosynthetic efficiency was not affected in the low-CO2 treatments, while the high-CO2 treatments saw a significant decline after two days, most notably in the UV-enriched + elevated CO2 treatment, indicating stress. However, after six days of exposure, photosynthetic efficiency recovered almost to pre-exposure levels. Pigment concentrations (chlorophyll-a and carotenoids) declined under all treatments, but losses were greatest under elevated CO₂ alone and were moderated in UV-exposed treatments. Internal carbon content increased under both elevated CO₂ and UV exposure, while nitrogen content and nitrate reductase activity were largely unaffected by treatment. Overall, increases in UV or CO₂ alone cause physiological stress in Alaria esculenta, but when they are combined, they are beneficial. Lebrun et al. (2024) investigated the combined effects of warming, salinity, and light on four kelp species, including Alaria esculenta. For six weeks, kelps collected from Kongsfjorden, were exposed to an unmanipulated control treatment which had ambient seawater flowing into the tank at roughly 5.3°C, 33.8 PSU, with an irradiance of 47.8 µmol photons/m2/s, and three additional treatments: T1 = moderate warming (+3.3°C), reduced salinity (-2.5 PSU, and reduced light (-25% irradiance); T2 = stronger warming (+5.3°C), greater salinity reduction (-5 PSU), and lower light (-40% irradiance); and T3 = stronger warming alone (+5.3°C) without changes in salinity or irradiance. These conditions were chosen to reflect future global warming scenarios in which warming increases ice-melt, causing an addition of freshwater and suspended sediments and particles into the marine environment. Chlorophyll-a concentration declined in the control, reflecting normal seasonal changes, and showed similar patterns in T1 and T3. However, chlorophyll-a remained significantly higher in T2 (stronger warming with reduced salinity and light). Growth rates and carbon:nitrogen ratios were stable across the experiment. These results suggest that Alaria esculenta could potentially be resistant to the combined effects of global warming, reduced salinity, and reduced light. Mytilus edulisMytilus edulis exhibits light-sensitive behavioural and developmental responses, although the long-term population-level consequences remain unclear. Laboratory studies using artificial light at night (ALAN) show that red and white light (at 20 lux ± 0.5, approx. equivalent to average street ALAN and coastal water surface levels) reduces valve gaping frequency, potentially decreasing feeding activity, whereas green light at the same intensity increases gaping frequency, which may be energetically costly and elevate predation risk (Christoforou et al., 2023). In early life stages, ALAN exposure has been associated with significant reductions in larval survival, with up to 57% mortality after 60 days of continuous exposure at 50 lux, suggesting that prolonged light exposure can impair recruitment (Tidau et al., 2023). Behavioural rhythms in Mytilus spp. are strongly influenced by photoperiod. Tran et al. (2020) monitored a recently re-established population of Mytilus sp. in the high Arctic over nearly two years and found that shell growth and valve activity followed a clear annual rhythm, with much higher rates during the polar day compared to the polar night. This rhythmicity was closely tied to the light-dark cycle rather than water temperature, indicating that the species’ behavioural and growth patterns are highly responsive to photoperiod. By contrast, a native bivalve, Chlamys islandica, showed no clear annual rhythm in valve behaviour or growth, emphasizing the particular sensitivity and adaptability of Mytilus to light cues. Tran et al. (2020) concluded that Mytilus sp. can adjust its physiology and behaviour to extreme and rapidly changing photoperiods, suggesting a capacity for resilience to alterations in incident light, although the energetic costs and implications for survival under chronic artificial illumination remain unknown. Sensitivity AssessmentAlaria esculenta has mixed responses to increases in light, for example due to increased solar radiation, reduced turbidity, the removal of coastal infrastructure, or artificial light sources. Changes in light regimes have also been shown to produce abnormal recruits with lower growth rates (Martins et al., 2022), while increased irradiance can reduce gametophyte density under elevated temperatures and nutrient concentrations (Silva et al., 2022). Elevated UV levels may additionally cause physiological stress (Gordillo et al., 2015). There is currently no evidence of Alaria esculenta’s response to artificial light at night (ALAN). Evidence from other macroalgae suggests that ALAN can alter reproductive timing and affect assemblage structure (Moyse et al., 2025). Regarding Mytilus edulis, Tidau et al. (2023) reported that ALAN significantly reduced larval survival in Mytilus edulis, and Christoforou et al. (2023) found that artificial lighting induced behavioural changes that increased energetic expenditure and potentially elevated predation risk. Therefore, the biotope’s resistance to an increase in light is assessed as ‘Medium’ as a precaution due to the effects of ALAN on the characterising species’ reproductive cycles, resilience as ‘High’ if the source of the light is removed quickly, but ‘Very Low’ if permanent. Therefore, in a worst-case scenario where an increase in light is permanent, sensitivity is assessed as ‘Medium’. Shading of the biotope would certainly negatively affect Alaria esculenta. The evidence shows that Alaria esculenta does not grow and cannot produce gametes in prolonged periods of darkness (Silva et al., 2022), whilst also experiencing declines in physiological performance and biomass, and that recovery from darkness can be constrained in higher temperatures (Gordillo et al., 2022; Cobos et al., 2026). Therefore, resistance to shading is ‘Low’ and resilience is ‘High’ if the source of the shading is removed quickly, but ‘Very Low’ if permanent. Therefore, in a worst-case scenario where shading is permanent, sensitivity to shading is assessed as ‘High’. | LowHelp | Very LowHelp | HighHelp |
Barrier to species movement [Show more]Barrier to species movementBenchmark. A permanent or temporary barrier to species movement over ≥50% of water body width or a 10% change in tidal excursion (Barrier to species movement pressure definition). EvidenceNot relevant. This pressure is considered applicable to mobile species, e.g. fish and marine mammals rather than seabed habitats. Physical and hydrographic barriers may limit the dispersal of spores. But spore dispersal is not considered under the pressure definition and benchmarks, e.g. fish and marine mammals rather than seabed habitats. Physical and hydrographic barriers may limit the dispersal of spores. But spore dispersal is not considered under the pressure definition and benchmark. | Not relevant (NR)Help | Not relevant (NR)Help | Not relevant (NR)Help |
Death or injury by collision [Show more]Death or injury by collisionBenchmark. Injury or mortality from collisions of biota with both static or moving structures due to 0.1% of tidal volume on an average tide, passing through an artificial structure (Death for collision pressure definition). EvidenceNot relevant. Collision from grounding vessels is addressed under abrasion above. | Not relevant (NR)Help | Not relevant (NR)Help | Not relevant (NR)Help |
Visual disturbance [Show more]Visual disturbanceBenchmark. The daily duration of transient visual cues exceeds 10% of the period of site occupancy by the feature (Visual disturbance pressure definition). EvidenceNot relevant | Not relevant (NR)Help | Not relevant (NR)Help | Not relevant (NR)Help |
Biological Pressures
Use [show more] / [show less] to open/close text displayed
| Resistance | Resilience | Sensitivity | |
Genetic modification & translocation of indigenous species [Show more]Genetic modification & translocation of indigenous speciesBenchmark. Translocation of indigenous species or the introduction of genetically modified or genetically different populations of indigenous species may result in changes in the genetic structure of local populations, hybridization, or a change in community structure (Translocation pressure definition). EvidenceNo evidence | No evidence (NEv)Help | Not relevant (NR)Help | No evidence (NEv)Help |
Introduction of microbial pathogens [Show more]Introduction of microbial pathogensBenchmark. The introduction of relevant microbial pathogens or metazoan disease vectors to an area where they are currently not present (e.g. Martelia refringens and Bonamia, Avian influenza virus, viral Haemorrhagic Septicaemia virus) (pathogen or disease pressure definition). EvidenceThere is no evidence in the literature that infection by microbial pathogens results in the mass death of kelp populations and the kelp themselves are known to regulate bacterial infections through iodine metabolism (Cosse et al., 2009). Laminariocolax aecidioides (syn. Streblonema aecidioides and Gononema aecidioides) is a filamentous brown alga that causes spot disease in kelps (Lein et al., 1991). Laminariocolax sp. (syn. Entonema, Streblonema, or Myrionema) has been found in Alaria esculenta, Laminaria digitata, and Saccharina latissima (studied as Laminaria saccharina) (Levring, 1937; Jaasund, 1965; Jorde, 1975; cited in Lein et al., 1991). The endophytic brown microalga Microspongium alariae has been described to “infect” the tissues of many kelp species including Alaria esculenta, sometimes causing the appearance of warts (Murúa et al., 2018). However, it is not currently known if this infection is detrimental to the host kelp. Microspongium alariae has been found in Alaria esculenta hosts in Scotland and in Brittany (France). Evidence for a new group of phaeoviruses (viruses which affect macroalgae) infecting kelps was first reported by McKeown et al. (2017). Within this group (sub-group C) is the type species referred to as LdigV, which targets the nucleus in the cells of Laminaria digitata for its genome replication. This infection results in the degradation of chloroplasts and the assembly of virions in the cytoplasm of vegetative and reproductive cells. McKeown et al. (2017) found that 64.7% of sporophytes and 23.2% of gametophyte mixes (both from all three kelp species sampled) tested positive for the phaeovirus. Infection of Laminaria japonica sporophytes by Pseudoalteromonas, Vibrio and Halomonas result in the characteristic symptoms of hole-rotten disease (Wang et al., 2008). Additionally, red spot disease may be caused by bacteria of the genus Alteromonas (Sawabe et al., 1998). Hyperplasia or gall growths are often seen as dark spots on Laminaria digitata and have been associated with endophytic brown filamentous algae. It can be inferred from these observations that microbial pathogens may impact growth rates of individuals. Evidence of fungal pathogens has been reported for Laminaria digitata. Kononenko et al. (2022) reported traces of mycotoxins (toxic compounds produced by fungi) such as ergot alkaloids (produced by Claviceps spp.) and aflatoxins (produced by Aspergillus spp.). However, no signs of infection were reported. As a species with commercial significance, more research effort has been expended on Mytilus edulis. Much of this sensitivity assessment will be based evidence from a recent review by Mainwaring et al. (2014) of the impacts of Marteilia refringens on Mytilus edulis populations. It should be noted that Mytilus edulis beds are host to a diverse array of disease organisms, parasites and commensals from many animal and plant groups including bacteria, blue-green algae, green algae, protozoa, boring sponges, boring polychaetes, boring lichen, the intermediary life stages of several trematodes, copepods and decapods (Bower, 1992; Gray et al., 1999; Bower, 2010). However, at usual levels of infestation, these are not considered to lead to high levels of mortality. Outbreaks of Bonamia may cause significant mortalities in some shellfish populations but this protozoan has been shown not to infect Mytilus edulis (Culloty et al., 1999). Marteilia refringens can infect and have significant impacts on the health of Mytilus edulis. There is some debate as to whether there are two species of Marteilia, one which infects oysters (Marteilia refringens) and another that infects blue mussels (Marteilia maurini) (Le Roux et al., 2001) or whether they are just two strains of the same species (Lopez-Flores et al.,2004; Balseiro et al., 2007). Both species are present in southern parts of the United Kingdom. The infection of Marteilia results in Marteiliosis which disrupts the digestive glands of Mytilus edulis especially at times of spore release. Heavy infection can result in a reduced uptake of food, reduced absorption efficiency, lower carbohydrate levels in the haemolymph and inhibited gonad development particularly after the spring spawning resulting in an overall reduced condition of the individual (Robledo et al., 1995). Recent evidence suggests that Marteilia is transferred to and from Mytilus edulis via the copepod Paracartia grani. This copepod is not currently prevalent in the UK waters, with only a few records in the English Channel and along the South coast. However, it is thought to be transferred by ballast water and so localised introductions of this vector may be possible in areas of mussel seed transfer. The mussel populations here are considered to be naive (i.e. not previously exposed) and therefore could be heavily affected, although the likelihood is slim due to the dependence on the introduction of a vector that is carrying Marteilia and then it being transferred to the mussels. Experimental infection of Mytilus edulis with Marteilia pararefringens in Norway induced pronounced pathology, including degeneration of digestive tubules and approx. 50% mortality, although it could not be confirmed whether mortality was directly and exclusively attributable to the infection (Bøgwald et al., 2022). Berthe et al. (2004) concluded that Mytilus edulis is rarely significantly affected by Marteilia sp. However, occasions have been recorded of nearly 100% mortality when British spat have been transferred from a ‘disease-free area’ to areas in France were Marteilia sp. are present. This suggests that there is a severe potential risk if naive spat are moved around the UK from northern waters into southern waters where the disease is resident (enzootic) or if increased temperatures allow the spread of Marteilia sp. northwards towards the naive northern populations. In addition, rising temperatures could allow increased densities of the Marteilia sp. resulting in heavier infections which can lead to mortality. Vibrio spp., particularly Vibrio splendidus, have been linked to abnormal mortality events (up to 99% mortality) in wild and cultured mussel populations (Bechemin et al., 2014; Cheikh et al., 2016). Experimental exposure of adult Mytilus edulis to highly pathogenic strains has produced cumulative mortality ranging from 17 to 83% depending on family lineage, indicating both high susceptibility and moderate heritability of resistance traits (Ajithkumar et al., 2024, 2025). Challenge studies with Vibrio spp. suggest that some populations are resistant to naturally occurring doses, with effects typically only observed at high concentrations(approx. 108 CFU (colony-forming units, an estimate of viable microbial cells)/ml, vs approx. 105 CFU/ml found in the environment), and some populations retaining some resistance even to the higher doses (Charles et al., 2020). Vibrio infection can also disrupt the native microbiota, contributing to dysbiosis and mortality (Cheikh & Travers, 2022). Mussels experimentally exposed to Vibrio splendidus and Pseudomonas fluorescens showed a 4.9% increase in cell mortality after four hours, indicating potential acute effects (Gendre et al., 2023). Larval stages are particularly vulnerable to microbial pathogens. Exposure to naturally occurring concentrations of Vibrio spp. has been shown to reduce larval viability and development (De Rijcke et al., 2016), with experimental challenge causing up to 98% mortality within five days (Eggermont et al., 2017; Wang et al., 2021). Similarly, toxic dinoflagellates such as Karlodinium armiger can cause substantial mortality in both embryos and larvae, with natural blooms affecting recruitment and survival in wild populations (Binzer et al., 2018). Other microbial organisms have been detected in European Mytilus edulis populations, with potential but currently uncertain impacts on health. Francisella halioticida has been recorded in wild mussels in Normandy, France and in the Tamar estuary, UK, where mass mortality events have occurred, although no causal link has yet been proven (Bouras et al., 2023; Cano et al., 2022). Experimental infection of adults caused up to 36% mortality at very high bacterial doses, though lower, more ecologically relevant, doses produced no significant effects (Bouras et al., 2023). Protozoan parasites, including Cryptosporidium spp. and Toxoplasma gondii, can be bioaccumulated by mussels for at least 21 days (Bigot-Clivot et al., 2022), with haemocytes responding to Toxoplasma gondii exposure, although no measurable pathology was reported for Cryptosporidium spp. (Le Guernic et al., 2020). These findings indicate that while these pathogens can be taken up and retained by mussels, direct effects on survival and condition remain unclear, and further investigation is needed to assess their ecological significance. Historical records indicate that subtidal Mytilus edulis beds in the Wadden Sea have suffered severe declines associated with disease outbreaks, particularly in combination with other pressures such as intensive fishing. Following such declines, populations have shown partial recovery over decades, suggesting that while adults can survive endemic pathogen presence, recruitment and long-term population stability are vulnerable to novel pathogen introduction (Reise & Buschbaum, 2017, cited in Ricklefs et al., 2020). A further emerging microbial disease risk is transmissible disseminated neoplasia. Genetic evidence indicates that a clonally transmissible cancer lineage originating in Mytilus trossulus has crossed species boundaries and infected Mytilus edulis populations in Europe, where outbreaks have been associated with extremely high mortality (90 to 100%) affecting both juvenile and adult mussels (Benabdelmouna & Ledu, 2016; Yonemitsu et al., 2019). Although such outbreaks appear spatially restricted, they demonstrate the potential for severe population-level impacts following introduction of novel transmissible pathogens. Sensitivity AssessmentThere was no evidence of mortality in Alaria esculenta due to microbial infections. Mytilus edulis is host to a range of microbial pathogens, including Marteilia spp., Vibrio spp., Francisella halioticida, protozoan parasites such as Cryptosporidium spp. and Toxoplasma gondii, and other bacterial and protozoan organisms. While Marteilia spp. infections can cause reduced condition and occasionally high mortality in naive populations, other pathogens such as Francisella halioticida or Vibrio spp. may cause moderate mortality under high exposure, with effects highly dependent on dose, environmental context, and host genetics. The impacts of protozoans are less clear, with some immune responses but no confirmed widespread mortality. Bower (2010) noted that although Marteilia was a potentially lethal pathogen of mussels, most populations were not adversely affected by marteilioisis, but that in some areas, mortality can be significant in mariculture (Berthe et al., 2004). The resultant population would be more sensitive to other pressures, even where the disease only resulted in a reduced condition. A precautionary resistance of ‘Medium’ is suggested, with a resilience of ‘High’ and sensitivity of ‘Low’. | MediumHelp | HighHelp | LowHelp |
Removal of target species [Show more]Removal of target speciesBenchmark. Removal of species targeted by fishery, shellfishery or harvesting at a commercial or recreational scale (targeted removal pressure definition). EvidenceAlaria esculenta has recently received commercial interest as a consumable product called “Sea Vegetables” or “Atlantic Wakame Kelp”. However, no studies examining the effect of commercial extraction of Alaria esculenta biotopes were found. Removal of the algal canopy would expose the understorey fauna and flora to increased desiccation during low tide. Experimental macroalgal canopy removal experiments conducted in the Isle of Man (Hawkins & Harkin, 1985) found that following the removal of the macroalgal canopy the understorey encrusting red algae became bleached and died within a week. Mytilus edulis settlement has also been found significantly higher near Alaria esculenta and is thought to increase beneath Alaria esculenta canopies (Bégin et al., 2004). Therefore, any loss of Alaria esculenta due to commercial extraction may dramatically affect the understorey community. Traditionally Laminaria digitata was used on agricultural lands as fertilizers; now Laminaria spp. are used in a range of different products, with their alginates used in the cosmetic, pharmaceutical and agri-food industries (Kervarec et al., 1999; McHugh, 2003). Collection of Laminaria digitata by mechanical harvesting (trawling) is not done in the UK, (Netalgae, 2012). Trawling, used to harvest Laminaria hyperborea in Norway results in whole alga being removed from the substratum, and substantial scouring of the substratum, indicating that the use of trawls in a Laminaria digitata biotope is likely to detrimentally affect the biotope, regardless of the target species. In France, Laminaria digitata is harvested with a ‘Scoubidou’, a curved iron hook which is mechanically operated. This device is considered to be selective; only harvesting individuals older than 2 years (Arzel, 2002). France reportedly harvests 75,000t kelp, mainly consisting of Laminaria digitata annually (FAO, 2007). Davoult et al. (2011) suggested that the maintenance of a sustainable crop of Laminaria digitata was possible if the industry continues employing small vessels evenly dispersed along the coastline. This could protect against habitat fragmentation and buffer over exploitation (Davoult et al., 2011). A fallow period of 18 to 24 months has been suggested for Laminaria digitata in France, where competition between the juvenile sporophytes of Laminaria digitata and Saccorhiza polyschides was indicated as a threat to the continued harvesting effort of Laminaria digitata (Engelen et al., 2011). Canopy removal of Laminaria digitata has been shown to reduce shading, resulting in the bleaching of sub-canopy algae (Hawkins & Harkin, 1985). Harvesting may also result in habitat fragmentation, a major threat to this biotope’s ecosystem functioning (Valero et al., 2011). Mytilus edulis may be targeted as bait or food by fishers (Holt et al., 1998). However, Mytilus edulis in this biotope occur in patches rather than a continuous bed. Therefore, it is highly unlikely that the mussels in this biotope would be targeted by dredging activities at high tide. Even hand-harvesting for mussels at low tide is likely to significantly deplete the biomass of mussels within this biotope (Smith & Murray 2005). Sensitivity AssessmentBoth characterising species are targeted for commercial use, although evidence of the effects of harvesting Alaria esculenta was lacking. If it is assumed that the effects of Alaria harvesting are similar to those of Laminaria digitata harvesting, then resistance would be assessed as ‘None’. Resilience is ‘High’, so the biotope’s sensitivity to this pressure is ‘Low’. | NoneHelp | HighHelp | LowHelp |
Removal of non-target species [Show more]Removal of non-target speciesBenchmark. Removal of features or incidental non-targeted catch (by-catch) through targeted fishery, shellfishery or harvesting at a commercial or recreational scale (non-targeted removed pressure definition). EvidenceIncidental/accidental removal of Alaria esculenta is likely to cause similar effects to that of direct harvesting; hence, the same evidence has been used for both pressure assessments. Alaria esculenta has recently received commercial interest as a consumable product called “Sea Vegetables” or “Atlantic Wakame Kelp”. However, no studies examining the effect of commercial extraction of Alaria esculenta biotopes were found. Removal of the algal canopy would expose the understorey fauna and flora to increased desiccation. Experimental macroalgal canopy removal experiments conducted in the Isle of Man (Hawkings & Harkin, 1985) found that following the removal of the macroalgal canopy the understorey encrusting red algae became bleached and died within a week. Mytilus edulis settlement has also been found significantly higher in close proximity to Alaria esculenta and is thought to increase beneath Alaria esculenta canopies (Bégin et al., 2004). Therefore, any loss of Alaria esculenta, as a result of commercial extraction, may dramatically affect the understorey community. Traditionally Laminaria digitata was added to agricultural lands as fertilizers; now Laminaria species are used in a range of different products, with its alginates used in the cosmetic, pharmaceutical and agri-food industries (Kervarec et al., 1999; McHugh, 2003). Laminaria digitata is harvested with a ‘Scoubidou’ (a curved iron hook which is mechanically operated) in France. This device is considered to be selective- only harvesting individuals older than 2 years (Arzel, 2002). France reportedly harvests 75,000t kelp, mainly consisting of Laminaria digitata annually (FAO, 2007). The loss of Laminaria digitata would represent a significant change to IR.HIR.KFaR.Ala.Ldig. Corallina officinalis is collected for medical purposes; the fronds are dried and converted to hydroxyapatite and used as bone forming material (Ewers et al. 1987). It is also sold as a powder for use in the cosmetic industry. Moderate trampling on articulated coralline algal turf in the New Zealand intertidal (Brown & Taylor 1999; Schiel & Taylor 1999) resulted in reduced turf height, declines in turf densities, and loss of crustose bases in some case probably due to loss of the canopy algae and resultant desiccation. Calcification is thought to be an adaptation to grazing and sediment scour (Littler & Kauker 1984). Corallina officinalis produces spores over a protracted period and can colonize artificial substratum within one week in the intertidal (Harkin & Lindbergh 1977; Littler & Kauker 1984). The crustose base enables Corallina officinalis to survive the loss of fronds. Sensitivity assessment. There is little published evidence for the effects of commercial harvesting of Alaria esculenta. If it is assumed that all canopy forming kelp are removed then resistance would be assessed as ’None‘, resilience would be assessed as ’Medium‘. Sensitivity has been assessed as ’Medium‘. Within IR.HIR.KFaR.AlaAnCrSp and IR.HIR.KFaR.Ala.Myt, monospecific canopies of Alaria esculenta are expected to recover quicker than mixed canopies of Laminaria digitata (as in IR.HIR.KFaR.Ala.Ldig). | NoneHelp | MediumHelp | MediumHelp |
Introduction or spread of invasive non-indigenous species (INIS) Pressures
Use [show more] / [show less] to open/close text displayed
| Resistance | Resilience | Sensitivity | |
The American slipper limpet, Crepidula fornicata [Show more]The American slipper limpet, Crepidula fornicataEvidenceThe American slipper limpet Crepidula fornicata was introduced to the UK and Europe in the 1870s from the Atlantic coasts of North America with imports of the eastern oyster Crassostrea virginica. It was recorded in Liverpool in 1870 and the Essex coast in 1887-1890 and has spread into waters around mainland Europe (Blanchard, 1997, 2009; Bohn et al., 2012, 2013a, 2013b, 2015; De Montaudouin et al., 1999, 2018; Hinz et al., 2011; Helmer et al., 2019; McNeill et al., 2010; Powell-Jennings & Calloway, 2018; Preston et al., 2020; Stiger-Pouvreau & Thouzeau, 2015). It ranges from the Baltic Sea, the Kattegat and Skagerrak, the North Sea coasts of the UK, Germany, and Belgium, through the English Channels and into the Irish sea coasts of Ireland and south Wales with records in east and west Scotland, Northern Ireland, northwest France, Spain and south into the Mediterranean (NBN, 2024; OBIS, 2026). Abundances at its northern and southern extremes may be low but densities in UK and France are often over 1000 individuals/m2 and it may carpet the seafloor in the Solent and Essex. In the UK, it was reported to reach abundances of >1000 individuals/m2 (max. 2,748 individuals/m2) in the Milford Harbour Waterway (Bohn et al., 2012), 84 individuals/m2 in Portsmouth, 174 individuals/m2 in Langstone and 306 individuals/m2 in Chichester harbours in 2017 (Helmer et al., 2019). In France, it has been reported to reach >4,700 individuals/m2 in the Bay of Marennes-Oleron, France, 11.6 tonnes/ha in Bay of Mont-Saint-Michel, 8.2 tonnes/ha in the Bay of Brest and 2.8 tonnes/ha in the Bay of Saint-Brieuc (Blanchard, 2009; Bohn et al., 2012, 2015; Powell-Jennings & Calloway, 2018). Its density and ability to spread within and between sites (e.g., bays) depend on the availability of suitable habitat, competition with other species, larval retention within the site, human activities (e.g., dredging), and seasonal temperatures, particularly in the intertidal zone. For example, the Crepidula fornicata population in the Bay of Mont-Saint-Michel grew by 50% between 1996 and 2004, covering 25% of the area at high density (51 to 100% cover), aided by local oyster farming and shellfish dredging (Blanchard, 2009). However, in Arcachon Bay, France, Crepidula fornicata was limited to only 155 tonnes in 1999 and 312 tonnes in 2011 (De Montaudouin et al., 2001, 2018). It was confined to muddy sediments, which accounted for only approx. 8% of the bay and were colonized by Zostera beds. These areas represented just 0.4% of the suspension feeder biomass compared to the oysters Magallana gigas in the bay, and there was no indication of increasing biomass over a 12-year period. In addition, benthic trawling was prohibited in the bay (De Montaudouin et al., 2001, 2018). As a result, De Montaudouin et al. (2018) concluded that Crepidula fornicata was not invasive in the Bay of Arcachon. Crepidula fornicata is recorded from shallow, sheltered bays, lagoons and estuaries or the sheltered sides of islands, in variable salinity (from 18 to 40 PSU) although it prefers around 30 PSU (Tillin et al., 2020). Larvae require hard substrata for settlement. It prefers muddy gravelly, shell-rich, substrata that include gravel, or shells of other Crepidula, or other species e.g., oysters, and mussels. It is highly gregarious and seeks out adult shells for settlement, forming characteristic ‘stacks’ of adults. It has also recorded from rock, artificial substrata, and Sabellaria alveolata reefs (Blanchard, 1997, 2009; Bohn et al., 2012, 2013a, 2013b, 2015; De Montaudouin et al., 2018; Hinz et al., 2011; Helmer et al., 2019; Powell-Jennings & Calloway, 2018; Preston et al., 2020; Stiger-Pouvreau & Thouzeau, 2015; Tillin et al., 2020). In the eastern Solent harbours of Portsmouth, Langstone, and Chichester, 75% to 98% of Crepidula larvae settled on dead Crepidula shells, while approx. 4% settled on stone, 2.5% on live Crepidula, 0.3% oyster shell, 0.6% cockle shell, 0.3% winkle shell and 0.1% periwinkle shell (Preston et al., 2020). In the Milford Harbour Waterway, the highest densities of Crepidula were found in areas of sediment with hard substrata, e.g., mixed fine sediment with shell, or gravel or both but, while Crepidula density increased as gravel cover increased in the subtidal, the reverse was found in the intertidal (Bohn et al., 2015). However, gravel formed the base of most stacks of Crepidula in the intertidal, which suggested that initial colonization occurred on available hard substrata (i.e., gravel) in the absence of adult shells of Crepidula. The availability of hard substrata (e.g., gravel) may only restrict initial colonization as higher densities of Crepidula functions as substrata for subsequent colonization (Thieltges et al., 2004; Blanchard, 2009). Bohn et al. (2015) also noted that Crepidula density was low in areas of homogenous fine sediment and absent in areas dominated by boulders. Bohn et al. (2015) suggested that wave action (exposure) probably prevented the establishment of large numbers of Crepidula in high-energy areas. However, Hinz et al. (2011) recorded Crepidula off the Isle of Wight in the English Channel, at approx. 60 m on rough ground in areas of high tidal flow. Tillin et al. (2020) suggested that the effect of oscillatory wave meditated flow might have a greater effect on Crepidula than tidal flow, presumably due to mobilization of the substratum. Similarly, Crepidula was absent from sandy substrata in Swansea Bay but was most abundant in the shelter of the breakwater at Swansea east site (Powell-Jennings & Calloway, 2018). Crepidula fornicata has been recorded from the lower intertidal to approx. 160 m in depth but it most common in the shallow subtidal and low water springs (Blanchard, 1997; Thieltges et al., 2003; Bohn et al., 2012, 2015; Hinz et al., 2011; OBIS, 2026; Tillin et al., 2020). Bohn et al. (2012, 2013a, 2013b, 2015) suggested that extreme conditions in the intertidal limited its upward distribution due to early post-settlement mortality. It reached its highest densities in the lower shore (below approx. 0.7 m) and was absent from high tidal level (approx. 1.8 m) in the Milford Harbour Waterway (Bohn et al., 2015).
The density of Crepidula populations in the northern Europe (Germany, Denmark, and Norway) is significantly lower (<100 individuals/m2) than in southern waters. Thieltges et al. (2004) reported that the population of Crepidula was affected strongly by cold winters in the Wadden Sea. The winters of 2001 and 2003 resulted in approx. 56 to 64% mortality of intertidal Crepidula and up to 97% on one mussel bed, compared to only 11 to 14% in southern areas without frost. Crepidula almost vanished from the Wadden Sea after the 1978/79 winter and took ten years to recover due to moderate winters which regularly affected the population. Similarly, 25% mortality was observed in Crepidula populations on the south coast of the UK after the extreme 1962/63 winter (Crisp, 1964, Bohn et al., 2012). Thieltges et al. (2003) suggested that global warming way allow Crepidula populations become more abundant in northern Europe. Valdizan et al. (2011) noted higher water temperatures between 2000 to 2001 and 2006 to 2007 together with elevated chlorophyll-a corresponded to an increase in gametogenesis and the duration of broods in Crepidula population in Bournerf Bay, France. They suggested that rising temperatures in northern Europe could increase its reproductive success due favourable breeding temperatures and increased phytoplankton (Valdizan et al., 2011). Nehls et al. (2006) noted that the decline in mussel (Mytilus edulis) beds in the Wadden Sea was due to mild winters that favoured non-native oysters (Magallana gigas) and slipper limpets, which coexisted with the mussels. There is currently a lack of evidence of Crepidula fornicata colonization on bedrock in the infralittoral or circalittoral. Tillin et al. (2020) suggested that Crepidula could colonize circalittoral rock due to its presence on tide-swept rough grounds in the English Channel (Hinz et al., 2011). However, Hinz et al. (2011) reported that Crepidula fornicata only dominated one assemblage (with an average of 181 individuals per trawl) on gravel substratum with boulders. Bohn et al. (2015) noted that Crepidula occurred at low density or was absent in areas dominated by boulders, and Bohn et al. (2013a, 2013b, 2015) and Preston et al. (2020) showed that while Crepidula could settle on slate panels or ‘stone’ it preferred shell, especially that of conspecifics. Sensitivity AssessmentThere is currently a lack of evidence of Crepidula fornicata colonization on bedrock in the infralittoral or circalittoral. Tillin et al. (2020) suggested that Crepidula could colonize circalittoral rock due to its presence on tide-swept rough grounds in the English Channel (Hinz et al., 2011), but considered high energy wave action and macroalgal communities would render these habitats unsuitable. At present, there is Insufficient Evidence to suggest that this biotope is sensitive to colonization by Crepidula fornicata. | Insufficient evidence (IEv)Help | Insufficient evidence (IEv)Help | Help |
The carpet sea squirt, Didemnum vexillum [Show more]The carpet sea squirt, Didemnum vexillumEvidenceThe carpet sea squirt Didemnum vexillum (syn. Didemnum vestitum; Didemnum vestum) is a colonial ascidian with rapidly expanding populations that have invaded most temperate coastal regions around the world (Kleeman, 2009; Stefaniak et al., 2012; Tillin et al., 2020). It is an ecosystem engineer that can change or modify invaded habitats and alter biodiversity (Griffith et al., 2009; Mercer et al., 2009). A lack of published descriptions and an incomplete historical record has led to the widespread misidentification of Didemnum vexillum and it is often recorded as Didemnum spp. Hence, the native range of the species is not known conclusively (Lambert, 2009; Stefaniak et al., 2012; McKenzie et al., 2017; Holt, 2024). However, molecular data and limited historical evidence have suggested that the species may be native to Japan with its native range possibly extending into continental Asia and north-western Pacific (Stefaniak et al., 2012; Tillin et al., 2020; Holt, 2024). Previously unrecorded populations of a colonial ascidian have been recently identified as Didemnum vexillum (Tillin et al., 2020). Didemnum vexillum has colonized and established populations in the northeast Pacific, Canadian and USA coast; New Zealand; France, Spain, and the Wadden Sea, Netherlands; the Mediterranean Sea and Adriatic Sea (Bullard et al., 2007; Coutts & Forrest, 2007; Dijkstra et al., 2007; Valentine et al., 2007a; Valentine et al., 2007b; Lambert, 2009; Hitchin, 2012; Tagliapietra et al., 2012; Gittenberger et al., 2015; Vercaemer et al., 2015; McKenzie et al., 2017; Cinar & Ozgul, 2023; Holt, 2024). In the UK, Didemnum vexillum has colonized Holyhead marina and Milford Haven, Wales; the west coast of Scotland (marinas around Largs, Clyde, Loch Creran and Loch Fyne), South Devon (Plymouth, Yealm, and Dartmouth estuaries), the Solent, northern Kent, Essex, and Suffolk coasts (Griffith et al., 2009; Lambert, 2009; Hitchin, 2012; Minchin & Nunn, 2013; Bishop et al., 2015; McKenzie et al., 2017; Tillin et al., 2020, Holt, 2024; NBN, 2024). Didemnum vexillum has the ability to rapidly overgrow and displace on other sessile organisms such as other colonial ascidians (Ciona intestinalis, Styela clava, Ascidiella aspera, Botrylloides violaceus, Botryllus schlosseri, Diplosoma listerianium and Aplidium spp.), bryozoan, hydroids, sponges (Clione celata and Halichrondria sp.), anemone (Diadumene cincta), calcareous tube worms, eelgrass (Zostera marina), kelp (Laminaria spp. and Agarum sp.), green algae (Codium fragile subsp. fragile), red algae (Plocamium, Chondrus crispus and bush weed Agardhiella subulata), brown algae (Ascophyllum nodosum, Sargassum, Halidrys, Fucus evanescens and Fucus serratus), calcareous algae (Corallina officinalis), mussels (Mytilus galloprovincialis, Perna canaliculus and Mytilus edulis), barnacles, oysters (Magallana gigas, Ostrea edulis and Crassostrea virginica), sea scallops (Placopecten magellanicus), or dead shells (Dijkstra et al., 2007; Gittenberger, 2007; Valentine et al., 2007a; Valentine et al., 2007b; Griffith et al., 2009; Carman & Grunden, 2010; Dijkstra & Nolan, 2011; Groner et al., 2011; Hitchin, 2012; Tagliapietra et al., 2012; Minchin & Nunn, 2013; Gittenberger et al., 2015; Long & Grosholz, 2015; Vercaemer et al., 2015). Didemnum vexillum has been found colonizing the stipes of Laminaria spp. in the Gulf of Maine (Dijkstra et al., 2007) and in Norway (Legrand et al., 2025). However, it has not been recorded in sites exposed to wave action, that is ‘very wave exposed’, ‘wave exposed’ and ‘moderately wave exposed’ (sensu MNCR, Hiscock, 1996), especially in the intertidal where wave action is not ameliorated by depth (see Hiscock, 1983). This species requires suitable hard substrata for successful settlement and the establishment of colonies. It can grow quickly and can establish large colonies of dense encrusting mats on a variety of hard substrata (Valentine et al., 2007a; Griffith et al., 2009; Lambert, 2009; Groner et al., 2011; Cinar & Ozgul, 2023). Mats can be up to several meters in area, covering large portions of the seafloor (Mercer et al., 2009). Gittenberger (2007) stated that invasive Didemnum sp. was a threat to native ecosystems by its ability to overgrow virtually all hard substrata present. Suitable hard substrata can include rocky substrata such as bedrock gravel, pebble, cobble, or boulders (Tillin et al., 2020). Didemnum vexillum has been reported colonizing these types of hard substrata in the USA, Canada, northern Kent and the Solent (Bullard et al., 2007; Valentine et al., 2007a; Valentine et al., 2007b; Hitchin, 2012; Vercaemer et al., 2015; Tillin et al., 2020). It is therefore likely that the substrate in this biotope is suitable for Didemnum vexillum colonisation. In addition, the depth range at which Laminaria hyperborea biotopes are found (0 to 30 m) overlaps with the depth range that is suitable for suitable for Didemnum vexillum colonization. Didemnum vexillum has been recorded from less than 1 m to at least 81 m deep (Bullard et al., 2007; Tagliapietra et al., 2012; Tillin et al., 2020). Didemnum vexillum tolerates a wide range of environmental conditions including temperature and salinity (Herborg et al., 2009; Tillin et al., 2020). Didemnum vexillum can withstand a wide range of salinities from 20 to 44 PSU, is commonly found in marine waters around 33 PSU but is unable to survive in salinities below 20 PSU (Bullard & Whitlatch, 2009; Groner et al., 2011; Tillin et al., 2020). It has been recorded in estuarine conditions and tidal lagoons (Dijkstra et al., 2007; Tillin et al., 2020). In the Lagoon of Venice, Mediterranean, Didemnum vexillum is found in a mean salinity value of 30 PSU. It was absent in low salinity, such as the estuary and around the saltmarshes, but well established in the euhaline and tidally well flushed zones of the Lagoon of Venice (Tagliapietra et al., 2012). Similar results were found in Connecticut and Rhode Island where Didemnum vexillum was not found in environments with salinity less than 20 PSU (Bullard & Whitlatch, 2009). However, in the Wadden Sea, colonies of Didemnum vexillum were abundant in salinities between 17.91 to 25.97 PSU (Gittenberger, 2007; Gittenberger et al., 2015). Didemnum vexillum is a temperate species that can survive a broad temperature range of -2 to 24°C, with an upper survival limit suggested to be 25°C (Bullard et al., 2007; Valentine et al., 2007a; Herborg et al., 2009; Kleeman, 2009; McKenzie et al., 2017; Holt, 2024). It thrives best at 14 to 20°C, with optimal growth temperature between 14 to 18°C during summer months (May, June, September, October) (Gittenberger, 2007; Kleeman, 2009; McKenzie et al., 2017). Reinhart et al. (2012) examined the effects of water flow and hydrodynamics on the encrusting and tendril forms of Didemnum vexillum. They reported that a current speed of approx. 7.6 m/s was required to induce fragmentation of tendrils, but that natural tidal flow alone was insufficient to cause fragmentation of tendrils. They suggested that rare instances of wave action such as storms that resulted in wave orbital velocities of approx. 8 m/s or (more likely) human activity could cause fragmentation of tendrils. Reinhart et al. (2012) noted that the tensile strength of Didemnum vexillum was an order of magnitude higher than Botrylloides sp. and was similar to that of Alcyonium digitatum. Alcyonium digitatum is reported from sheltered to very wave exposed conditions, but in the sublittoral. Reinhart et al. (2012) also suggested that seasonal changes in the condition of Didemnum vexillum reduced the tensile strength of colonies and was associated with the period of greater larval production, and implied that fragmentation aided dispersal. The oscillatory nature of wave-mediated water flow (wave orbital velocities) combined with wave pressure in the lacerating zone, where breaking wave causes multidirectional strong water movement (Hiscock, 1983), would probably dislodge and break up Didemnum vexillum colonies, prevent them from forming suffocating mats, and restrict the colonies to crevices and overhangs. However, it is unclear if moderately wave exposed conditions would be adequate to prevent Didemnum vexillum from developing extensive mats in the summer months when wave action is typically reduced. Hitchin (2012) suggested that the presence of Didemnum vexillum in Whitstable, Kent was contrary to its then known habitat preferences. Sensitivity AssessmentThere is no evidence of Didemnum vexillum colonizing this biotope in the UK. However, it has been recorded in similar kelp habitats in Norway (Järnegren et al., 2023). Didemnum vexillum requires hard substrata for successful colonization, so it could colonize the bedrock that characterizes this biotope. Didemnum vexillum can overgrow sessile organisms, including kelp Laminaria sp. However, no direct evidence was found on how Didemnum vexillum affects kelp or if it contributes to mortality (Järnegren et al., 2023), although epifaunal growth by Membranacea membrancea was reported to reduce the physical strength of Laminaria digitata fronds and make them susceptible to removal by wave action (Krumhansl et al., 2011). In addition, overgrowth by epiphytes contributed to the decline of Saccharina latissima in Norway (Andersen et al., 2011). However, Didemnum vexillum may compete for light and space with kelp and epifauna and could interfere with recruitment, which could lead to the mortality of some epifauna, the loss of kelp, and a reduction in biodiversity. Didemnum prefer sheltered conditions so the wave exposed and tidally swept conditions that characterize this biotope may mitigate its abundance. Therefore, a resistance of ‘Medium’ (some mortality, <25%) is suggested as a precaution. Resilience is likely to be ‘Very low’ as Didemnum vexillum would need to be physically removed to allow recovery. Hence, sensitivity to invasion by Didemnum is assessed as ‘Medium’. However, confidence in the assessment is ‘Low’ due to the lack of direct evidence of damage to kelp beds. | MediumHelp | Very LowHelp | MediumHelp |
The Pacific oyster, Magallana gigas [Show more]The Pacific oyster, Magallana gigasEvidenceThe Pacific oyster, Magallana (syn. Crassostrea) gigas, is native to warm temperate regions from the northwest Pacific to Japan and northeast Asia, including Cape Mariya (Russia) to Hong Kong (China) (Carrasco & Baron, 2010; GBNNSIP, 2011, 2012). It is a fast-growing and tolerant species that has become a successful invader in the coastal waters of all continents, aside from Antarctica (Wrange et al., 2010; Carrasco & Baron, 2010; Padilla, 2010). It was initially introduced for aquaculture in Europe and the UK in the 1960s due to a decline in the Portuguese oyster (Crassostrea angulata) and the European flat oyster (Ostrea edulis) (Spencer et al., 1994; GBNNSIP, 2011, 2012; Humphreys et al., 2014, cited in Alves et al., 2021; Hansen et al., 2023). It was also introduced to the northeast Adriatic Sea (Ezgeta-Balic et al., 2019) and southwest England from France, possibly via fouling on ships (GBNNSIP, 2011, 2012; Padilla, 2010; Ezgeta-Balic et al., 2019). Magallana gigas has a high fecundity, a long-lived pelagic larval phase (2 to 4 weeks) and can produce up to 200 million eggs during spawning (Herbert et al., 2012, 2016; Alves et al., 2021; Wood et al., 2021; Hansen et al., 2023). Hence, as a broadcast spawner, it has a high dispersal potential of more than 1000 km (Padilla, 2010; Wood et al., 2021). Although larval mortality can be as large as 99% due to sensitivity to environmental conditions (Alves et al., 2021), adults are long-lived so that populations can survive with infrequent recruitment (Padilla, 2010). Larval dispersal has facilitated the establishment of populations in various regions, such as the Oosterschelde estuary in the Netherlands and the Scandinavian coastlines, where northward drift on tidal and wind-driven currents has been suggested (Hansen et al., 2023). Offshore structures and aquaculture operations can enhance spread (Wood et al., 2021). Magallana gigas is an ecosystem engineer and can dramatically change habitat structure when it invades. Once successfully settled, groups of Pacific oysters may form dense aggregations, potentially forming a reef, which in some regions can reach densities of 700 individuals/m2 (Herbert et al., 2012, 2016). Once, the density of live or dead Pacific oysters reaches or exceeds 200 individuals/m2, little of the underlying substratum remains visible (Herbert et al., 2016). These reefs can stabilize the sediment surface locally (Troost, 2010). When such reefs are formed or, particularly when the species colonizes soft sediments such as mud or sand, it can change and affect local communities, by creating hard substrata for mobile species, which might not otherwise be present before the invasion (Padilla, 2010). However, Hansen et al. (2023) suggested that no immediate ecosystem risk is observed where the Pacific oyster occurs sporadically. Settlement requires hard substrata, including rock, bedrock, chalk, bare boulders, cobbles and pebbles and shells (Kochmann, 2012, Kochmann et al., 2013; McKinstry & Jensen, 2013; Herbert et al., 2016; Tillin et al., 2020). Magallana gigas also attaches to available hard materials in mixed sediment environments such as shingle and sand within otherwise unsuitable mudflats (Spencer et al., 1994; McKinstry & Jensen, 2013; Tillin et al., 2020). Populations of Magallana gigas have been found wave exposed rocky shores to wave sheltered soft sediment environments and it has been described as a habitat generalist (Troost, 2010; Kochmann, 2012, Kochmann et al., 2013). For example, in Scotland, wild Magallana gigas are mainly located in the lower intertidal on bedrock, bedrock encrusted with barnacles, within bedrock crevices, and large and small boulders (Cook et al., 2014). Patches of Pacific oyster reefs have been recorded on littoral rock in Kent, southern England and on littoral sediments in southern England, the North Sea, and the English Channel (Herbert et al., 2012, 2016; Morgan et al., 2021). Magallana gigas has been reported from estuaries growing on intertidal mudflats and sandflats, and other soft sediments (Padilla, 2010; Herbert et al., 2016; Cabral et al., 2020). The settlement of spat on hard substrata within sediments has been observed in the estuaries of the River Dart, Exe, Fal, Fowey, Tamar, Teign, and Yealm in Devon and Cornwall, the Menai Straits, Wales and large estuaries of Lough Swilly, Lough Foyle and the Shannon in Ireland, and the Tagus Estuary in Portugal (Spencer et al., 1994; Kochmann, 2012, Kochmann et al., 2013; Cabral et al., 2020). In Lough Swilly, Lough Foyle and the Shannon, the Pacific oyster was often associated with intertidal mud or sandflats (Kochmann et al., 2013). In contrast, the Pacific oysters were absent from sandflat areas in Poole Harbour (McKinstry & Jensen, 2013). Although shorelines comprised of mainly mud were suggested to be unsuitable for spat settlement (Spencer et al., 1994), the presence of smaller hard substrata, such as shells or pebbles, can enable larvae to settle (Tillin et al., 2020). For example, in the River Teign estuary, Pacific oyster settlement was observed on shell-covered ground mainly attached to mussel shells, and occasionally attached to cockles, stones and common periwinkle (Littorina littorea) shells on a mud flat in the estuarine intertidal zone otherwise mainly comprised of sand and mud (Spencer et al., 1994). In addition, the Blue Lagoon on the north shore of Poole Harbour had the highest abundance of oysters on mud mixed with shingle and shell (McKinstry & Jensen, 2013). Outside of the Blue Lagoon, oysters were also recorded on mixed substrata composed of mud, gravel, and shell (McKinstry & Jensen, 2013). Tillin et al. (2020) concluded that while successful invasions occurred on mudflats, Magallana gigas prefers mixed substrata. Fine mud sediments without hard substrata (such as small stones, gravel, and shell) are unlikely to be suitable (Tillin et al., 2020). The speed of Magallana gigas reef formation on soft substrata seems to be dependent on the amount of hard substrata present (Troost, 2010). Bergstrom et al. (2021) reported that the presence of Magallana gigas was partially dependent on increasing gravel content up to 15% but remained stable with increasing percentages (measured up to 80%). While often described as an intertidal and shallow subtidal species, Magallana gigas has been observed across a broader depth range. Although rocky habitats deeper than 10 m are generally considered unsuitable, it has been recorded down to 42 m in the Oosterschelde, Netherlands (Herbert et al., 2012, 2016; Tillin et al., 2020; Smaal et al., 2009). It frequently occurs between Mean High Water and Mean Low Water in intertidal zones but has also been recorded at 1 to 10 m depth in regions like Sweden, Ireland, and the UK (Kochmann et al., 2013; Herbert et al., 2016; Bergstrom et al., 2021). In Lough Swilly and Lough Foyle, Ireland, oysters were found on shallow subtidal mussel beds and mixed mud and sand habitats (Kochmann, 2012). In the Thames Estuary and parts of Essex and Kent, oysters have also been found subtidally, 2 to 3 m below chart datum (Tillin et al., 2020). Bergstrom et al. (2021) suggested the optimal depth in the Skagerrak is around 0.5 m, although presence is documented down to 5 m. In Lim Bay (Adriatic Sea), M. gigas occurs in the intertidal and shallow subtidal (down to 1 m), but not beyond 3 m depth (Stagličić et al., 2020). The species has not been recorded below extreme low water on rocky habitats, although it has been found subtidally on soft sediments in some areas (Herbert et al., 2012). The Pacific oyster prefers wide intertidal areas with shallow gradients; it is generally absent from steep shores (McKinstry & Jensen, 2013; Herbert et al., 2016; Tillin et al., 2020). In Ireland and the Solway Firth, it is more commonly found on intertidal shores over 40 to 50 m wide (Kochmann et al., 2013; Cook et al., 2014). It has been suggested that recruitment is enhanced, and abundances are higher in wave sheltered conditions (Robinson et al., 2005; Ruesink, 2007 cited in Teschke et al., 2020; Tillin et al., 2020). Teschke et al. (2020) found the abundance of Magallana gigas was significantly higher at wave-protected sites within the artificial harbours of Helgoland, North Sea, compared to wave exposed sites outside the harbours. The authors suggested that the successful colonization in wave-protected sites could be due to the relative retention of water masses in the harbours that reduces larval drift and whiplash effect on newly settled larvae. In addition, better growth and higher survival rates were observed at wave-protected sites, whereas mortality rates increased at wave exposed sites, due to the wave exposure causing dislodgement or detachment from the settlement substratum (Teschke et al., 2020; Tillin et al., 2020). Similarly, Bergstrom et al. (2021) noted that the occurrence of high densities of both Ostrea edulis and Magallana gigas decreased with increasing wave exposure. Magallana gigas can withstand a wide range of salinities (from 11 to 34 PSU), but no oysters were observed in areas on the west Swedish coast which had salinities less than 20 PSU (Wrange et al., 2010; Kochmann, 2012; Chu et al., 1996 cited in Tillin et al., 2020). Bergstrom et al. (2021) noted that in the Skagerrak, native and Pacific oyster densities increased with rising salinity above 15 to 27 PSU. Larvae can survive salinities between 19 to 35 PSU (Troost, 2010; Tillin et al., 2020). Growth of Pacific oysters can occur between 10 to 30 PSU (Troost, 2010). Carrasco & Baron (2010) suggested that Magallana gigas has successfully adapted to colonize a range of thermal niches. Temperature is important for the life cycle of the Pacific oyster and influences the establishment of feral and wild populations (Alves et al., 2021). Within its native range, Magallana gigas occurs in areas where the sea surface temperatures range from 14.0°C to 28.6°C in the warmest month of the year, and between -1.9°C and 19.8°C in the coldest month (Carrasco & Baron, 2010). Magallana gigas has a seasonal reproductive cycle (Alves et al., 2021). Spawning occurs in the summer months, when temperatures are 16 to 34°C and larvae require a water temperature of 18°C or above for successful development (Mann 1979; Troost, 2010; Kochmann, 2012; Ezgeta-Balic et al., 2020; Alves & Tidbury, 2022). In Poole, UK, spawning temperatures were estimated at 19.7°C (Alves & Tidbury, 2022). Ezgeta-Balic et al.’s (2020) study indicated that temperatures in the Mediterranean and the Adriatic were favourable for Pacific oyster larval development, with gametogenesis initiated at temperatures from around 10 to 15°C and spawning initiated at around 24°C. However, the lower thermal limit for spawning was recognized as 16°C (Carrasco & Baron, 2010) and once settled, larvae are unable to survive in temperatures below 3°C (Alves & Tidbury, 2022). Adults can survive in water temperatures up to 40°C and at low tide, freezing air temperatures as low as -17°C, depending on the salinity of the water in their shells (Troost, 2010; Tillin et al., 2020; Hansen et al., 2023). Growth of Pacific oysters occurs between 3 to 40°C (Troost, 2010; Kochmann, 2012). Dense macroalgal cover is unsuitable for the Magallana gigas (Herbert et al., 2012, 2016; Tillin et al., 2020), being rarely found under macroalgal cover in Northern Ireland, absent from exposed bedrock or large boulders with macroalgae cover in the Solway Firth, Scotland, and absent in Poole Harbour where there was competition with macroalgae (Kochmann, 2012, Kochmann et al., 2013; McKinstry & Jensen, 2013; Cook et al., 2014; Tillin et al., 2020). Fucus cover significantly reduced larval recruitment of the Pacific oyster in the Wadden Sea (Diederich, 2005). Hence, the Pacific oyster is more likely to colonize bare rock, boulders, or mussel beds without macroalgae (Diederich, 2005; Cook et al., 2014). Kochmann et al. (2013) suggested that macrophyte canopies prevent larvae from settling on the rock underneath and macroalgae fronds inhibit settlement and recruitment by exuding metabolites. Sensitivity AssessmentWhile most of the evidence suggests the environmental conditions within these biotopes are suitable for Magallana gigas, it is unlikely that they would be able to colonize this biotope without the removal of the macroalgal canopy. In addition, populations may be limited to low densities due to very wave exposed to wave exposed conditions. Therefore, this biotope is assessed as ‘Not Sensitive’ to this pressure. | HighHelp | HighHelp | Not sensitiveHelp |
Wireweed, Sargassum muticum [Show more]Wireweed, Sargassum muticumEvidenceSargassum muticum is a circumglobal invasive species (Engelen et al., 2015). It is recorded from Norway to Morocco and into the Mediterranean in the eastern Atlantic and from Alaska to Baja California in the eastern Pacific and from southern Russia to southern China in the western Pacific (Engelen et al., 2015). It colonizes a variety of habitats and can tolerate -1°C to 30°C and survive salinities below 10 PSU. Although fertilization does not occur below 15 PSU and growth of germlings is limited below 10°C it can complete its life cycle if temperatures are over 8°C for at least four months of the year (Engelen et al., 2015). However, its distribution is limited by the availability of hard substratum (e.g., stones >10 cm) and light (Staehr et al., 2000; Strong & Dring 2011; Engelen et al., 2015). It is most abundant between 1 and 3 m below mean water. But it has been recorded at 18 m or 30 m in the clear waters of California. However, it is a poor competitor under low light and only develops dense canopies in shallow areas (Engelen et al., 2015). Sargassum muticum was shown to replace and outcompete leathery, canopy-forming macroalgae such as Saccharina latissima, Halidrys siliquosa, and Fucus spp. and, to a lesser degree, understorey species such as Codium fragile, Chondrus crispus and Dictyota dichotoma in Limfjorden, Denmark between 1984 and 1997 (Staehr et al., 2000; Engelen et al., 2015; De Bettignies et al., 2021). The invasion in Limfjorden had stabilized by 2005 although many of the native macroalgal species continued to decline (Engelen et al., 2015). In Limfjorden, the distribution of Sargassum muticum was limited to areas with hard substratum, in particular stones >10 cm in diameter, while smaller stones, gravel and sand were unsuitable. It was most abundant between 1 and 4 m in depth but had low cover at 0 to 0.5 m and 4 to 6 m, in the turbid waters of the Limfjorden. Limfjorden is wave sheltered but wave exposure has been reported to restrict the growth and survival of Sargassum muticum (Staehr et al., 2000). Viejo et al. (1995) reported that Sargassum muticum transplanted to wave exposed shores in Spain experienced >80% breakages within a month and that the growth of undamaged plants was significantly lower than that of plants on sheltered shores. Similarly, Andrew & Viejo (1998) noted that Sargassum muticum was restricted to intertidal rockpools in wave exposed sites in the Bay of Biscay. Strong & Dring (2011) used canopy removal experiments to investigate inter- and intra-species competition between Sargassum muticum and Saccharina latissima in the Dorn, Strangford Lough, N. Ireland. The Dorn consists of tidal pools, very sheltered from wave action but with moderately strong tidal streams (1 to 2 knots). Sargassum muticum grew better in mixed stands with Saccharina latissima than in the highest-density monospecific stands examined. However, the growth of Saccharina was not affected by the proportion of Sargassum in mixed stands. They concluded that Saccharina was not impacted significantly by the alien species while Sargassum benefited from growth in mixed stands. Experimental manipulation of subtidal algal canopies in the San Juan Islands, Washington State, USA, showed that Sargassum muticum reduced the abundance of native macroalgae, including the kelp Laminaria bongardiana due to shading. However, the experimental removal of Sargassum resulted in the recovery of native species within about one year (Britton-Simmons, 2004; Engelen et al., 2015). The negative effects of Sargassum muticum on native macroalgae are mainly due to competition for light, rather than changes in nutrient availability, sedimentation or water flow (Britton-Simmons, 2004; Engelen et al., 2015). Sensitivity AssessmentThis biotope is found within the sublittoral with extreme to moderate wave exposure and strong tidal streams. The evidence above suggests that Sargassum muticum prefers wave sheltered, shallow sites in the sublittoral fringe. Competition with Sargassum is probably site-specific and dependent on local conditions, but it is highly unlikely that Sargassum will be able to colonize and survive in this biotope due to the high degree of wave exposure and tidal streams that characterize these biotopes. Therefore, resistance is assessed as ‘High’, resilience as ‘High’, and sensitivity is assessed as ‘Not Sensitive’. Overall, confidence is assessed as ‘Low’ due to evidence of variation and the site-specific nature of competition between native kelps and Sargassum muticum. | HighHelp | HighHelp | Not sensitiveHelp |
Wakame, Undaria pinnatifida [Show more]Wakame, Undaria pinnatifidaEvidenceUndaria pinnatifida (Wakame or Asian kelp) is a large brown seaweed and an Invasive Non-Indigenous Species (INIS) that could outcompete native UK kelp species (see Farrell & Fletcher, 2006; Thompson & Schiel, 2012; Brodie et al., 2014; Heiser et al., 2014; Arnold et al., 2016; Epstein & Smale, 2017; Epstein & Smale, 2018; Kraan, 2017; Epstein et al., 2019a,b; Tidbury, 2020). Undaria pinnatifida originates from Japan but is established currently on the coastlines of New Zealand, Australia, Northern France, Spain, Italy, the UK, Portugal, Belgium, Holland, Argentina, Mexico, and the USA (De Leij et al., 2017). Undaria pinnatifida was first recorded in the UK in the Hamble Estuary in 1994 (Macleod et al., 2016) and has since proliferated along UK coastlines. One year after its discovery at the Queen Anne Battery marina, Plymouth, it became a major fouling plant on pontoons (Minchin & Nunn, 2014). Although initially restricted to artificial habitats, such as marinas and ports, it is now widespread in natural habitats in several areas, including Plymouth Sound. Undaria pinnatifida seems to settle better on artificial substrata (e.g., floats, marinas or piers) than on natural rocky shores among local kelps (Vaz-Pinto et al., 2014). It is found predominantly in low intertidal to shallow subtidal habitats (Epstein et al., 2019b) and is significantly more abundant on artificial substrata compared to natural rocky substrata (Heiser et al., 2014; Epstein & Smale, 2018). James (2017) suggested that Undaria pinnatifida could outcompete native species on artificial substrata (such as marinas and wharf structures). In Plymouth, UK, De Leij et al. (2017) found that natural habitats with dense native macroalgal canopies, such as Laminaria hyperborea, Laminaria ochroleuca, Laminaria digitata and Saccharina latissima had more resistance to Undaria pinnatifida invasion than disturbed or sparse canopies, due to limited space and light availability for Undaria pinnatifida recruits. However, the dense canopies did not always prevent the invasion of Undaria pinnatifida as sporophytes were still recorded within dense Laminaria canopies, so that canopy disturbance was not always required (De Leij et al., 2017; Epstein & Smale, 2018). Undaria behaves as a winter annual, and recruitment occurs in winter followed by rapid growth through spring, maturity and then senescence through summer, with only the microscopic life stages persisting through autumn. It exhibits multiple dispersal strategies, such as short-range spore dispersal, and long-range dispersal as whole drift plants or fragments. Undaria pinnatifida has spread rapidly across the UK and Europe, resulting in community-wide responses and impacts (Vaz-Pinto et al., 2014; Epstein & Smale, 2017). Its impacts are complex and context-specific, depending on space, time, and taxa present in the introduced location (Epstein & Smale, 2017; Teagle et al., 2017; Tidbury, 2020). Undaria pinnatifida has a wide physiological niche meaning it can occur in both coastal and estuarine environments showing tolerance for varying salinities, turbidity and siltation (Heiser et al., 2014; Epstein & Smale, 2018). Undaria pinnatifida has a greater preference for sites sheltered with low wave exposure and weak tidal streams (Heiser et al., 2014; Epstein & Smale, 2018). In natural habitats, Undaria pinnatifida was not recorded if the wave fetch was greater than 642 km but increased in abundance and cover in very sheltered sites (Epstein & Smale, 2018). In St Malo, France, there was evidence that Undaria pinnatifida coexisted with Laminaria hyperborea under certain conditions (Castric-Fey et al., 1993). Epstein & Smale (2018) also observed that Undaria pinnatifida was relatively common (abundance of >70 individuals per 25 m transect) at three sites in Devon, UK (Jennycliff, Bovisand and Beacon Cove) where Laminaria spp. were abundant (40 to 79%) or superabundant (>80%), which suggested that Undaria pinnatifida could coexist within refugia amongst areas with dense Laminaria spp. In Plymouth Sound, UK, Heiser et al. (2014) observed that Laminaria hyperborea was significantly less abundant at sites with the presence of Undaria pinnatifida, with only approx. 0.5 Laminaria hyperborea individuals per m2 present compared to approx. 8 individuals per m2 at sites without the presence of Undaria pinnatifida. However, the results from their correlation study only showed that the species were not found together (pers. comm., Epstein, 2021). Whereas exclusion and succession experiments on reefs tell us that Laminaria spp. exclude Undaria pinnatifida, not the other way around. Epstein & Smale (2018) reported that in Devon, UK, persistent, dense, and intact Laminaria spp. canopies in rocky reef habitats exerted a strong influence over the presence/absence, abundance, and percentage cover of Undaria pinnatifida. A dense canopy of native kelp restricts the proliferation of Undaria pinnatifida and disturbance of the canopy is often the key to the recruitment of Undaria pinnatifida. Epstein et al. (2019b) reported that Undaria pinnatifida density and biomass were significantly negatively correlated with the sum of all Laminaria spp. in Plymouth, UK. The evidence indicated that native Laminaria spp. canopies in the UK inhibited Undaria pinnatifida and that Undaria pinnatifida was opportunistic but competitively inferior (Farrell & Fletcher, 2006; Heiser et al., 2014; Minchin & Nunn, 2014; De Leij et al., 2017; Epstein & Smale, 2018; Epstein et al., 2019b). However, Epstein et al. (2019b) also noted that Laminaria hyperborea had a non-significant positive relationship with Undaria pinnatifida due to low densities of Laminaria hyperborea across the study area, resulting in insufficient data. In Plymouth Sound (UK), Epstein et al. (2019b) found that within its depth range (+1 to –4 m), Undaria pinnatifida coexisted with seven species of canopy-forming brown macroalgae, including Laminaria hyperborea. De Leij et al. (2017) found that natural habitats with dense native macroalgal canopies, such as Laminaria hyperborea had more resistance to Undaria pinnatifida invasion than disturbed or sparse canopies, due to limited space and light availability for Undaria recruits. However, the dense canopies will not prevent the invasion of Undaria, as sporophytes were still recorded within dense Laminaria canopies, and this suggests that canopy disturbance is not always required. Undaria pinnatifida was successfully eradicated on a sunken ship in Chatham Islands, New Zealand, by applying a heat treatment of 70°C (Wotton et al., 2004). However, numerous other eradication attempts have failed and as noted by Fletcher & Farrell (1998), once established Undaria pinnatifida resists most attempts at long-term removal. Sensitivity AssessmentUndaria pinnatifida has the potential to colonize and coexist in refugia within kelp habitats, especially in shallow examples of their biotopes that are within its depth range (1 to 4 m) and sheltered from wave action. A dense kelp canopy may restrict or slow the proliferation of Undaria pinnatifida. A lower abundance of native macroalgae may result in increased Undaria pinnatifida growth. However, it is highly unlikely that Undaria pinnatifida will be able to colonize or survive the degree of wave exposure that characterizes these biotopes. Therefore, sensitivity is assessed as ‘Not Sensitive’. Overall, confidence is assessed as ‘Low’ due to evidence of variation and the site-specific nature of competition between native kelps and Undaria pinnatifida. | HighHelp | HighHelp | Not sensitiveHelp |
Other INIS [Show more]Other INISEvidenceThe golden kelp Laminaria ochroleuca is a warm-temperate Lusitanian kelp with a distribution ranging from Morocco to the south of the UK. It was first recorded in the southwest UK in 1946 (Parke, 1948) and is projected to expand further northwards under future climate change scenarios (Franco et al., 2018). A small population was recorded in northwest Ireland in 2018 (Schoenrock et al., 2019), further suggesting ongoing poleward expansion. While not considered a traditional invasive species, its northward expansion into the UK has led to competition with Laminaria hyperborea. In Plymouth Sound, southwest UK, estimates of Laminaria ochroleuca standing stock are now comparable to those of Laminaria hyperborea (Taylor-Robinson et al., 2024; also see Smale et al., 2016 for standing stock of Laminaria hyperborea). It is suggested that Laminaria ochroleuca may have a competitive advantage over Laminaria hyperborea due to its tolerance of warmer waters. Barrientos et al. (2025) investigated changes in kelp forests in northwest Spain between 1997 and 2023. They found that kelp forests had disappeared or severely declined in density at 29 of 50 sites, and the canopy was now dominated by Laminaria ochroleuca at the surviving sites, while Laminaria hyperborea is almost entirely absent, occurring at only two sites. These changes were linked to sea surface temperature (an average increase of 0.01 to 0.02°C per year over the 26-year study period), which suggested that Laminaria ochroleuca was more resistant to warming and could therefore outcompete Laminaria hyperborea under global warming scenarios. There is contrasting evidence on the relative resilience of Laminaria ochroleuca and Laminaria hyperborea to storm damage. Pereira et al. (2017) reported no recovery of Laminaria hyperborea populations in the two years following a storm in northern Portugal, whereas Laminaria ochroleuca showed partial recovery. In contrast, Smale & Vance (2015) found that Laminaria hyperborea was highly resistant to severe storms in the UK during the 2013 to 2014 winter season. The breakage of mature Laminaria hyperborea stipes ranged between 2.3 and 6.9%, while broken Laminaria ochroleuca stipes were on average 8.7 times more prevalent. Given this conflicting evidence, it remains unclear whether Laminaria ochroleuca biotopes could displace Laminaria hyperborea biotopes following storm events. Another potential advantage of Laminaria ochroleuca is its greater average stipe length compared to Laminaria hyperborea, potentially reducing light availability for Laminaria hyperborea recruits in mixed-population forests (Smale et al., 2015). This shading effect may exaggerate the impacts of marine heatwaves on Laminaria hyperborea, as elevated temperatures increase metabolic demands that cannot be met under light-limited conditions (Bass et al., 2023). The introduction of Laminaria ochroleuca into Laminaria hyperborea forests can have negative impacts on biodiversity. Kelp stipe assemblages differ significantly between the two species due to the texture of the stipe. Laminaria hyperborea stipes are rough and pitted and therefore have a larger surface area, while Laminaria ochroleuca stipes are uniformly smooth. Teagle & Smale (2018) found species from up to 15 different taxonomic groups on Laminaria hyperborea stipes in spring, compared to 2 taxa at most on Laminaria ochroleuca stipes all year round. In addition, the biomass of Laminaria hyperborea stipe assemblages was >3600 more than Laminaria ochroleuca stipe assemblages. Therefore, the proliferation of Laminaria ochroleuca could reduce available habitat space for epibionts that are associated with Laminaria hyperborea biotopes. Sensitivity AssessmentNo evidence was found of Laminaria ochroleuca competing against the macroalgae species that characterise this biotope. KFaR.Ala and its sub-biotopes occur across a range of wave exposure levels, from extremely exposed to moderately exposed. At present, Laminaria ochroleuca is abundant only in KFaR.LhypLoch, which occurs in sheltered to moderately exposed conditions, and is less abundant in KFaR.LhypR.Loch, which occurs in exposed to very exposed conditions (JNCC, 2022). Evidence also suggests that Laminaria ochroleuca is less resistant to wave action than Laminaria hyperborea (see Wave Exposure Changes section in IR.HIR.KFaR.LhypR.Loch). Since Laminaria hyperborea is excluded from KFaR.Ala biotopes by the high wave action of the sublittoral fringe, these conditions are also likely to exclude Laminaria ochroleuca. Resistance is therefore assessed as ‘High’, resilience as ‘High’ by default (no impact to recover from), and sensitivity as ‘Not Sensitive’. | HighHelp | HighHelp | Not sensitiveHelp |
Bibliography
Béchemin, C., Soletchnik, P., Polsenaere, P., Le Moine, O., Pernet, F., Protat, M., Fuhrmann, M., Quere, C., Goulitquer, S. & Corporeau, C., 2014. Surmortalités de la moule bleue Mytilus edulis dans les Pertuis Charentais (mars 2014).
Cheikh, Y.B., Travers, M., Morga, B., Godfrin, Y., Rioult, D. & Le Foll, F., 2016. First evidence for a Vibrio strain pathogenic to Mytilus edulis altering hemocyte immune capacities. Developmental & Comparative Immunology, 57, 107–119.
Knöbel, L., Nascimento-Schulze, J.C., Sanders, T., Zeus, D., Hiebenthal, C., Barboza, F.R., Stuckas, H. & Melzner, F., 2021. Salinity driven selection and local adaptation in Baltic Sea mytilid mussels. Frontiers in Marine Science, 8, 692078.
Liu, Q., Herman, P.M.J., Mooij, W.M., Huisman, J., Scheffer, M., Olff, H. & van de Koppel, J., 2014. Pattern formation at multiple spatial scales drives the resilience of mussel bed ecosystems. Nature Communications, 5 (1), 5234. DOI https://doi.org/10.1038/ncomms6234
Theisen, B.F., 1973. The growth of Mytilus edulis L. (Bivalvia) from Disko and Thule district, Greenland. Ophelia, 12 (1-2), 59–77.
van de Koppel, J., Rietkerk, M., Dankers, N. & Herman, P.M.J., 2005. Scale‐Dependent Feedback and Regular Spatial Patterns in Young Mussel Beds. The American Naturalist, 165 (3), E66–E77. DOI https://doi.org/10.1086/428362
Airoldi, L., 2003. The effects of sedimentation on rocky coast assemblages. Oceanography and Marine Biology: An Annual Review, 41,161-236
Ajithkumar, M., D'Ambrosio, J., Travers, M.A., Morvezen, R. & Degremont, L., 2025. Genomic selection for resistance to one pathogenic strain of Vibrio splendidus in blue mussel Mytilus edulis. Frontiers in Genetics, 15. DOI https://doi.org/10.3389/fgene.2024.1487807
Ajithkumar, M., Lillehammer, M., Travers, M.A., Maurouard, E., Aslam, M.L. & Dégremont, L., 2024. Genetic parameters for resistance to field mortality outbreaks and resistance to a pathogenic strain of Vibrio splendidus in Mytilus edulis, Mytilus galloprovincialis and natural hybrid. Aquaculture, 590. DOI https://doi.org/10.1016/j.aquaculture.2024.741034
Akaishi, F.M., St-Jean, S.D., Bishay, F., Clarke, J., Rabitto, I.d.S. & Ribeiro, C.A., 2007. Immunological responses, histopathological finding and disease resistance of blue mussel (Mytilus edulis) exposed to treated and untreated municipal wastewater. Aquatic Toxicology, 82 (1), 1-14.
Albert, L., Deschamps, F., Jolivet, A., Olivier, F., Chauvaud, L. & Chauvaud, S., 2020. A current synthesis on the effects of electric and magnetic fields emitted by submarine power cables on invertebrates. Marine Environmental Research, 159. DOI https://doi.org/10.1016/j.marenvres.2020.104958
Albert, L., Maire, O., Olivier, F., Lambert, C., Romero-Ramirez, A., Jolivet, A., Chauvaud, L. & Chauvaud, S., 2022. Can artificial magnetic fields alter the functional role of the blue mussel, Mytilus edulis?. Marine Biology, 169 (6). DOI https://doi.org/10.1007/s00227-022-04065-4
Alfaro, A.C., 2005. Effect of water flow and oxygen concentration on early settlement of the New Zealand green-lipped mussel, Perna canaliculus. Aquaculture, 246, 285-94.
Alfaro, A.C., 2006. Byssal attachment of juvenile mussels, Perna canaliculus, affected by water motion and air bubbles. Aquaculture, 255, 357-61
Almada-Villela P.C., 1984. The effects of reduced salinity on the shell growth of small Mytilus edulis L. Journal of the Marine Biological Association of the United Kingdom, 64, 171-182.
Almada-Villela, P.C., Davenport, J. & Gruffydd, L.L.D., 1982. The effects of temperature on the shell growth of young Mytilus edulis L. Journal of Experimental Marine Biology and Ecology, 59, 275-288.
Alves, M. T. & Tidbury, H. J., 2022. Invasive non-native species management under climatic and anthropogenic pressure: application of a modelling framework. Management of Biological Invasions, 13 (2), 259-273. DOI https://doi.org/10.3391/mbi.2022.13.2.01
Alves, M. T., Taylor, N. G. H. & Tidbury, H. J., 2021. Understanding drivers of wild oyster population persistence. Sci Rep, 11 (1), 7837. DOI https://doi.org/10.1038/s41598-021-87418-1
Ameyaw-Akumfi, C. & Naylor, E., 1987. Spontaneous and induced components of salinity preference behaviour in Carcinus maenas. Marine Ecology Progress Series, 37, 153-158.
Andersen, G.S., Steen, H., Christie, H., Fredriksen, S. & Moy, F.E., 2011. Seasonal patterns of sporophyte growth, fertility, fouling, and mortality of Saccharina latissima in Skagerrak, Norway: implications for forest recovery. Journal of Marine Biology, 2011, Article ID 690375, 8 pages. DOI: https://doi.org/10.1155/2011/690375
Andrew, N.L. & Viejo, R.M., 1998. Ecological limits to the invasion of Sargassum muticum in northern Spain. Aquatic Botany, 60 (3), 251-263. DOI https://doi.org/10.1016/S0304-3770(97)00088-0
Arafeh-Dalmau, N., Montaño-Moctezuma, G., Martínez, J.A., Beas-Luna, R., Schoeman, D.S. & Torres-Moye, G., 2019. Extreme Marine Heatwaves Alter Kelp Forest Community Near Its Equatorward Distribution Limit. Frontiers in Marine Science, 6 (499). DOI https://doi.org/10.3389/fmars.2019.00499
Arnold, M., Teagle, H., Brown, M.P. & Smale, D.A., 2016. The structure of biogenic habitat and epibiotic assemblages associated with the global invasive kelp Undaria pinnatifida in comparison to native macroalgae. Biological Invasions, 18 (3), 661-676. DOI https://doi.org/10.1007/s10530-015-1037-6
Arzel, P., 2002. La laminaire digitée. Les nouvelles de l’Ifremer, 33 (4).
Arzel, P., 1998. Les laminaires sur les côtes bretonnes. Évolution de l'exploitation et de la flottille de pêche, état actuel et perspectives. Plouzané, France: Ifremer.
Assis, J., Lucas, A.V., Bárbara, I. & Serrão, E.Á., 2016. Future climate change is predicted to shift long-term persistence zones in the cold-temperate kelp Laminaria hyperborea. Marine Environmental Research, 113, 174-182. DOI https://doi.org/10.1016/j.marenvres.2015.11.005
Assis, J., Serrão, E.A., Claro, B., Perrin, C. & Pearson, G.A., 2014. Climate-driven range shifts explain the distribution of extant gene pools and predict future loss of unique lineages in a marine brown alga. Molecular Ecology, 23 (11), 2797-2810. DOI https://doi.org/10.1111/mec.12772
Aunaas, T., Denstad, J-P. & Zachariassen, K., 1988. Ecophysiological importance of the isolation response of hibernating blue mussels (Mytilus edulis). Marine Biology 98: 415-9
Bøgwald, M., Skår, C.K., Karlsbakk, E., Alfjorden, A., Feist, S.W., Bass, D. & Mortensen, S., 2022. Infection cycle of Marteilia pararefringens in blue mussels Mytilus edulis in a heliothermic marine oyster lagoon in Norway. Diseases of Aquatic Organisms, 148, 153–166. DOI https://doi.org/10.3354/dao03651
Baardseth, E., 1956. The growth rings in Alaria stipes. In Proceedings of the International Seaweed Symposium, 2, Trondheim (eds T. Braarud & N.A. Sorensen) pp. 153-157. London: Pergamon Press.
Bahmet, I., Berger, V. & Halaman, V., 2005. Heart rate in the blue mussel Mytilus edulis (Bivalvia) under salinity change. Russian Journal of Marine Biology, 31, 314-7
Baird, R.H., 1966. Factors affecting the growth and condition of mussels (Mytilus edulis). Fishery Investigations. Ministry of Agriculture, Fisheries and Food, Series II, no. 25, 1-33.
Bakhmet, I., Aristov, D., Marchenko, J. & Nikolaev, K., 2022. Handling the heat: Changes in the heart rate of two congeneric blue mussel species and their hybrids in response to water temperature. Journal of Sea Research, 185. DOI https://doi.org/10.1016/j.seares.2022.102218
Bakhmet, I.N., 2017. Cardiac activity and oxygen consumption of blue mussels (Mytilus edulis) from the White Sea in relation to body mass, ambient temperature and food availability. Polar Biology, 40 (10), 1959–1964. DOI https://doi.org/10.1007/s00300-017-2111-6
Balseiro P., Montes A., Ceschia G., Gestal C., Novoa B. & Figueras A., 2007. Molecular epizootiology of the European Marteilia spp., infecting mussels (Mytilus galloprovincialis and M. edulis) and oysters (Ostrea edulis): an update. Bulletin of the European Association of Fish Pathologists, 27(4), 148-156.
Bamber, R.N. & Irving, P.W., 1993. The Corallina run-offs of Bridgewater Bay. Porcupine Newsletter, 5, 190-197.
Bamber, S.D., 2018. Does sustained tolerance of reduced salinity seawater alter phagocytosis efficiency in haemocytes of the blue mussel Mytilus edulis (L.)?. Journal of Experimental Marine Biology and Ecology, 500, 132–139. DOI https://doi.org/10.1016/j.jembe.2017.07.006
Banke, T.L., Steinfurth, R.C., Lange, T., Canal-Vergés, P., Svane, N. & Flindt, M.R., 2024. Dislodgement and mortality challenges when restoring shallow mussel beds (Mytilus edulis) in a Danish estuary. Restoration Ecology, 32 (5). DOI https://doi.org/10.1111/rec.14160
Barrett, N.J., Thyrring, J., Harper, E.M., Sejr, M.K., Sorensen, J.G., Peck, L.S. & Clark, M.S., 2022. Molecular responses to thermal and osmotic stress in arctic intertidal mussels (Mytilus edulis): the limits of resilience. Genes, 13 (1). DOI https://doi.org/10.3390/genes13010155
Barrientos, S., Piñeiro-Corbeira, C. & Barreiro, R., 2025. Twenty-five years on: Widespread kelp forest decline revealed in a potential climatic refugium. Journal of Environmental Management, 373. DOI https://doi.org/10.1016/j.jenvman.2024.123734
Bartsch, I., Vogt, J., Pehlke, C. & Hanelt, D., 2013. Prevailing sea surface temperatures inhibit summer reproduction of the kelp Laminaria digitata at Helgoland (North Sea). Journal of Phycology, 49 (6), 1061-1073.
Bartsch, I., Wiencke, C., Bischof, K., Buchholz, C.M., Buck, B.H., Eggert, A., Feuerpfeil, P., Hanelt, D., Jacobsen, S. & Karez, R., 2008. The genus Laminaria sensu lato: recent insights and developments. European Journal of Phycology, 43 (1), 1-86.
Bass, A.V., Smith, K.E. & Smale, D.A., 2023. Marine heatwaves and decreased light availability interact to erode the ecophysiological performance of habitat-forming kelp species. Journal of Phycology, 59 (3), 481–495. DOI https://doi.org/10.1111/jpy.13332
Bayne B., 1964. Primary and secondary settlement in Mytilus edulis L.(Mollusca). Journal of Animal Ecology, 33, 513-523.
Bayne, B., Iglesias, J., Hawkins, A., Navarro, E., Heral, M., Deslous-Paoli, J-M., 1993. Feeding behaviour of the mussel, Mytilus edulis: responses to variations in quantity and organic content of the seston. Journal of the Marine Biological Association of the United Kingdom, 73, 813-29
Bayne, B.L. (ed.), 1976b. Marine mussels: their ecology and physiology. Cambridge: Cambridge University Press. [International Biological Programme 10.]
Bayne, B.L., 1976a. The biology of mussel larvae. In Marine mussels: their ecology and physiology (ed. B.L. Bayne), pp. 81-120. Cambridge: Cambridge University Press. [International Biological Programme 10.]
Bearham, D., Vanderklift, M.A., Downie, R.A., Thomson, D.P. & Clementson, L.A., 2020. Macrophyte-derived detritus in shallow coastal waters contributes to suspended particulate organic matter and increases growth rates of Mytilus edulis. Marine Ecology Progress Series, 644, 91–103. DOI https://doi.org/10.3354/meps13314
Beauchamp, K.A., Gowing, M.M., 1982. A quantitative assessment of human trampling effects on a rocky intertidal community. Marine Environmental Research, 7, 279-94
Beesley, A., Lowe, D.M., Pascoe, C.K. & Widdicombe, S., 2008. Effects of CO2-induced seawater acidification on the health of Mytilus edulis. Climate Research, 37 (2-3), 215-225. DOI https://doi.org/10.3354/cr00765
Bégin, C., Johnson, L.E. & Himmelman, J.H., 2004. Macroalgal canopies: distribution and diversity of associated invertebrates and effects on the recruitment and growth of mussels. Marine Ecology Progress Series, 271 (1), 121-132.
Cheikh, Y.B. & Travers, M.A., 2022. Vibrio splendidus infection induces dysbiosis in the blue mussel and favors pathobiontic bacteria. Microbiological Research, 261. DOI https://doi.org/10.1016/j.micres.2022.127078
Benabdelmouna, A. & Ledu, C., 2016. The mass mortality of blue mussels (Mytilus spp.) from the Atlantic coast of France is associated with heavy genomic abnormalities as evidenced by flow cytometry. Journal of Invertebrate Pathology, 138, 30–38. DOI https://doi.org/10.1016/j.jip.2016.06.001
Berge, J., Johnsen, G., Nilsen, F., Gulliksen, B. & Slagstad, D., 2005. Ocean temperature oscillations enable reappearance of blue mussels Mytilus edulis in Svalbard after a 1000 year absence. Marine Ecology Progress Series, 303, 167-175.
Berge, J.A., Bjerkeng, B., Pettersen, O., Schaanning, M.T. & Øxnevad, S., 2006. Effects of increased sea water concentrations of CO2 on growth of the bivalve Mytilus edulis L. Chemosphere, 62 (4), 681-687. DOI https://doi.org/10.1016/j.chemosphere.2005.04.111
Bergmann, M., Wieczorek, S.K., Moore, P.G., 2002. Utilisation of invertebrates discarded from the Nephrops fishery by variously selective benthic scavengers in the west of Scotland. Marine Ecology Progress Series, 233,185-98
Bergström, P., Thorngren, L., Strand, Å & Lindegarth, M., 2021. Identifying high-density areas of oysters using species distribution modeling: Lessons for conservation of the native Ostrea edulis and management of the invasive Magallana (Crassostrea) gigas in Sweden. Ecology and Evolution, 11 (10), 5522-5532. DOI https://doi.org/10.1002/ece3.7451
Berthe, F.C.J., Le Roux, F., Adlard, R.D. & Figueras, A., 2004. Marteiliosis in molluscs: a review. Aquatic Living Resources, 17 (4), 433-448.
Beszczynska-Möller, A., & Dye, S.R., 2013. ICES Report on Ocean Climate 2012. In ICES Cooperative Research Report, vol. 321 pp. 73.
Beukema, J. J., Dekker, R., Drent, J. & van der Meer, J., 2017a. Long-term changes in annual growth of bivalves in the Wadden Sea: influences of temperature, food, and abundance. Marine Ecology Progress Series, 573, 143–156. DOI https://doi.org/10.3354/meps12122
Bigot-Clivot, A., La Carbona, S., Cazeaux, C., Durand, L., Géba, E., Le Foll, F., Xuereb, B., Chalghmi, H., Dubey, J.P., Bastien, F., Bonnard, I., Ladeiro, M.P., Escotte-Binet, S., Aubert, D., Villena, I. & Geffard, A., 2022. Blue mussel (Mytilus edulis)-A bioindicator of marine water contamination by protozoa: Laboratory and in situ approaches. Journal of Applied Microbiology, 132 (1), 736–746. DOI https://doi.org/10.1111/jam.15185
Binzer, S.B., Lundgreen, R.B.C., Berge, T., Hansen, P.J. & Vismann, B., 2018. The blue mussel Mytilus edulis is vulnerable to the toxic dinoflagellate Karlodinium armiger - Adult filtration is inhibited and several life stages killed. Plos One, 13 (6). DOI https://doi.org/10.1371/journal.pone.0199306
Birchenough, S., Bremner, J., Henderson, P., Hinz, H., D, S., Mieszkowska, N., Roberts, J., Kamenos, N. & Plenty, S., 2013. Impacts of climate change on shallow and shelf subtidal habitats. Marine Climate Change Impacts Partnership: Science Review, 2013. DOI http://doi.org/10.14465/2013.arc20.193-203
Birkett, D.A., Maggs, C.A., Dring, M.J. & Boaden, P.J.S., 1998b. Infralittoral reef biotopes with kelp species: an overview of dynamic and sensitivity characteristics for conservation management of marine SACs. Natura 2000 report prepared by Scottish Association of Marine Science (SAMS) for the UK Marine SACs Project., Scottish Association for Marine Science. (UK Marine SACs Project, vol VI.), 174 pp. Available from: http://ukmpa.marinebiodiversity.org/uk_sacs/pdfs/reefkelp.pdf
Bishop, J. D. D., Wood, C. A., Yunnie, A. L. E. & Griffiths, C. A., 2015. Unheralded arrivals: non-native sessile invertebrates in marinas on the English coast. Aquatic Invasions, 10 (3), 249-264. DOI https://doi.org/10.3391/ai.2015.10.3.01
Blanchard, M., 2009. Recent expansion of the slipper limpet population (Crepidula fornicata) in the Bay of Mont-Saint-Michel (Western Channel, France). Aquatic Living Resources, 22 (1), 11-19. DOI https://doi.org/10.1051/alr/2009004
Blanchard, M., 1997. Spread of the slipper limpet Crepidula fornicata (L.1758) in Europe. Current state and consequences. Scientia Marina, 61, Supplement 9, 109-118. Available from: http://scimar.icm.csic.es/scimar/index.php/secId/6/IdArt/290/
Bohn, K., Richardson, C. & Jenkins, S., 2012. The invasive gastropod Crepidula fornicata: reproduction and recruitment in the intertidal at its northernmost range in Wales, UK, and implications for its secondary spread. Marine Biology, 159 (9), 2091-2103. DOI https://doi.org/10.1007/s00227-012-1997-3
Bohn, K., Richardson, C.A. & Jenkins, S.R., 2015. The distribution of the invasive non-native gastropod Crepidula fornicata in the Milford Haven Waterway, its northernmost population along the west coast of Britain. Helgoland Marine Research, 69 (4), 313.
Bohn, K., Richardson, C.A. & Jenkins, S.R., 2013a. Larval microhabitat associations of the non-native gastropod Crepidula fornicata and effects on recruitment success in the intertidal zone. Journal of Experimental Marine Biology and Ecology, 448, 289-297. DOI https://doi.org/10.1016/j.jembe.2013.07.020
Bohn, K., Richardson, C.A. & Jenkins, S.R., 2013b. The importance of larval supply, larval habitat selection and post-settlement mortality in determining intertidal adult abundance of the invasive gastropod Crepidula fornicata. Journal of Experimental Marine Biology and Ecology, 440, 132-140. DOI https://doi.org/10.1016/j.jembe.2012.12.008
Both, A., Byron, C.J., Costa-Pierce, B., Parrish, C.C. & Brady, D.C., 2020. Detrital subsidies in the diet of Mytilus edulis; macroalgal detritus likely supplements essential fatty acids. Frontiers in Marine Science, 7. DOI https://doi.org/10.3389/fmars.2020.561073
Boukadida, K., Mlouka, R., Clerandeau, C., Banni, M. & Cachot, J., 2021. Natural distribution of pure and hybrid Mytilus sp. along the south Mediterranean and North-east Atlantic coasts and sensitivity of D-larvae stages to temperature increases and metal pollution. Science of the Total Environment, 756. DOI https://doi.org/10.1016/j.scitotenv.2020.143675
Bouras, H., Quesnelle, Y., Barozet, A., Goux, D., Blin, J.L., Savary, M., Zatylny-Gaudin, C. & Houssin, M., 2023. First isolation of Francisella halioticida strains from blue mussel (Mytilus edulis) in Normandy, France. Journal of Invertebrate Pathology, 200. DOI https://doi.org/10.1016/j.jip.2023.107950
Bower, S.M., 1996. Synopsis of Infectious Diseases and Parasites of Commercially Exploited Shellfish: Bald-sea-urchin Disease. [On-line]. Fisheries and Oceans Canada. [cited 26/01/16]. Available from:
Bower S.M., 2010. Synopsis of Infectious Diseases and Parasites of Commercially Exploited Shellfish [online]. Ontario, Fisheries and Oceans, Canada. Available from: http://dev-public.rhq.pac.dfo-mpo.gc.ca/science/species-especes/shellfish-coquillages/diseases-maladies/index-eng.htm [Accessed: 14/02/2014]
Bower, S.M., 1992. Diseases and parasites of mussels. In The mussel Mytilus: ecology, physiology, genetics and culture (ed. E.M. Gosling), pp. 543-563. Amsterdam: Elsevier Science Publ. [Developments in Aquaculture and Fisheries Science, no. 25.]
Breeman, A.M., 1990. Expected Effects of Changing Seawater Temperatures on the Geographic Distribution of Seaweed Species. In Beukema, J.J., et al. (eds.). Expected Effects of Climatic Change on Marine Coastal Ecosystems, Dordrecht: Springer Netherlands, pp. 69-76. DOI: https://doi.org/10.1007/978-94-009-2003-3_9
Britton, D., Cornwall, C.E., Revill, A.T., Hurd, C.L. & Johnson, C.R., 2016. Ocean acidification reverses the positive effects of seawater pH fluctuations on growth and photosynthesis of the habitat-forming kelp, Ecklonia radiata. Scientific reports, 6 (1), 26036. DOI: https://doi.org/10.1038/srep26036
Britton-Simmons, K.H., 2004. Direct and indirect effects of the introduced alga Sargassum muticum on benthic, subtidal communities of Washington State, USA. Marine Ecology Progress Series, 277, 61-78. DOI https://doi.org/10.3354/meps277061
Brodie J., Williamson, C.J., Smale, D.A., Kamenos, N.A., Mieszkowska, N., Santos, R., Cunliffe, M., Steinke, M., Yesson, C. & Anderson, K.M., 2014. The future of the northeast Atlantic benthic flora in a high CO2 world. Ecology and Evolution, 4 (13), 2787-2798. DOI https://doi.org/10.1002/ece3.1105
Brosnan, D.M. & Crumrine, L.L., 1994. Effects of human trampling on marine rocky shore communities. Journal of Experimental Marine Biology and Ecology, 177, 79-97.
Broughton, C.C., Bailey, J., Green, D., Weidmann, M. & Carboni, D., 2019. Spat mortality in farmed blue mussels (Mytilus edulis) in Scotland. Insitute of Aquaculture. University of Stirling.
Brown, P.J. & Taylor, R.B., 1999. Effects of trampling by humans on animals inhabiting coralline algal turf in the rocky intertidal. Journal of Experimental Marine Biology and Ecology, 235, 45-53.
Bryan, G.W., 1984. Pollution due to heavy metals and their compounds. In Marine Ecology: A Comprehensive, Integrated Treatise on Life in the Oceans and Coastal Waters, vol. 5. Ocean Management, part 3, (ed. O. Kinne), pp.1289-1431. New York: John Wiley & Sons.
Bullard, S. G. & Whitlatch, R. B., 2009. In situ growth of the colonial ascidian Didemnum vexillum under different environmental conditions. Aquatic Invasions, 4, 275-278. DOI https://doi.org/10.3391/ai.2009.4.1.27
Bullard, S. G., Lambert, G., Carman, M. R., Byrnes, J., Whitlatch, R. B., Ruiz, G., Miller, R. J., Harris, L., Valentine, P. C., Collie, J. S., Pederson, J., McNaught, D. C., Cohen, A. N., Asch, R. G., Dijkstra, J. & Heinonen, K., 2007. The colonial ascidian Didemnum sp. A: Current distribution, basic biology and potential threat to marine communities of the northeast and west coasts of North America. Journal of Experimental Marine Biology and Ecology, 342 (1), 99-108. DOI https://doi.org/10.1016/j.jembe.2006.10.020
Bultelle, F., Boutet, I., Devin, S., Caza, F., St-Pierre, Y., Péden, R., Brousseau, P., Chan, P., Vaudry, D., Le Foll, F., Fournier, M., Auffret, M. & Rocher, B., 2021. Molecular response of a sub-antarctic population of the blue mussel (Mytilus edulis platensis) to a moderate thermal stress. Marine Environmental Research, 169. DOI https://doi.org/10.1016/j.marenvres.2021.105393
Burrows, M.T., 2017. Intertidal species and habitats. MCCIP Science Review 2017, 62-72. DOI https://doi.org/10.14465/2017.arc10.006-ish
- Burrows, M.T., Hawkins, S. J., Moore, J. J., Adams, L., Sugden, H., Firth, L. B. & Mieszkowska, N., 2020. Global‐scale species distributions predict temperature‐related changes in species composition of rocky shore communities in Britain. Global Change Biology, 26 (4), 2093–2105. DOI https://doi.org/10.1111/gcb.14968
Burrows, M.T., Smale, D., O’Connor, N., Rein, H.V. & Moore, P., 2014. Marine Strategy Framework Directive Indicators for UK Kelp Habitats Part 1: Developing proposals for potential indicators. Joint Nature Conservation Comittee, Peterborough. Report no. 525.
Buschbaum, C. & Saier, B., 2001. Growth of the mussel Mytilus edulis L. in the Wadden Sea affected by tidal emergence and barnacle epibionts. Journal of Sea Research, 45, 27-36
Bussell, J. A., Gidman, E. A., Causton, D. R., Gwynn-Jones, D., Malham, S. K., Jones, M. L. M., Reynolds, B. & Seed. R., 2008. Changes in the immune response and metabolic fingerprint of the mussel, Mytilus edulis (Linnaeus) in response to lowered salinity and physical stress. Journal of Experimental Marine Biology and Ecology, 358, 78-85.
Cárdenas, L., Leclerc, J.C., Bruning, P., Garrido, I., Détrée, C., Figueroa, A., Astorga, M., Navarro, J.M., Johnson, L.E., Carlton, J.T. & Pardo, L., 2020. First mussel settlement observed in Antarctica reveals the potential for future invasions. Scientific Reports, 10 (1). DOI https://doi.org/10.1038/s41598-020-62340-0
Cabral, S., Carvalho, F., Gaspar, M., Ramajal, J., Sá, E., Santos, C., Silva, G., Sousa, A., Costa, J. L. & Chainho, P., 2020. Non-indigenous species in soft-sediments: Are some estuaries more invaded than others?. Ecological Indicators, 110. DOI https://doi.org/10.1016/j.ecolind.2019.105640
Cano, I., Parker, A., Ward, G.M., Green, M., Ross, S., Bignell, J., Daumich, C., Kerr, R., Feist, S.W. & Batista, F.M., 2022. First detection of Francisella halioticida infecting a wild population of blue mussels Mytilus edulis in the United Kingdom. Pathogens, 11 (3). DOI https://doi.org/10.3390/pathogens11030329
Capelle, J.J., van Stralen, M.R., Wijsman, J.W.M., Herman, P.M.J. & Smaal, A.C., 2017. Population dynamics of subtidal blue mussels Mytilus edulis and the impact of cultivation. Aquaculture Environment Interactions, 9, 155–168. DOI https://doi.org/10.3354/aei00221
Carman, M.R. & Grunden, D.W., 2010. First occurrence of the invasive tunicate Didemnum vexillum in eelgrass habitat. Aquatic Invasions, 5 (1), 23-29. DOI https://doi.org/10.3391/ai.2010.5.1.4
Carrasco, Mauro F. & Barón, Pedro J., 2010. Analysis of the potential geographic range of the Pacific oyster Crassostrea gigas (Thunberg, 1793) based on surface seawater temperature satellite data and climate charts: the coast of South America as a study case. Biological Invasions, 12 (8), 2597-2607. DOI https://doi.org/10.1007/s10530-009-9668-0
Carrier-Belleau, C., Lauzon, F., Boucher-Fontaine, J., Tiegs, S., Cusson, M., Guichard, F., Nozais, C. & Archambault, P., 2024. Interacting effects of local and global stressors on mussel beds and ecosystem functioning. Journal of Experimental Marine Biology and Ecology, 579. DOI https://doi.org/10.1016/j.jembe.2024.152046
Casas, G., Scrosati, R. & Piriz, M.L., 2004. The invasive kelp Undaria pinnatifida (Phaeophyceae, Laminariales) reduces native seaweed diversity in Nuevo Gulf (Patagonia, Argentina). Biological Invasions, 6 (4), 411-416.
Castric-Fey, A., Girard, A. & L'Hardy-Halos, M.T., 1993. The Distribution of Undaria pinnatifida (Phaeophyceae, Laminariales) on the Coast of St. Malo (Brittany, France). Botanica Marina, 36 (4), 351-358. DOI https://doi.org/10.1515/botm.1993.36.4.351
Cazenave, A. & Nerem, R.S., 2004. Present-day sea-level change: Observations and causes. Reviews of Geophysics, 42 (3). DOI https://doi.org/10.1029/2003rg000139
Cereja, R., Pereira, A., Brito, A. C., Pires, C., Diniz, M., Ferreira, I., Mil-Homens, M., Brito, P., Costa, P. R. & Marques, A., 2026. Laminaria ochroleuca as a natural remediator of copper-based antifouling agents in aquaculture systems. Marine Pollution Bulletin, 223, 119023. DOI https://doi.org/10.1016/j.marpolbul.2025.119023
Chapman, A.R.O., 1981. Stability of sea urchin dominated barren grounds following destructive grazing of kelp in St. Margaret's Bay, Eastern Canada. Marine Biology, 62, 307-311.
Chapple, J.P., Smerdon, G.R., Berry, R.J. & Hawkins, A.J.S., 1998. Seasonal changes in stress-70 protein levels reflect thermal tolerance in the marine bivalve Mytilus edulis L. Journal of Experimental Marine Biology and Ecology, 229 (1), 53-68. DOI https://doi.org/10.1016/S0022-0981(98)00040-9
Chapuis, A.F., Wale, M.A., Bailey, M., Farley, H.M., Bean, T.P. & Regan, T., 2025. Anthropogenic noise exposure suppresses the immune response in Mytilus spp. following Vibrio splendidus challenge. Frontiers in Immunology, 16. DOI https://doi.org/10.3389/fimmu.2025.1657667
Charles, M., Trancart, S., Oden, E. & Houssin, M., 2020. Experimental infection of Mytilus edulis by two Vibrio splendidus-related strains: Determination of pathogenicity level of strains and influence of the origin and annual cycle of mussels on their sensitivity. Journal of Fish Diseases, 43 (1), 9–21. DOI https://doi.org/10.1111/jfd.13094
Christie, H., Fredriksen, S. & Rinde, E., 1998. Regrowth of kelp and colonization of epiphyte and fauna community after kelp trawling at the coast of Norway. Hydrobiologia, 375/376, 49-58.
Christoforou, E., Dominoni, D., Lindström, J., Diamantopoulou, C., Czyzewski, J., Mirzai, N. & Spatharis, S., 2023. The effects of artificial light at night (ALAN) on the gaping activity and feeding of mussels. Marine Pollution Bulletin, 192. DOI https://doi.org/10.1016/j.marpolbul.2023.115105
Chu, F. E., Volety, A. K. & Constantin, G., 1996. A comparison of Crassostrea gigas and Crassostrea virginica: effects of temperature asalinity on susceptibility to the protozoan parasite, Perkinsus marinus. Journal of Shellfish Research, 15 (2), 375–380.
Church, J.A. & White, N.J., 2006. A 20th century acceleration in global sea-level rise. Geophysical Research Letters, 33 (1). DOI https://doi.org/10.1029/2005gl024826
Church, J.A., White, N.J., Coleman, R., Lambeck, K. & Mitrovica, J.X., 2004. Estimates of the Regional Distribution of Sea Level Rise over the 1950–2000 Period. Journal of Climate, 17 (13), 2609-2625.
Cinar, M. E. & Ozgul, A., 2023. Clogging nets Didemnum vexillum (Tunicata: Ascidiacea) is in action in the eastern Mediterranean. Journal of the Marine Biological Association of the United Kingdom, 103. DOI https://doi.org/10.1017/s0025315423000802
Clark, M.S., Peck, L.S. & Thyrring, J., 2021. Resilience in Greenland intertidal Mytilus: The hidden stress defense. Science of the Total Environment, 767. DOI https://doi.org/10.1016/j.scitotenv.2020.144366
Cobos, P., Gordillo, F. J. L., Steiner, N., Bartsch, I. & Iñiguez, C., 2026. Photosynthesis and growth reactivation of kelps after the Polar Night in a warming Arctic. Environmental and Experimental Botany, 248, 106392. DOI https://doi.org/10.1016/j.envexpbot.2026.106392
Cole, S., Codling, I.D., Parr, W. & Zabel, T., 1999. Guidelines for managing water quality impacts within UK European Marine sites. Natura 2000 report prepared for the UK Marine SACs Project. 441 pp., Swindon: Water Research Council on behalf of EN, SNH, CCW, JNCC, SAMS and EHS. [UK Marine SACs Project.]. Available from: http://ukmpa.marinebiodiversity.org/uk_sacs/pdfs/water_quality.pdf
Colthart, B.J., & Johanssen, H.W., 1973. Growth rates of Corallina officinalis (Rhodophyta) at different temperatures. Marine Biology, 18, 46-49.
Connor, D.W., Allen, J.H., Golding, N., Howell, K.L., Lieberknecht, L.M., Northen, K.O. & Reker, J.B., 2004. The Marine Habitat Classification for Britain and Ireland. Version 04.05. ISBN 1 861 07561 8. In JNCC (2015), The Marine Habitat Classification for Britain and Ireland Version 15.03. [2019-07-24]. Joint Nature Conservation Committee, Peterborough. Available from https://mhc.jncc.gov.uk/
Connor, D.W., Dalkin, M.J., Hill, T.O., Holt, R.H.F. & Sanderson, W.G., 1997a. Marine biotope classification for Britain and Ireland. Vol. 2. Sublittoral biotopes. Joint Nature Conservation Committee, Peterborough, JNCC Report no. 230, Version 97.06., Joint Nature Conservation Committee, Peterborough, JNCC Report no. 230, Version 97.06.
Cook, E., Beveridge, C., Lamont, P., O'Higgins, T. & Wilding, T., 2014. Survey of wild Pacific Oyster (Crassostrea gigas) in Scotland. Scottish Aquaculture Research Forum. DOI https://doi.org/10.13140/RG.2.1.1371.7369
Cosse, A., Potin, P. & Leblanc, C., 2009. Patterns of gene expression induced by oligoguluronates reveal conserved and environment‐specific molecular defence responses in the brown alga Laminaria digitata. New Phytologist, 182 (1), 239-250.
Cottrell, R.S., Black, K.D., Hutchison, Z.L. & Last, K.S., 2016. The influence of organic material and temperature on the burial tolerance of the blue mussel, Mytilus edulis: Considerations for the management of marine aggregate dredging. Plos One, 11 (1). DOI https://doi.org/10.1371/journal.pone.0147534
Coutts, A.D.M. & Forrest, B.M., 2007. Development and application of tools for incursion response: Lessons learned from the management of the fouling pest Didemnum vexillum. Journal of Experimental Marine Biology and Ecology, 342 (1), 154-162. DOI https://doi.org/10.1016/j.jembe.2006.10.042
Crisp, D.J. & Mwaiseje, B., 1989. Diversity in intertidal communities with special reference to the Corallina officinalis community. Scientia Marina, 53, 365-372.
Crisp, D.J. (ed.), 1964. The effects of the severe winter of 1962-63 on marine life in Britain. Journal of Animal Ecology, 33, 165-210.
Crump, R.G., Morley, H.S., & Williams, A.D., 1999. West Angle Bay, a case study. Littoral monitoring of permanent quadrats before and after the Sea Empress oil spill. Field Studies, 9, 497-511.
Culloty, S.C., Novoa, B., Pernas, M., Longshaw, M., Mulcahy, M.F., Feist, S.W. & Figueras, A., 1999. Susceptibility of a number of bivalve species to the protozoan parasite Bonamia ostreae and their ability to act as vectors for this parasite. Diseases of Aquatic Organisms, 37 (1), 73-80.
Da Silva Junior, E. C., Babaahmadifooladi, M., Folens, K., dos Reis, A. R., Guilherme, L. R. G., Van de Wiele, T., Jacxsens, L. & Du Laing, G., 2023. Content, speciation and in vitro bioaccessibility of trace elements in seaweeds and derived food products. Journal of Food Composition and Analysis, 118, 105162. DOI https://doi.org/10.1016/j.jfca.2023.105162
Daly, M.A. & Mathieson, A.C., 1977. The effects of sand movement on intertidal seaweeds and selected invertebrates at Bound Rock, New Hampshire, USA. Marine Biology, 43, 45-55.
Dare, P.J., 1976. Settlement, growth and production of the mussel, Mytilus edulis L., in Morecambe Bay, England. Fishery Investigations, Ministry of Agriculture, Fisheries and Food, Series II, 28 , 25pp.
Dauvin, J.C., Bellan, G., Bellan-Santini, D., Castric, A., Francour, P., Gentil, F., Girard, A., Gofas, S., Mahe, C., Noel, P., & Reviers, B. de., 1994. Typologie des ZNIEFF-Mer. Liste des parametres et des biocoenoses des cotes francaises metropolitaines. 2nd ed. Secretariat Faune-Flore, Museum National d'Histoire Naturelle, Paris (Collection Patrimoines Naturels, Serie Patrimoine Ecologique, No. 12). Coll. Patrimoines Naturels, vol. 12, Secretariat Faune-Flore, Paris.
Davenport, J., 1979. The isolation response of mussels (Mytilus edulis) exposed to falling sea water concentrations. Journal of the Marine Biological Association of the United Kingdom, 59, 124-132.
Davies, C.E. & Moss, D., 1998. European Union Nature Information System (EUNIS) Habitat Classification. Report to European Topic Centre on Nature Conservation from the Institute of Terrestrial Ecology, Monks Wood, Cambridgeshire. [Final draft with further revisions to marine habitats.], Brussels: European Environment Agency.
Davies, T.W., McKee, D., Fishwick, J., Tidau, S. & Smyth, T., 2020. Biologically important artificial light at night on the seafloor. Scientific Reports, 10 (1). DOI https://doi.org/10.1038/s41598-020-69461-6
Davoult, E., Engel, C.R., Arzel, P., Knoch, D. & Laurans, M., 2011. Environmental factors and commercial harvesting: exploring possible links behind the decline of the kelp Laminaria digitata in Brittany, France. Cah. Biol. Mar, 52, 1-6.
Dayton, P.K., Tegner, M.J., Parnell, P.E. & Edwards, P.B., 1992. Temporal and spatial patterns of disturbance and recovery in a kelp forest community. Ecological Monographs, 62, 421-445.
De Bettignies, T., De Bettignies, F., Bartsch, I., Bekkby, T., Boiffin, A., Casado de Amezúa, P., Christie, H., Edwards, H., Fournier, N., García, A., Gauthier, L., Gillham, K., Halling, C., Harrald, M., Hennicke, J., Hernández, S., Kilnäs, M., Martinez, B., Mieszkowska, N., Moore, P., Moy, F., Mueller, M., Norderhaug, K.M., Ó Cadhla, O., Parry, M., Ramsay, K., Robertson, M., Russel, T., Serrão, E., Smale, D., Sousa Pinto, I., Steen, H., Street, M., Walday, M., Werner, T. & La Rivière, M., 2021. Background Document for Kelp Forests. OSPAR Commission, London, OSPAR 788/2021, 66 pp. Available from: https://www.ospar.org/documents?v=46796
De Leij, R., Epstein, G., Brown, M.P. & Smale, D.A., 2017. The influence of native macroalgal canopies on the distribution and abundance of the non-native kelp Undaria pinnatifida in natural reef habitats. Marine Biology, 164 (7). DOI https://doi.org/10.1007/s00227-017-3183-0
De Montaudouin, X., Andemard, C. & Labourg, P-J., 1999. Does the slipper limpet (Crepidula fornicata L.) impair oyster growth and zoobenthos diversity ? A revisited hypothesis. Journal of Experimental Marine Biology and Ecology, 235, 105-124.
De Montaudouin, X., Blanchet, H. & Hippert, B., 2018. Relationship between the invasive slipper limpet Crepidula fornicata and benthic megafauna structure and diversity, in Arcachon Bay. Journal of the Marine Biological Association of the United Kingdom, 98 (8), 2017-2028. DOI https://doi.org/10.1017/s0025315417001655
De Montaudoüin, X., Labarraque, D., Giraud, K. & Bachelet, G., 2001. Why does the introduced gastropod Crepidula fornicata fail to invade Arcachon Bay (France)? Journal of the Marine Biological Association of the United Kingdom, 81 (1), 97-104. DOI https://doi.org/10.1017/S0025315401003447
De Rijcke, M., Van Acker, E., Nevejan, N., De Schamphelaere, K.A.C. & Janssen, C.R., 2016. Toxic dinoflagellates and Vibrio spp. act independently in bivalve larvae. Fish & Shellfish Immunology, 57, 236–242. DOI https://doi.org/10.1016/j.fsi.2016.08.027
De Rijcke, M., Vandegehuchte, M.B., Bussche, J.V., Nevejan, N., Vanhaecke, L., De Schamphelaere, K.A.C. & Janssen, C.R., 2015. Common European harmful algal blooms affect the viability and innate immune responses of Mytilus edulis larvae. Fish & Shellfish Immunology, 47 (1), 175–181. DOI https://doi.org/10.1016/j.fsi.2015.09.003
Denny, M.W., 1987. Lift as a mechanism of patch initiation in mussel beds. Journal of Experimental Marine Biology and Ecology, 113, 231-45
Dereuder, E. T. R., Otto, S., Rehder, G. & Sokolova, I. M., 2025. Diel-cycling hypoxia and hypercapnia interact with the physiological and redox response of the bivalve Mytilus edulis to heat-wave. Marine Environmental Research, 209. DOI https://doi.org/10.1016/j.marenvres.2025.107241
Devinny, J. & Volse, L., 1978. Effects of sediments on the development of Macrocystis pyrifera gametophytes. Marine Biology, 48 (4), 343-348.
Devlin, M.J., Barry, J., Mills, D.K., Gowen, R.J., Foden, J., Sivyer, D. & Tett, P., 2008. Relationships between suspended particulate material, light attenuation and Secchi depth in UK marine waters. Estuarine, Coastal and Shelf Science, 79 (3), 429-439.
Diaz, R.J. & Rosenberg, R., 1995. Marine benthic hypoxia: a review of its ecological effects and the behavioural responses of benthic macrofauna. Oceanography and Marine Biology: an Annual Review, 33, 245-303.
Dickey, G., Preziosi, B.M., Clark, C.T. & Bowden, T.J., 2018. The impact of ocean acidification on the byssal threads of the blue mussel (Mytilus edulis). PLOS ONE, 13 (10), e0205908. DOI https://doi.org/10.1371/journal.pone.0205908
Dieck, T.I., 1992. North Pacific and North Atlantic digitate Laminaria species (Phaeophyta): hybridization experiments and temperature responses. Phycologia, 31, 147-163.
Dieck, T.I., 1993. Temperature tolerance and survival in darkness of kelp gametophytes (Laminariales: Phaeophyta) - ecological and biogeographical implications. Marine Ecology Progress Series, 100, 253-264.
Diederich, S., 2005. Differential recruitment of introduced Pacific oysters and native mussels at the North Sea coast: coexistence possible? Journal of Sea Research, 53 (4), 269-281.
Dijkstra, J. A. & Nolan, R., 2011. Potential of the invasive colonial ascidian, Didemnum vexillum, to limit escape response of the sea scallop, Placopecten magellanicus. Aquatic Invasions, 6 (4), 451-456. DOI https://doi.org/10.3391/ai.2011.6.4.10
Dijkstra, J., Harris, L.G. & Westerman, E., 2007. Distribution and long-term temporal patterns of four invasive colonial ascidians in the Gulf of Maine. Journal of Experimental Marine Biology and Ecology, 342 (1), 61-68. DOI https://doi.org/10.1016/j.jembe.2006.10.015
Dobretsov, S. & Wahl, M., 2008. Larval recruitment of the blue mussel Mytilus edulis: the effect of flow and algae. Journal of Experimental Marine Biology and Ecology, 355, 137-44
Dolmer, P. & Svane, I. 1994. Attachment and orientation of Mytilus edulis L. in flowing water. Ophelia, 40, 63-74
Dommasnes, A., 1968. Variation in the meiofauna of Corallina officinalis with wave exposure. Sarsia, 34, 117-124.
Eckman, J.E., 1983. Hydrodynamic processes affecting benthic recruitment 1. Limnology and Oceanography, 28 (2), 241-257.
Eckman, J.E. & Duggins, D.O., 1991. Life and death beneath macrophyte canopies: effects of understory kelps on growth rates and survival of marine, benthic suspension feeders. Oecologia, 87, 473-487.
Edwards, A., 1980. Ecological studies of the kelp Laminaria hyperborea and its associated fauna in south-west Ireland. Ophelia, 9, 47-60.
Eggermont, M., Bossier, P., Pande, G.S.J., Delahaut, V., Rayhan, A.M., Gupta, N., Islam, S.S., Yumo, E., Nevejan, N., Sorgeloos, P., Gomez-Gil, B. & Defoirdt, T., 2017. Isolation of Vibrionaceae from wild blue mussel (Mytilus edulis) adults and their impact on blue mussel larviculture. Fems Microbiology Ecology, 93 (4). DOI https://doi.org/10.1093/femsec/fix039
Elner, R.W. & Vadas, R.L., 1990. Inference in ecology: the sea urchin phenomenon in the northwest Atlantic. American Naturalist, 136, 108-125.
Engelen, A.H., Leveque, L., Destombe, C. & Valer, M., 2011. Spatial and temporal patterns of recovery of low intertidal Laminaria digitata after experimental spring and autumn removal. Cahiers De Biologie Marine, 52 (4), 441-453.
Engelen, A.H., Serebryakova, A., Ang, P., Britton-Simmons, K., Mineur, F., Pedersen, M. F., & Toth, G., 2015. Circumglobal invasion by the brown seaweed Sargassum muticum. Oceanography and Marine Biology: An Annual Review, 53, 81-126.
Epstein, G. & Smale, D.A., 2017. Undaria pinnatifida: A case study to highlight challenges in marine invasion ecology and management. Ecology and Evolution, 7 (20), 8624-8642. DOI https://doi.org/10.1002/ece3.3430
Epstein, G. & Smale, D.A., 2018. Environmental and ecological factors influencing the spillover of the non-native kelp, Undaria pinnatifida, from marinas into natural rocky reef communities. Biological Invasions, 20 (4), 1049-1072. DOI https://doi.org/10.1007/s10530-017-1610-2
Epstein, G., Foggo, A. & Smale, D.A., 2019a. Inconspicuous impacts: Widespread marine invader causes subtle but significant changes in native macroalgal assemblages. Ecosphere, 10 (7). DOI https://doi.org/10.1002/ecs2.2814
Epstein, G., Hawkins, S.J. & Smale, D.A., 2019b. Identifying niche and fitness dissimilarities in invaded marine macroalgal canopies within the context of contemporary coexistence theory. Scientific Reports, 9. DOI https://doi.org/10.1038/s41598-019-45388-5
Erwin, D.G., Picton, B.E., Connor, D.W., Howson, C.M., Gilleece, P. & Bogues, M.J., 1990. Inshore Marine Life of Northern Ireland. Report of a survey carried out by the diving team of the Botany and Zoology Department of the Ulster Museum in fulfilment of a contract with Conservation Branch of the Department of the Environment (N.I.)., Ulster Museum, Belfast: HMSO.
Essink, K., 1999. Ecological effects of dumping of dredged sediments; options for management. Journal of Coastal Conservation, 5, 69-80.
Ewers, R., Kasperk, C. & Simmons, B., 1987. Biologishes Knochenimplantat aus Meeresalgen. Zahnaerztliche Praxis, 38, 318-320.
Ezgeta-Balic, D., Radonic, I., Varezic, D. B., Zorica, B., Arapov, J., Staglicic, N., Jozic, S., Peharda, M., Briski, E., Lin, Y. P. & Segvic-Bubic, T., 2020. Reproductive cycle of the non-native Pacific oyster, Crassostrea gigas, in the Adriatic Sea. Mediterranean Marine Science, 21 (1), 146-156. DOI https://doi.org/10.12681/mms.21304
Ezgeta-Balic, D., Segvic-Bubic, T., Staglicic, N., Lin, Y. P., Bojanic Varezic, D., Grubisic, L. & Briski, E., 2019. Distribution of non-native Pacific oyster Magallana gigas (Thunberg, 1793) along the eastern Adriatic coast. Acta Adriatica, 60 (2), 137-146. DOI https://doi.org/10.32582/aa.60.2.3
FAO (Food and Agriculture Organization of the United Nations), 2007. Aquaculture production: values 1984-2005. FISHSTAT Plus - Universal software for fishery statistical time series [online or CD-ROM]. Fishery Information, Data and Statistics Unit. Food and Agriculture Organization of the United Nations, Rome, Italy.
Farrell, P. & Fletcher, R., 2006. An investigation of dispersal of the introduced brown alga Undaria pinnatifida (Harvey) Suringar and its competition with some species on the man-made structures of Torquay Marina (Devon, UK). Journal of Experimental Marine Biology and Ecology, 334 (2), 236-243.
Fernández, P.A., Roleda, M.Y. & Hurd, C.L., 2015. Effects of ocean acidification on the photosynthetic performance, carbonic anhydrase activity and growth of the giant kelp Macrocystis pyrifera. 124 (3), 293-304. DOI https://doi.org/10.1007/s11120-015-0138-5
Fitzer, S.C., Wenzhong, Z.K., Tanner, E., Phoenix, V.R., Kamenos, N.A. & Cusack, M., 2015. Ocean acidification alters the material properties of Mytilus edulis shells. Journal of the Royal Society. Interface, 12 (103). DOI https://doi.org/10.1098/rsif.2014.1227
Fletcher, R. & Farrell, P., 1998. Introduced brown algae in the North East Atlantic, with particular respect to Undaria pinnatifida (Harvey) Suringar. Helgolander Meeresuntersuchungen, 52 (3-4), 259-275.
Fletcher, R.L., 1996. The occurrence of 'green tides' - a review. In Marine Benthic Vegetation. Recent changes and the Effects of Eutrophication (ed. W. Schramm & P.H. Nienhuis). Berlin Heidelberg: Springer-Verlag. [Ecological Studies, vol. 123].
Fly, E.K., Hilbish, T.J., Wethey, D.S. & Rognstad, R.L., 2015. Physiology and biogeography: The response of European mussels (Mytilus spp.) to climate change. American Malacological Bulletin, 33 (1), 136–149. DOI https://doi.org/10.4003/006.033.0111
Franco, J. N., Tuya, F., Bertocci, I., Rodríguez, L., Martínez, B., Sousa-Pinto, I. & Arenas, F., 2018. The ‘golden kelp’ Laminaria ochroleuca under global change: integrating multiple eco-physiological responses with species distribution models. Journal of Ecology, 106 (1), 47–58. DOI https://doi.org/10.1111/1365-2745.12810
Franz, M., Barboza, F.R., Hinrichsen, H.H., Lehmann, A., Scotti, M., Hiebenthal, C., Molis, M., Schütt, R. & Wahl, M., 2019. Long-term records of hard-bottom communities in the southwestern Baltic Sea reveal the decline of a foundation species. Estuarine Coastal and Shelf Science, 219, 242–251. DOI https://doi.org/10.1016/j.ecss.2019.02.029
Frechette, M., Butman, C.A., Geyer, W.R., 1989. The importance of boundary-layer flow in supplying phytoplankton to the benthic suspension feeder, Mytilus edulis L. Limnology and Oceanography, 34, 19-36.
Fredersdorf, J., Müller, R., Becker, S., Wiencke, C. & Bischof, K., 2009. Interactive effects of radiation, temperature and salinity on different life history stages of the Arctic kelp Alaria esculenta (Phaeophyceae). Oecologia, 160 (3), 483-492.
Fredriksen, S., Sjøtun, K., Lein, T.E. & Rueness, J., 1995. Spore dispersal in Laminaria hyperborea (Laminariales, Phaeophyceae). Sarsia, 80 (1), 47-53.
Frieder, C., Nam, S., Martz, T. & Levin, L., 2012. High temporal and spatial variability of dissolved oxygen and pH in a nearshore California kelp forest. Biogeosciences, 9 (10), 3917-3930.
Frölicher, T.L., Fischer, E.M. & Gruber, N., 2018. Marine heatwaves under global warming. Nature, 560 (7718), 360-364. DOI https://doi.org/10.1038/s41586-018-0383-9
Garrard, S.L., Gambi, M.C., Scipione, M.B., Patti, F.P., Lorenti, M., Zupo, V., Paterson, D.M. & Buia, M.C., 2014. Indirect effects may buffer negative responses of seagrass invertebrate communities to ocean acidification. Journal of Experimental Marine Biology and Ecology, 461, 31-38. DOI https://doi.org/10.1016/j.jembe.2014.07.011
GBNNSIP, 2011b. Risk assessment for Crassostrea gigas. GB Non-native Species Information Portal, GB Non-native Species Secretariat. Available from: https://www.nonnativespecies.org/assets/Uploads/RA_Crassostrea_gigas_finalpoc.pdf
GBNNSIP, 2012. Pacific oyster Magallana gigas. Factsheet. GB Non-native Species Information Portal, [online] GB Non-native Species Secretariat. [Accessed July 2024]. Available from: https://www.nonnativespecies.org/non-native-species/information-portal/view/1013
Gendre, H., Ben Cheikh, Y., Le Foll, F., Geffard, A. & Ladeiro, M.P., 2023. Comparative immune responses of blue mussel and zebra mussel haemocytes to simultaneous chemical and bacterial exposure. Fish & Shellfish Immunology, 135. DOI https://doi.org/10.1016/j.fsi.2023.108654
Giltrap, M., Ronan, J., Hardenberg, S., Parkes, G., McHugh, B., McGovern, E. & Wilson, J., 2013. Assessment of biomarkers in Mytilus edulis to determine good environmental status for implementation of MSFD in Ireland. Marine Pollution Bulletin, 71 (1), 240-249.
Gittenberger, A, Rensing, M, Dekker, R, Niemantsverdriet, P, Schrieken, N & Stegenga, H, 2015. Native and non-native species of the Dutch Wadden Sea in 2014. Issued by Office for Risk Assessment and Research, The Netherlands Food and Consumer Product Safety Authority.
Gittenberger, A., 2007. Recent population expansions of non-native ascidians in The Netherlands. Journal of Experimental Marine Biology and Ecology, 342 (1), 122-126. DOI https://doi.org/10.1016/j.jembe.2006.10.022
Gommez, J.L.C. & Miguez-Rodriguez, L.J., 1999. Effects of oil pollution on skeleton and tissues of Echinus esculentus L. 1758 (Echinodermata, Echinoidea) in a population of A Coruna Bay, Galicia, Spain. In Echinoderm Research 1998. Proceedings of the Fifth European Conference on Echinoderms, Milan, 7-12 September 1998, (ed. M.D.C. Carnevali & F. Bonasoro) pp. 439-447. Rotterdam: A.A. Balkema.
- Gonzalez, J.G. & Yevich, P., 1976. Responses of an estuarine population of the blue mussel Mytilus edulis to heated water from a steam generating plant. Marine Biology, 34 (2), 177-189. DOI https://doi.org/10.1007/BF00390760
Gordillo, F. J. L., Carmona, R., Viñegla, B., Wiencke, C. & Jiménez, C., 2016. Effects of simultaneous increase in temperature and ocean acidification on biochemical composition and photosynthetic performance of common macroalgae from Kongsfjorden (Svalbard). Polar Biology, 39 (11), 1993–2007. DOI https://doi.org/10.1007/s00300-016-1897-y
Gordillo, F., Carmona, R. & Jimenez, C., 2022. A Warmer Arctic Compromises Winter Survival of Habitat-Forming Seaweeds. Frontiers in Marine Science, 8. DOI https://doi.org/10.3389/fmars.2021.750209
Gordillo, F.J.L., Aguilera, J., Wiencke, C. & Jiménez, C., 2015. Ocean acidification modulates the response of two Arctic kelps to ultraviolet radiation. Journal of Plant Physiology, 173, 41-50. DOI https://doi.org/10.1016/j.jplph.2014.09.008
Gorman, D., Bajjouk, T., Populus, J., Vasquez, M. & Ehrhold, A., 2013. Modeling kelp forest distribution and biomass along temperate rocky coastlines. Marine Biology, 160 (2), 309-325.
Gosling, E.M. (ed.), 1992a. The mussel Mytilus: ecology, physiology, genetics and culture. Amsterdam: Elsevier Science Publ. [Developments in Aquaculture and Fisheries Science, no. 25]
Grahame, J., & Hanna, F.S., 1989. Factors affecting the distribution of the epiphytic fauna of Corallina officinalis (L.) on an exposed rocky shore. Ophelia, 30, 113-129.
Grandy, N., 1984. The effects of oil and dispersants on subtidal red algae. Ph.D. Thesis. University of Liverpool.
Gray, A.R., Lucas, I.A.N, Seed, R. & Richardson, C.A., 1999. Mytilus edulis chilensis infested with Coccomyxa parasitica (Chlorococcales, Coccomyxaceae). Journal of Molluscan Studies, 65, 289-294.
Gray, J.S., Wu R.S.-S. & Or Y.Y., 2002. Effects of hypoxia and organic enrichment on the coastal marine environment. Marine Ecology Progress Series, 238, 249-279. DOI https://doi.org/10.3354/meps238249
Greatorex, R. & Knights, A.M., 2023. Differential effects of ocean acidification and warming on biological functioning of a predator and prey species may alter future trophic interactions. Marine Environmental Research, 186. DOI https://doi.org/10.1016/j.marenvres.2023.105903
Griffith, K., Mowat, S., Holt, R.H., Ramsay, K., Bishop, J.D., Lambert, G. & Jenkins, S.R., 2009. First records in Great Britain of the invasive colonial ascidian Didemnum vexillum Kott, 2002. Aquatic Invasions, 4 (4), 581-590.
Grimmelpont, M., Payton, L., Lefrançois, C. & Tran, D., 2024. Molecular and behavioural responses of the mussel Mytilus edulis exposed to a marine heatwave. Marine Environmental Research, 196. DOI https://doi.org/10.1016/j.marenvres.2024.106418
Groenewold, S. & Fonds, M., 2000. Effects on benthic scavengers of discards and damaged benthos produced by the beam-trawl fishery in the southern North Sea. ICES Journal of Marine Science, 57 (5), 1395-1406.
Groner, F., Lenz, M., Wahl, M. & Jenkins, S.R., 2011. Stress resistance in two colonial ascidians from the Irish Sea: The recent invader Didemnum vexillum is more tolerant to low salinity than the cosmopolitan Diplosoma listerianum. Journal of Experimental Marine Biology and Ecology, 409 (1), 48-52. DOI https://doi.org/10.1016/j.jembe.2011.08.002
Gruffydd, L.D., Huxley, R. & Crisp, D., 1984. The reduction in growth of Mytilus edulis in fluctuating salinity regimes measured using laser diffraction patterns and the exaggeration of this effect by using tap water as the diluting medium. Journal of the Marine Biological Association of the United Kingdom, 64, 401-9.
Guillou, E., Androuin, T., Toupoint, N. & Tremblay, R., 2023. Selective pressure on ontogenic stages of blue mussels (Mytilus edulis, L.). Journal of Experimental Marine Biology and Ecology, 568. DOI https://doi.org/10.1016/j.jembe.2023.151940
Guinle, C., Gurning, R.W., Baratange, C., Cognie, B., Mossion, A., Wielgosz-Collin, G., Bertrand, S., Montiel, G., Poirier, L., Deleris, P. & Zalouk-Vergnoux, A., 2025. Integrating multi-level approaches to assess blue mussel (Mytilus spp.) responses to short-term temperature and salinity changes. Marine Environmental Research, 211. DOI https://doi.org/10.1016/j.marenvres.2025.107436
Guiry, M.D. & Blunden, G., 1991. Seaweed Resources in Europe: Uses and Potential. Chicester: John Wiley & Sons.
Hammer, L., 1972. Anaerobiosis in marine algae and marine phanerograms. In Proceedings of the Seventh International Seaweed Symposium, Sapporo, Japan, August 8-12, 1971 (ed. K. Nisizawa, S. Arasaki, Chihara, M., Hirose, H., Nakamura V., Tsuchiya, Y.), pp. 414-419. Tokyo: Tokyo University Press.
Hansen, B.W., Dolmer, P. & Vismann, B., 2023. Too late for regulatory management on Pacific oysters in European coastal waters? Journal of Sea Research, 191. DOI https://doi.org/10.1016/j.seares.2022.102331
Haque, M.N. & Kwon, S., 2018. Effect of ultra-sonication and its use with sodium hypochlorite as antifouling method against Mytilus edulis larvae and mussel. Environmental Geochemistry and Health, 40 (1), 209–215. DOI https://doi.org/10.1007/s10653-016-9894-1
Harger, J.R.E. & Landenberger, D.E., 1971. The effects of storms as a density dependent mortality factor on populations of sea mussels. The Veliger, 14, 195-210.
Harkin, E., 1981. Fluctuations in epiphyte biomass following Laminaria hyperborea canopy removal. In Proceedings of the Xth International Seaweed Symposium, Gø teborg, 11-15 August 1980 (ed. T. Levring), pp.303-308. Berlin: Walter de Gruyter.
Harlin, M.M., & Lindbergh, J.M., 1977. Selection of substrata by seaweed: optimal surface relief. Marine Biology, 40, 33-40.
Hawkins, A., Smith, R., Bayne, B. & Heral, M., 1996. Novel observations underlying the fast growth of suspension-feeding shellfish in turbid environments: Mytilus edulis. Marine Ecology Progress Series, 131, 179-90
Hawkins, S.J. & Harkin, E., 1985. Preliminary canopy removal experiments in algal dominated communities low on the shore and in the shallow subtidal on the Isle of Man. Botanica Marina, 28, 223-30.
Hawkins, S.J. & Hartnoll, R.G., 1985. Factors determining the upper limits of intertidal canopy-forming algae. Marine Ecology Progress Series, 20, 265-271.
Hayward, P.J. 1988. Animals on seaweed. Richmond, Surrey: Richmond Publishing Co. Ltd. [Naturalists Handbooks 9].
Heiser, S., Hall-Spencer, J.M. & Hiscock, K., 2014. Assessing the extent of establishment of Undaria pinnatifida in Plymouth Sound Special Area of Conservation, UK. Marine Biodiversity Records, 7, e93. DOI https://doi.org/10.1017/S1755267214000608
Helmer, L., Farrell, P., Hendy, I., Harding, S., Robertson, M. & Preston, J., 2019. Active management is required to turn the tide for depleted Ostrea edulis stocks from the effects of overfishing, disease and invasive species. Peerj, 7 (2). DOI https://doi.org/10.7717/peerj.6431
Helmuth, B., Harley, C.D., Halpin, P.M., O'Donnell, M., Hofmann, G.E. & Blanchette, C.A., 2002. Climate change and latitudinal patterns of intertidal thermal stress. Science, 298 (5595), 1015-1017.
Herbert, R.J.H., Humphreys, J., Davies, C.J., Roberts, C., Fletcher, S. & Crowe, T.P., 2016. Ecological impacts of non-native Pacific oysters (Crassostrea gigas) and management measures for protected areas in Europe. Biodiversity and Conservation, 25 (14), 2835-2865. DOI https://doi.org/10.1007/s10531-016-1209-4
Herbert, R.J.H., Roberts, C., Humphreys, J., & Fletcher, S. 2012. The Pacific oyster (Crassostrea gigas) in the UK: economic, legal and environmental issues associated with its cultivation, wild establishment and exploitation. Available from: https://www.daera-ni.gov.uk/publications/pacific-oyster-uk-issues-associated-its-cultivation-wild-establishment-and-exploitation
Herborg, L.M., O’Hara, P. & Therriault, T.W., 2009. Forecasting the potential distribution of the invasive tunicate Didemnum vexillum. Journal of Applied Ecology, 46 (1), 64-72. DOI https://doi.org/10.1111/j.1365-2664.2008.01568.x
Hiebenthal, C., Philipp, E.E.R., Eisenhauer, A. & Wahl, M., 2013. Effects of seawater pCO2 and temperature on shell growth, shell stability, condition and cellular stress of Western Baltic Sea Mytilus edulis (L.) and Arctica islandica (L.). Marine Biology, 160 (8), 2073-2087.
Hill, T., 1993. Algal zonation in the sublittoral fringe: the importance of competition. Ph.D. Thesis., University of Liverpool, Liverpool, UK.
Hinz, H., Capasso, E., Lilley, M., Frost, M. & Jenkins, S.R., 2011b. Temporal differences across a bio-geographical boundary reveal slow response of sub-littoral benthos to climate change. Marine Ecology Progress Series, 423, 69-82. DOI https://doi.org/10.3354/meps08963
Hiscock, K. & Hoare, R., 1975. The ecology of sublittoral communities at Abereiddy Quarry, Pembrokeshire. Journal of the Marine Biological Association of the United Kingdom, 55 (4), 833-864.
Hiscock, K. & Mitchell, R., 1980. The Description and Classification of Sublittoral Epibenthic Ecosystems. In The Shore Environment, Vol. 2, Ecosystems, (ed. J.H. Price, D.E.G. Irvine, & W.F. Farnham), 323-370. London and New York: Academic Press. [Systematics Association Special Volume no. 17(b)].
Hiscock, K., 1983. Water movement. In Sublittoral ecology. The ecology of shallow sublittoral benthos (ed. R. Earll & D.G. Erwin), pp. 58-96. Oxford: Clarendon Press.
Hitchin, B., 2012. New outbreak of Didemnum vexillum in North Kent: on stranger shores. Porcupine Marine Natural History Society Newsletter, 31, 43-48.
Hobday, A.J., Alexander, L.V., Perkins, S.E., Smale, D.A., Straub, S.C., Oliver, E.C.J., Benthuysen, J.A., Burrows, M.T., Donat, M.G., Feng, M., Holbrook, N.J., Moore, P.J., Scannell, H.A., Sen Gupta, A. & Wernberg, T., 2016. A hierarchical approach to defining marine heatwaves. Progress in Oceanography, 141, 227-238. DOI https://doi.org/10.1016/j.pocean.2015.12.014
Hofmann, L.C., Straub, S. & Bischof, K., 2013. Elevated CO2 levels affect the activity of nitrate reductase and carbonic anhydrase in the calcifying rhodophyte Corallina officinalis. Journal of Experimental Botany, 64 (4), 899-908. DOI https://doi.org/10.1093/jxb/ers369
Holt, R., 2024. GB Non-native organism risk assessment for Didemnum vexillum. GB Non-native Species Information Portal, GB Non-native Species Secretariat. Available from: https://www.nonnativespecies.org/assets/Uploads/Didemnum-vexillum-final_forwebsite.pdf
Holt, T.J., Jones, D.R., Hawkins, S.J. & Hartnoll, R.G., 1995. The sensitivity of marine communities to man induced change - a scoping report. Countryside Council for Wales, Bangor, Contract Science Report, no. 65.
Holt, T.J., Rees, E.I., Hawkins, S.J. & Seed, R., 1998. Biogenic reefs (Volume IX). An overview of dynamic and sensitivity characteristics for conservation management of marine SACs. Scottish Association for Marine Science (UK Marine SACs Project), 174 pp. Available from: http://ukmpa.marinebiodiversity.org/uk_sacs/pdfs/biogreef.pdf
Hopkin, R. & Kain, J.M., 1978. The effects of some pollutants on the survival, growth and respiration of Laminaria hyperborea. Estuarine and Coastal Marine Science, 7, 531-553.
Hubert, J., Booms, E., Witbaard, R. & Slabbekoorn, H., 2022. Responsiveness and habituation to repeated sound exposures and pulse trains in blue mussels. Journal of Experimental Marine Biology and Ecology, 547. DOI https://doi.org/10.1016/j.jembe.2021.151668
Hull, S., 1997. Seasonal changes in diversity and abundance of ostracodes on four species of intertidal algae with differing structural complexity. Marine Ecology Progress Series, 161, 71-82.
Humphreys, J., Herbert, R. J. H., Roberts, C. & Fletcher, S., 2014. A reappraisal of the history and economics of the Pacific oyster in Britain. Aquaculture, 428-429, 117–124. DOI https://doi.org/10.1016/j.aquaculture.2014.02.034
Hutchison, Z.L., Hendrick, V.J., Burrows, M.T., Wilson, B. & Last, K.S., 2016. Buried Alive: The Behavioural Response of the Mussels, Modiolus modiolus and Mytilus edulis to Sudden Burial by Sediment. PLoS ONE, 11 (3), e0151471.
Hutchison, Z.L., Secor, D.H. & Gill, A.B., 2020. The interaction between resource species an electromagnetic fields associated with electricity production by offshore wind farms. Oceanography, 33 (4), 96–107. DOI https://doi/org/10.5670/oceanog.2020.409
Huthnance, J., 2010. Ocean Processes Feeder Report. London, DEFRA on behalf of the United Kingdom Marine Monitoring and Assessment Strategy (UKMMAS) Community.
Iñiguez, C., Carmona, R., Lorenzo, M.R., Niell, F.X., Wiencke, C. & Gordillo, F.J.L., 2016b. Increased temperature, rather than elevated CO2, modulates the carbon assimilation of the Arctic kelps Saccharina latissima and Laminaria solidungula. 163 (12), 248. DOI https://doi.org/10.1007/s00227-016-3024-6
Incze, L.S., Lutz, R.A. & Watling, L., 1980. Relationships between effects of environmental temperature and seston on growth and mortality of Mytilus edulis in a temperate northern estuary. Marine Biology, 57 (3), 147-156. DOI https://doi.org/10.1007/BF00390733
Järnegren, J.; Gulliksen, B.; Husa, V.; Malmstrøm, M.; Oug, E.; Berg, P.R.; Bryn, A.; Geange, S.R.; Hindar, K.; Hole, L.R.; Kausrud, K.L.; Kirkendall, L.R.; Nielsen, A.; Sandercock, B.K.; Thorstad, E.B.; Velle, G., 2023. Assessment of risk and risk-reducing measures related to the introduction and dispersal of the invasive alien carpet tunicate Didemnum vexillum in Norway. Scientific Opinion of the Panel on Biodiversity of the Norwegian Scientific Committee for Food and Environment.
Jönsson, M. & Nordberg, E. K., 2024. Chemical food safety of seaweed: Species, spatial and thallus dependent variation of potentially toxic elements (PTEs) and techniques for their removal. Journal of Applied Phycology, 36 (2), 765–781. DOI https://doi.org/10.1007/s10811-023-03131-8
Jackson, A.C. & McIlvenny, J., 2011. Coastal squeeze on rocky shores in northern Scotland and some possible ecological impacts. Journal of Experimental Marine Biology and Ecology, 400 (1), 314-321. DOI https://doi.org/10.1016/j.jembe.2011.02.012
Jacobson, M.Z., 2005. Studying ocean acidification with conservative, stable numerical schemes for nonequilibrium air-ocean exchange and ocean equilibrium chemistry. Journal of Geophysical Research: Atmospheres, 110 (D7). DOI https://doi.org/10.1029/2004JD005220
James, K, 2017. A review of the impacts from invasion by the introduced kelp Undaria pinnatifida. Waikato Regional Council Technical Report 2016/40, Institute of Marine Science, University of Auckland, Hamilton, 40 pp. Available from: https://www.waikatoregion.govt.nz/assets/WRC/WRC-2019/TR201640.pdf
Jenner, H.A., Whitehouse, J.W., Taylor, C.J. & Khalanski, M. 1998. Cooling water management in European power stations Biology and control of fouling. Hydroécologie Appliquée, 10, I-225.
JNCC (Joint Nature Conservation Committee), 1999. Marine Environment Resource Mapping And Information Database (MERMAID): Marine Nature Conservation Review Survey Database. [on-line] http://www.jncc.gov.uk/mermaid
JNCC (Joint Nature Conservation Committee), 2022. The Marine Habitat Classification for Britain and Ireland Version 22.04. [Date accessed]. Available from: https://mhc.jncc.gov.uk/
Johansson, I., Saurel, C., Taylor, D., Petersen, J.K. & Nielsen, P., 2024. Longevity of subtidal mussel beds ( Mytilus edulis ) in eutrophic coastal areas. Journal of Sea Research, 199. DOI https://doi.org/10.1016/j.seares.2024.102506
Johnston, E.L. & Roberts, D.A., 2009. Contaminants reduce the richness and evenness of marine communities: a review and meta-analysis. Environmental Pollution, 157 (6), 1745-1752.
Jones, C.G., Lawton, J.H. & Shackak, M., 1994. Organisms as ecosystem engineers. Oikos, 69, 373-386.
Jones, D.J., 1971. Ecological studies on macro-invertebrate communities associated with polluted kelp forest in the North Sea. Helgolander Wissenschaftliche Meersuntersuchungen, 22, 417-431.
Jones, L.A., Hiscock, K. & Connor, D.W., 2000. Marine habitat reviews. A summary of ecological requirements and sensitivity characteristics for the conservation and management of marine SACs. Joint Nature Conservation Committee, Peterborough. (UK Marine SACs Project report.). Available from: http://ukmpa.marinebiodiversity.org/uk_sacs/pdfs/marine-habitats-review.pdf
Jones, N.J.E., Ridgway, I.D. & Richardson, C.A., 2009. Transport of cuttlefish, Sepia officinalis, eggs under dry and damp conditions. Journal of Molluscan Studies, 75, 192-194.
Jones, N.S. & Kain, J.M., 1967. Subtidal algal recolonisation following removal of Echinus. Helgolander Wissenschaftliche Meeresuntersuchungen, 15, 460-466.
Jones, S.J., Lima, F.P. & Wethey, D.S., 2010. Rising environmental temperatures and biogeography: poleward range contraction of the blue mussel, Mytilus edulis L., in the western Atlantic. Journal of Biogeography 37: 2243-59
Jorgensen, B.B., 1980. Seasonal oxygen depletion in the bottom waters of a Danish fjord and its effect on the benthic community. Oikos, 32, 68-76.
Jung, A. S., van der Veer, H. W., van der Meer, M. T. J. & Philippart, C. J. M., 2019. Seasonal variation in the diet of estuarine bivalves. Plos One, 14 (6). DOI https://doi.org/10.1371/journal.pone.0217003
Kain, J.M., 1964. Aspects of the biology of Laminaria hyperborea III. Survival and growth of gametophytes. Journal of the Marine Biological Association of the United Kingdom, 44 (2), 415-433.
Kain, J.M. & Svendsen, P., 1969. A note on the behaviour of Patina pellucida in Britain and Norway. Sarsia, 38, 25-30.
Kain, J.M., 1971a. Synopsis of biological data on Laminaria hyperborea. FAO Fisheries Synopsis, no. 87.
Kain, J.M., 1975a. Algal recolonization of some cleared subtidal areas. Journal of Ecology, 63, 739-765.
Kain, J.M., 1979. A view of the genus Laminaria. Oceanography and Marine Biology: an Annual Review, 17, 101-161.
Kain, J.M., 1987. Photoperiod and temperature as triggers in the seasonality of Delesseria sanguinea. Helgolander Meeresuntersuchungen, 41, 355-370.
Kain, J.M., & Norton, T.A., 1990. Marine Ecology. In Biology of the Red Algae, (ed. K.M. Cole & Sheath, R.G.). Cambridge: Cambridge University Press.
Kain, J.M., Drew, E.A. & Jupp, B.P., 1975. Light and the ecology of Laminaria hyperborea II. In Proceedings of the Sixteenth Symposium of the British Ecological Society, 26-28 March 1974. Light as an Ecological Factor: II (ed. G.C. Evans, R. Bainbridge & O. Rackham), pp. 63-92. Oxford: Blackwell Scientific Publications.
Kaiser, M.J., & Spencer, B.E., 1994a. A preliminary assessment of the immediate effects of beam trawling on a benthic community in the Irish Sea. In Environmental impact of bottom gears on benthic fauna in relation to natural resources management and protection of the North Sea. (ed. S.J. de Groot & H.J. Lindeboom). NIOZ-Rapport, 11, 87-94.
Kamermans, P. & Saurel, C., 2022. Interacting climate change effects on mussels (Mytilus edulis and M. galloprovincialis) and oysters (Crassostrea gigas and Ostrea edulis): experiments for bivalve individual growth models. Aquatic Living Resources, 35. DOI https://doi.org/10.1051/alr/2022001
Kaplanis, N., Edwards, C., Eynaud, Y. & Smith, J., 2019. Future sea-level rise drives rocky intertidal habitat loss and benthic community change. Preprint. Bioxiv. DOI https://doi.org/10.1101/553933
Karsten, U., 2007. Research note: salinity tolerance of Arctic kelps from Spitsbergen. Phycological Research, 55 (4), 257-262.
Kervarec, F., Arzel, P. & Guyader, O., 1999. Fisher Behaviour and Economic Interactions Between Fisheries: Examining Seaweed and Scallop Fisheries of the Brest District (Western Brittany, France). The XIth Annual Conference of the European Association of Fisheries Economists. 6th-10th April 1999, Dublin, pp.
Kindig, A.C., & Littler, M.M., 1980. Growth and primary productivity of marine macrophytes exposed to domestic sewage effluents. Marine Environmental Research, 3, 81-100.
King, N. G., Leathers, T., Smith, K. E. & Smale, D. A., 2024. The influence of pre-exposure to marine heatwaves on the critical thermal maxima (CTmax) of marine foundation species. Functional Ecology. DOI https://doi.org/10.1111/1365-2435.14622
Kinne, O. (ed.), 1971a. Marine Ecology: A Comprehensive, Integrated Treatise on Life in Oceans and Coastal Waters. Vol. 1 Environmental Factors, Part 2. Chichester: John Wiley & Sons.
Kinne, O., 1977. International Helgoland Symposium "Ecosystem research": summary, conclusions and closing. Helgoländer Wissenschaftliche Meeresuntersuchungen, 30(1-4), 709-727.
Kitching, J., 1941. Studies in sublittoral ecology III. Laminaria forest on the west coast of Scotland; a study of zonation in relation to wave action and illumination. The Biological Bulletin, 80 (3), 324-337
Kittner, C. & Riisgaard, H.U., 2005. Effect of temperature on filtration rate in the mussel Mytilus edulis: no evidence for temperature compensation. Marine Ecology Progress Series 305: 147-52
Kleeman, S.N., 2009. Didemnum vexillum - Feasibility of Eradication and/or Control. CCW Contract Science report, 53 pp. Available from: https://www.nonnativespecies.org/assets/Management-documents/Kleeman_2009-1.pdf
Koch, M., Bowes, G., Ross, C. & Zhang, X.-H., 2013. Climate change and ocean acidification effects on seagrasses and marine macroalgae. Global Change Biology, 19 (1), 103-132. DOI https://doi.org/10.1111/j.1365-2486.2012.02791.x
Kochmann, J, 2012. Into the Wild Documenting and Predicting the Spread of Pacific Oysters (Crassostrea gigas) in Ireland. PhD Thesis, University College Dublin. Available from: https://www.tcd.ie/research/simbiosys/images/JKPhD.pdf
Kochmann, J., O’Beirn, F., Yearsley, J. & Crowe, T.P., 2013. Environmental factors associated with invasion: modelling occurrence data from a coordinated sampling programme for Pacific oysters. Biological Invasions, 15 (10), 2265-2279. DOI https://doi.org/10.1007/s10530-013-0452-9
Koehn, R.K. & Hilbish, T.J., 1987. The biochemical genetics and physiological adaptation of an enzyme polymorphism. American Scientist, 75, 134-141.
Koehn, R.K., 1983. Biochemical genetics and adaptation in molluscs. In The Mollusca. vol. 2. Environmental biochemistry and physiology, (ed. P.W. Hochachka),pp 305-330.
Kong, H., Jiang, X.Y., Clements, J.C., Wang, T., Huang, X.Z., Shang, Y.Y., Chen, J.F., Hu, M.H. & Wang, Y.J., 2019. Transgenerational effects of short-term exposure to acidification and hypoxia on early developmental traits of the mussel Mytilus edulis. Marine Environmental Research, 145, 73–80. DOI https://doi.org/10.1016/j.marenvres.2019.02.011
Kononenko, G. P., Burkin, A. A., Georgiev, A. A. & Georgieva, M. L., 2022. Mycotoxins in Macroalgae from the Velikaya Salma Strait of the Kandalaksha Gulf of the White Sea. Russian Journal of Marine Biology, 47 (6), 480–488. DOI https://doi.org/10.1134/S1063074021060080
Kotta, J., Futter, M., Kaasik, A., Liversage, K., Rätsep, M., Barboza, F.R., Bergström, L., Bergström, P., Bobsien, I., Díaz, E., Herkül, K., Jonsson, P.R., Korpinen, S., Kraufvelin, P., Krost, P., Lindahl, O., Lindegarth, M., Lyngsgaard, M.M., Mühl, M., Sandman, A.N., Orav-Kotta, H., Orlova, M., Skov, H., Rissanen, J., Siaulys, A., Vidakovic, A. & Virtanen, E., 2020. Cleaning up seas using blue growth initiatives: Mussel farming for eutrophication control in the Baltic Sea. Science of the Total Environment, 709. DOI https://doi.org/10.1016/j.scitotenv.2019.136144
Kraan, S., 2017. Undaria marching on; late arrival in the Republic of Ireland. Journal of Applied Phycology, 29 (2), 1107-1114. DOI https://doi.org/10.1007/s10811-016-0985-2
Kraan, S., 2020. Concise review of the genus Alaria Greville, 1830. JOURNAL OF APPLIED PHYCOLOGY, 32 (6), 3543-3560. DOI http://doi.org/10.1007/s10811-020-02222-0
Krause-Jensen, D., Duarte, C.M., Hendriks, I.E., Meire, L., Blicher, M.E., Marbà, N. & Sejr, M.K., 2015. Macroalgae contribute to nested mosaics of pH variability in a subarctic fjord. Biogeosciences, 12 (16), 4895-4911. DOI https://doi.org/10.5194/bg-12-4895-2015
Kregting, L., Blight, A., Elsäßer, B. & Savidge, G., 2013. The influence of water motion on the growth rate of the kelp Laminaria hyperborea. Journal of Experimental Marine Biology and Ecology, 448, 337-345.
Kreissig, K. J., Hansen, L. T., Jensen, P. E., Wegeberg, S., Geertz-Hansen, O. & Sloth, J. J., 2021. Characterisation and chemometric evaluation of 17 elements in ten seaweed species from Greenland. PLOS ONE, 16 (2), e0243672. DOI https://doi.org/10.1371/journal.pone.0243672
Kroeker, K.J., Micheli, F., Gambi, M.C. & Martz, T.R., 2011. Divergent ecosystem responses within a benthic marine community to ocean acidification. Proceedings of the National Academy of Sciences, 108 (35), 14515. DOI https://doi.org/10.1073/pnas.1107789108
Krumhansl, K.A., Lee, J.M. & Scheibling, R.E., 2011. Grazing damage and encrustation by an invasive bryozoan reduce the ability of kelps to withstand breakage by waves. Journal of Experimental Marine Biology and Ecology, 407 (1), 12-18. DOI: https://doi.org/10.1016/j.jembe.2011.06.033
Kruuk, H., Wansink, D. & Moorhouse, A., 1990. Feeding patches and diving success of otters, Lutra lutra, in Shetland. Oikos, 57, 68-72.
Laeseke, P., Bartsch, I. & Bischof, K., 2019. Effects of kelp canopy on underwater light climate and viability of brown algal spores in Kongsfjorden (Spitsbergen). Polar Biology, 42 (8), 1511–1527. DOI https://doi.org/10.1007/s00300-019-02537-w
Lambert, G., 2009. Adventures of a sea squirt sleuth: unraveling the identity of Didemnum vexillum, a global ascidian invader. Aquatic Invaders, 4(1), 5-28. DOI https://doi.org/10.3391/ai.2009.4.1.2
Lander, T.R., Robinson, S.M., MacDonald, B.A. & Martin, J.D., 2012. Enhanced growth rates and condition index of blue mussels (Mytilus edulis) held at integrated multitrophic aquaculture sites in the Bay of Fundy. Journal of Shellfish Research, 31 (4), 997-1007.
Landes, A., Dolmer, P., Poulsen, L.K., Petersen, J.K. & Vismann, B., 2015. Growth and respiration in blue mussels (Mytilus spp.) from different salinity regimes. Journal of Shellfish Research, 34 (2), 373–382. DOI https://doi.org/10.2983/035.034.0220
Lane, D.J.W., Beaumont, A.R. & Hunter, J.R., 1985. Byssus drifting and the drifting threads of young postlarval mussel Mytilus edulis. Marine Biology, 84, 301-308.
Lang, C. & Mann, K., 1976. Changes in sea urchin populations after the destruction of kelp beds. Marine Biology, 36 (4), 321-326.
Langan R. & Howell W.H., 1994. Growth responses of Mytilus edulis to changes in water flow: A test of the "inhalant pumping speed" hypothesis. Journal of Shellfish Research, 13(1), 289.
Larsen, P.S., Lüskow, F. & Riisgård, H.U., 2018. Too much food may cause reduced growth of blue mussels (Mytilus edulis) - Test of hypothesis and new #&39;high Chl a BEG-model'. Journal of Marine Systems, 180, 299–306. DOI https://doi.org/10.1016/j.jmarsys.2018.01.011
Last, K.S., Hendrick V. J, Beveridge C. M & Davies A. J, 2011. Measuring the effects of suspended particulate matter and smothering on the behaviour, growth and survival of key species found in areas associated with aggregate dredging. Report for the Marine Aggregate Levy Sustainability Fund, Project MEPF 08/P76, 69 pp.
Le Guernic, A., Geffard, A., Le Foll, F. & Ladeiro, M. P., 2020. Y Comparison of viability and phagocytic responses of hemocytes withdrawn from the bivalves Mytilus edulis and Dreissena polymorpha, and exposed to human parasitic protozoa. International Journal for Parasitology, 50 (1), 75–83. DOI https://doi.org/10.1016/j.ijpara.2019.10.005
Le Roux, F., Lorenzo, G., Peyret, P., Audemard, C., Figueras, A., Vivares, C., Gouy, M. & Berthe, F., 2001. Molecular evidence for the existence of two species of Marteilia in Europe. Journal of Eukaryotic Microbiology, 48 (4), 449-454.
Lebrun, A., Miller, C. A., Gazeau, F., Urrutti, P., Alliouane, S., Gattuso, J. P. & Comeau, S., 2025. Tolerance of organisms composing an Arctic kelp community to ocean warming and marine heatwaves. Journal of Ecology. DOI https://doi.org/10.1111/1365-2745.70074
Lebrun, A., Miller, C. A., Meynadier, M., Comeau, S., Urrutti, P., Alliouane, S., Schlegel, R., Gattuso, J. P. & Gazeau, F., 2024. Multifactorial effects of warming, low irradiance, and low salinity on Arctic kelps. Biogeosciences, 21 (20), 4605–4620. DOI https://doi.org/10.5194/bg-21-4605-2024
Legrand, E., Svensen, Ø., Husa, V., Lelièvre, Y. & Svensen, R., 2025. In situ growth dynamics of the invasive ascidian Didemnum vexillum in Norway: Insights from a two-year monitoring study. Marine Pollution Bulletin, 211, 117440. DOI https://doi.org/10.1016/j.marpolbul.2024.117440
Lein, T.E., Sjøtun, K. & Wakili, S., 1991. Mass-occurrence of a brown filamentous endophyte in the lamina of the kelp Laminaria hyperborea (Gunnerus) Foslie along the southwestern coast of Norway. Sarsia, 76 (3), 187-193. DOI https://doi.org/10.1080/00364827.1991.10413474
Leinaas, H.P. & Christie, H., 1996. Effects of removing sea urchins (Strongylocentrotus droebachiensis): stability of the barren state and succession of kelp forest recovery in the east Atlantic. Oecologia, 105(4), 524-536.
Lewis, J.R., 1964. The Ecology of Rocky Shores. London: English Universities Press.
Liénart, C., Garbaras, A., Qvarfordt, S., Sysoev, A.Ö., Höglander, H., Walve, J., Schagerström, E., Eklöf, J. & Karlson, A.M.L., 2021. Long-term changes in trophic ecology of blue mussels in a rapidly changing ecosystem. Limnology and Oceanography, 66 (3), 694–710. DOI https://doi.org/10.1002/lno.11633
Li, C.J., Li, W.T., Liu, J.Y., Zhang, X.M. & Zhang, P.D., 2017. Zostera marina seed burial can be enhanced by manila clam Ruditapes philippinarum: A microcosm Study. Ocean Science Journal, 52 (2), 221–229. DOI https://doi.org/10.1007/s12601-017-0016-5
Li, S.G., Liu, C., Huang, J.L., Liu, Y.J., Zheng, G.L., Xie, L.P. & Zhang, R.Q., 2015. Interactive effects of seawater acidification and elevated temperature on biomineralization and amino acid metabolism in the mussel Mytilus edulis. Journal of Experimental Biology, 218 (22), 3623–3631. DOI https://doi.org/10.1242/jeb.126748
Lindahl, O. & Kollberg, S., 2008. How mussels can improve coastal water quality. Bioscience Explained, 5 (1), 1-14.
Littler, M.M., & Kauker, B.J., 1984. Heterotrichy and survival strategies in the red alga Corallina officinalis L. Botanica Marina, 27, 37-44.
Lobban, C.S. & Harrison, P.J. (eds.), 1994. Seaweed Ecology and Physiology. Cambridge, uk: Cambridge University Press, pp. 366.
Lobban, C.S. & Harrison, P.J., 1997. Seaweed ecology and physiology. Cambridge: Cambridge University Press.
Long, H. A. & Grosholz, E. D., 2015. Overgrowth of eelgrass by the invasive colonial tunicate Didemnum vexillum: Consequences for tunicate and eelgrass growth and epifauna abundance. Journal of Experimental Marine Biology and Ecology, 473, 188-194. DOI https://doi.org/10.1016/j.jembe.2015.08.014
Loo, L-O., 1992. Filtration, assimilation, respiration and growth of Mytilus edulis L. at low temperatures. Ophelia 35: 123-31
Loo, L.-O. & Rosenberg, R., 1983. Mytilus edulisculture: Growth and production in western Sweden. Aquaculture, 35, 137-150.
Loosanoff, V.L., 1962. Effects of turbidity on some larval and adult bivalves. Proceedings of the Gulf and Caribbean Fisheries Institute, 14, 80-95.
Lopez-Flores I., De la Herran, R., Garrido-Ramos, M.A., Navas, J.I., Ruiz-Rejon, C. & Ruiz-Rejon, M., 2004. The molecular diagnosis of Marteilia refringens and differentiation between Marteilia strains infecting oysters and mussels based on the rDNA IGS sequence. Parasitology, 19 (4), 411-419.
Lüning, K., 1990. Seaweeds: their environment, biogeography, and ecophysiology: John Wiley & Sons.
Lutz, R.A. & Kennish, M.J., 1992. Ecology and morphology of larval and early larval postlarval mussels. In The mussel Mytilus: ecology, physiology, genetics and culture, (ed. E.M. Gosling), pp. 53-85. Amsterdam: Elsevier Science Publ. [Developments in Aquaculture and Fisheries Science, no. 25]
Macleod, A., Cottier-Cook, E., Hughes, D. & Allen, C., 2016. Investigating the impacts of marine invasive non-native species. Natural England Commissioned Report NECR223, Natural England, 58 pp. Available from: https://pureadmin.uhi.ac.uk/ws/portalfiles/portal/3729569/NECR223_edition_1.pdf
Maddock, A., 2008. UK Biodiversity Action Plan; Priority Habitat Descriptions. UK Biodiversity Action Plan, 94pp
Mainwaring, K., Tillin, H. & Tyler-Walters, H., 2014. Assessing the sensitivity of blue mussel beds to pressures associated with human activities. Joint Nature Conservation Committee, JNCC Report No. 506., Peterborough, 96 pp. Available from: https://www.marlin.ac.uk/assets/pdf/JNCC_Report_506_web.pdf or http://jncc.defra.gov.uk/pdf/JNCC_Report_506_web.pdf
Mann, K.H., 1982. Kelp, sea urchins, and predators: a review of strong interactions in rocky subtidal systems of eastern Canada, 1970-1980. Netherlands Journal of Sea Research, 16, 414-423.
Mann, R., 1979. Some biochemical and physiological aspects of growth and gametogenesis in Crassostrea gigas and Ostrea edulis grown at sustained elevated temperatures. Journal of the Marine Biological Association of the United Kingdom, 59 (1), 95-110. DOI https://doi.org/10.1017/S0025315400046208
Martins, N., Barreto, L., Bartsch, I., Bernard, J., Serrao, E. A. & Pearson, G. A., 2022. Daylength influences reproductive success and sporophyte growth in the Arctic kelp species Alaria esculenta. Marine Ecology Progress Series, 683, 37–52. DOI https://doi.org/10.3354/meps13950
Matoo, O.B., Lannig, G., Bock, C. & Sokolova, I.M., 2021. Temperature but not ocean acidification affects energy metabolism and enzyme activities in the blue mussel, Mytilus edulis. Ecology and Evolution, 11 (7), 3366–3379. DOI https://doi.org/10.1002/ece3.7289
McGrorty, S., Clarke, R.T., Reading, C.J. & Goss, C.J.D., 1990. Population dynamics of the mussel Mytilus edulis: density changes and regulation of the population in the Exe Estuary, Devon. Marine Ecology Progress Series, 67, 157-169.
McHugh, D.J., 2003. A guide to the seaweed industry: Food and Agriculture Organization of the United Nations Rome.
McKenzie, C.H, Reid, V., Lambert, G., Matheson, K., Minchin, D., Pederson, J., Brown, L., Curd, A., Gollasch, S., Goulletquer, P, Occphipinti-Ambrogi, A., Simard, N. & Therriault, T.W., 2017. Alien species alert: Didemnum vexillum Kott, 2002: Invasion, impact, and control. ICES Cooperative Research Reports (CRR), 33 pp. DOI http://doi.org/10.17895/ices.pub.2138
McKeown, D. A., Stevens, K., Peters, A. F., Bond, P., Harper, G. M., Brownlee, C., Brown, M. T. & Schroeder, D. C., 2017. Phaeoviruses discovered in kelp (Laminariales). The ISME Journal, 11 (12), 2869–2873. DOI https://doi.org/10.1038/ismej.2017.130
McKinstry K. & Jensen A., 2013. Distribution, abundance and temporal variation of the Pacific oyster, Crassostrea gigas in Poole Harbour. Available from: https://assets.publishing.service.gov.uk/government/uploads/system/uploads/attachment_data/file/313003/fcf-oyster.pdf
McNeill, G., Nunn, J. & Minchin, D., 2010. The slipper limpet Crepidula fornicata Linnaeus, 1758 becomes established in Ireland. Aquatic Invasions, 5 (Suppl. 1), S21-S25. DOI https://doi.org/10.3391/ai.2010.5.S1.006
Melville, A. & Connell, S., 2001. Experimental effects of kelp canopies on subtidal coralline algae. Austral Ecology, 26 (1), 102-108.
Melzner, F., Buchholz, B., Wolf, F., Panknin, U. & Wall, M., 2020. Ocean winter warming induced starvation of predator and prey. Proceedings of the Royal Society B-Biological Sciences, 287 (1931). DOI https://doi.org/10.1098/rspb.2020.0970
Melzner, F., Stange, P., Trübenbach, K., Thomsen, J., Casties, I., Panknin, U., Gorb, S.N. & Gutowska, M.A., 2011. Food Supply and Seawater pCO2 Impact Calcification and Internal Shell Dissolution in the Blue Mussel Mytilus edulis. PLOS ONE, 6 (9), e24223. DOI https://doi.org/10.1371/journal.pone.0024223
Mercer, J.M, Whitlatch, R.B, & Osman, R.W. 2009. Potential effects of the invasive colonial ascidian (Didemnum vexillum Kott, 2002) on pebble-cobble bottom habitats in Long Island Sound, USA. Aquatic Invasions, 4, 133-142. DOI https://doi.org/10.3391/ai.2009.4.1.14
Met Office, 2016. Southern England: climate. https://www.metoffice.gov.uk/binaries/content/assets/metofficegovuk/pdf/weather/learn-about/uk-past-events/regional-climates/southern-england_-climate---met-office.pdf
Metcalf, 2019. The disappearance of Mytilus edulis in the Gulf of Maine. Gulf of Maine Institute. Available from: https://www.gulfofmaineinstitute.org/single-post/2019/10/11/-the-disappearance-of-mytilus-edulis-in-the-gulf-of-maine
Mieszkowska, N., 2016. Chapter 14 - Intertidal Indicators of Climate and Global Change. In Letcher, T.M. (ed.) Climate Change (Second Edition), Boston: Elsevier, pp. 213-229.
Mieszkowska, N., Leaper, R., Moore, P., Kendall, M., Burrows, M., Lear, D., Poloczanska, E., Hiscock, K., Moschella, P. & Thompson, R., 2005. Marine Biodiversity and Climate Change (MarClim) Assessing and predicting the influence of climatic change using intertidal rocky shore biota. Final Report for United Kingdom Funders. Marine Biological Association Occasional Publications, 20, 53p.
Miller III, H.L., Neale, P.J. & Dunton, K.H., 2009. Biological weighting functions for UV inhibtion of photosynthesis in the kelp Laminaria hyperborea (Phaeophyceae) 1. Journal of Phycology, 45 (3), 571-584.
Minchin, D. & Nunn, J., 2014. The invasive brown alga Undaria pinnatifida (Harvey) Suringar, 1873 (Laminariales: Alariaceae), spreads northwards in Europe. Bioinvasions Records, 3 (2), 57-63. DOI http://dx.doi.org/10.3391/bir.2014.3.2.01
Minchin, D.M & Nunn, J.D., 2013. Rapid assessment of marinas for invasive alien species in Northern Ireland. Northern Ireland Environment Agency Research and Development Series, Northern Ireland Environment Agency.
Moore, P.G., 1973a. The kelp fauna of north east Britain I. Function of the physical environment. Journal of Experimental Marine Biology and Ecology, 13, 97-125.
Moore, P.G., 1973b. The kelp fauna of north east Britain. II. Multivariate classification: turbidity as an ecological factor. Journal of Experimental Marine Biology and Ecology, 13, 127-163.
Moore, P.G., 1978. Turbidity and kelp holdfast Amphipoda. I. Wales and S.W. England. Journal of Experimental Marine Biology and Ecology, 32, 53-96.
Moore, P.G., 1985. Levels of heterogeneity and the amphipod fauna of kelp holdfasts. In The Ecology of Rocky Coasts: essays presented to J.R. Lewis, D.Sc. (ed. P.G. Moore & R. Seed), 274-289. London: Hodder & Stoughton Ltd.
Morgan, A., Slater, M., Mortimer, N., McNie, F., Singfield, C., Bailey, L., Covey, R., McNair, S., Waddell, C., Crundwell, R., Gall, A., Selley, H. & Packer, N., 2021. Partnership led strategy to monitor and manage spread of Pacific oyster populations in south Devon and Cornwall. Natural England Research Reports, NERR100. Natural England Research Reports, NERR100, Natural England, Truro, Cornwall, 258 pp. Available from: https://publications.naturalengland.org.uk/publication/4889256448491520#:~:text=Between 2017 and 2020, volunteers,method of controlling population expansion.
Moyse, E., Firth, L. B., Smyth, T. & Davies, T.W., 2025. Artificial light at night alters seaweed reproductive phenology. Environmental Pollution, 385, 127155. DOI https://doi.org/10.1016/j.envpol.2025.127155
Munda, I.M. & Luning, K., 1977. Growth performance of Alaria esculenta off Helgoland. Helgolander Wissenschaftliche Meeresuntersuchungen, 29, 311-314.
Murúa, P., Küpper, F. C., Muñoz, L. A., Bernard, M. & Peters, A. F., 2018. Microspongium alariae in Alaria esculenta: a widely-distributed non-parasitic brown algal endophyte that shows cell modifications within its host. Botanica Marina, 61 (4), 343–354. DOI https://doi.org/doi:10.1515/bot-2017-0095
Murray, F., De Clippele, L.H., Hiley, A., Wicks, L., Roberts, J.M. & Hennige, S., 2019. Multiple feeding strategies observed in the cold-water coral Lophelia pertusa. Journal of the Marine Biological Association of the United Kingdom, 99 (6), 1281-1283. DOI https://doi.org/10.1017/s0025315419000298
Myrand, B., Guderley, H. & Himmelman, J.H., 2000. Reproduction and summer mortality of blue mussels Mytilus edulis in the Magdalen Islands, southern Gulf of St. Lawrence. Marine Ecology Progress Series 197: 193-207
Nascimento-Schulze, J.C., Vajedsamiei, J., Bean, T.P., Frankholz, L., Brennan, R.S., Melzner, F. & Ellis, R.P., 2025. Thermal selection shifts genetic diversity and performance in blue mussel juveniles. Evolutionary Applications, 18 (6). DOI https://doi.org/10.1111/eva.70118
NBN, 2015. National Biodiversity Network 2015(20/05/2015).https://data.nbn.org.uk/
NBN, 2024. National Biodiversity Network 2024(20/05/2024).https://data.nbn.org.uk/
Nehls, G. & Thiel, M., 1993. Large-scale distribution patterns of the mussel Mytilus edulis in the Wadden Sea of Schleswig-Holstein: Do storms structure the ecosystems? Netherlands Journal of Sea Research, 31, 181-187.
Nehls, G., Diederich, S., Thieltges, David W. & Strasser, M., 2006. Wadden Sea mussel beds invaded by oysters and slipper limpets: competition or climate control? Helgoland Marine Research, 60 (2), 135-143. DOI https://doi.org/10.1007/s10152-006-0032-9
Nenonen, N.P., Hannoun, C., Horal, P., Hernroth, B. & Bergström, T., 2008. Tracing of norovirus outbreak strains in mussels collected near sewage effluents. Applied and Environmental Microbiology, 74 (8), 2544-2549.
Netalgae, 2012. Seaweed industry in Europe. http://www.netalgae.eu/publications.php: (24/04/2014).
Nichols, D., 1981. The Cornish Sea-urchin Fishery. Cornish Studies, 9, 5-18.
Nielsen, M.B., Vogensen, T.K., Thyrring, J., Sorensen, J.G. & Sejr, M.K., 2021. Freshening increases the susceptibility to heat stress in intertidal mussels (Mytilus edulis) from the Arctic. Journal of Animal Ecology, 90 (6), 1515–1524. DOI https://doi.org/10.1111/1365-2656.13472
Nippard, L. & Ciocan, C., 2019. Potential impact of aquaculture effluents in Loch Creran, Scotland. Vie Et Milieu-Life and Environment, 69 (1), 47–52. DOI https://doi.org/10.57890/pn0gv585
Norderhaug, K., 2004. Use of red algae as hosts by kelp-associated amphipods. Marine Biology, 144 (2), 225-230.
Norderhaug, K.M. & Christie, H.C., 2009. Sea urchin grazing and kelp re-vegetation in the NE Atlantic. Marine Biology Research, 5 (6), 515-528.
Norderhaug, K.M., Christie, H. & Fredriksen, S., 2007. Is habitat size an important factor for faunal abundances on kelp (Laminaria hyperborea)? Journal of Sea Research, 58 (2), 120-124.
Nordheim, van, H., Andersen, O.N. & Thissen, J., 1996. Red lists of Biotopes, Flora and Fauna of the Trilateral Wadden Sea area, 1995. Helgolander Meeresuntersuchungen, 50 (Suppl.), 1-136.
Norton, T.A., 1992. Dispersal by macroalgae. British Phycological Journal, 27, 293-301.
Norton, T.A., Hiscock, K. & Kitching, J.A., 1977. The Ecology of Lough Ine XX. The Laminaria forest at Carrigathorna. Journal of Ecology, 65, 919-941.
Nunes, J., McCoy, S.J., Findlay, H.S., Hopkins, F.E., Kitidis, V., Queirós, A.M., Rayner, L. & Widdicombe, S., 2016. Two intertidal, non-calcifying macroalgae (Palmaria palmata and Saccharina latissima) show complex and variable responses to short-term CO2 acidification. ICES Journal of Marine Science, 73 (3), 887-896. DOI https://doi.org/10.1093/icesjms/fsv081
O'Brien, P.J. & Dixon, P.S., 1976. Effects of oils and oil components on algae: a review. British Phycological Journal, 11, 115-142.
OBIS (Ocean Biodiversity Information System), 2026. OBIS (Ocean Biodiversity Information System). Available from: www.iobis.org
Oliveira, G.F., Siregar, H., Queiroga, H. & Peteiro, L.G., 2021. Main drivers of fecundity variability of mussels along a latitudinal gradient: Lessons to apply for future climate change scenarios. Journal of Marine Science and Engineering, 9 (7). DOI https://doi.org/10.3390/jmse9070759
Padilla, D.K., 2010. Context-dependent impacts of a non-native ecosystem engineer, the Pacific Oyster Crassostrea gigas. Integrative and Comparative Biology, 50 (2), 213-225. DOI https://doi.org/10.1093/icb/icq080
Page, H. & Hubbard, D., 1987. Temporal and spatial patterns of growth in mussels Mytilus edulis on an offshore platform: relationships to water temperature and food availability. Journal of Experimental Marine Biology and Ecology 111: 159-79
Paine, R.T. & Levin, S.A., 1981. Intertidal landscapes: disturbance and the dynamics of pattern. Ecological Monographs, 51, 145-178.
Park, J., Kim, J., Kong, J.-A., Depuydt, S., Brown, M. & Han, T., 2017. Implications of rising temperatures for gametophyte performance of two kelp species from Arctic waters. Botanica Marina, 60. DOI http://doi.org/10.1515/bot-2016-0103
Parke, M., 1948. Studies on British Laminariaceae. I. Growth in Laminaria saccharina (L.) Lamour. Journal of the Marine Biological Association of the United Kingdom, 27, 651-709.
Parry, H., & Pipe, R., 2004. Interactive effects of temperature and copper on immunocompetence and disease susceptibility in mussels (Mytilus edulis). Aquatic Toxicology 69: 311-25
Pearce, J.B., 1969. Thermal addition and the benthos, Cape Cod Canal. Chesapeake Science, 10 (3), 227-233. DOI https://doi.org/10.2307/1350459
Pedersen, M.F., Nejrup, L.B., Fredriksen, S., Christie, H. & Norderhaug, K.M., 2012. Effects of wave exposure on population structure, demography, biomass and productivity of the kelp Laminaria hyperborea. Marine Ecology Progress Series, 451, 45-60.
Penfold, R., Hughson, S., & Boyle, N., 1996. The potential for a sea urchin fishery in Shetland. http://www.nafc.ac.uk/publish/note5/note5.htm, 2000-04-14
Pereira, T.R., Engelen, A.H., Pearson, G.A., Valero, M. & Serrao, E.A., 2017. Population dynamics of temperate kelp forests near their low-latitude limit. Aquatic Botany, 139, 8–18. DOI https://doi.org/10.1016/j.aquabot.2017.02.006
Pérez, R., 1971. Écologie, croissance et régénération, teneurs en acide alginique de Laminaria digitata sur les cotes de la Manche. Revue des Travaux de l'Institut des Peches Maritimes, 35, 287-346.
Perry, M. & Golding, N., 2011. Range of environmental temperature conditions in the United Kingdom Met Office, Exeter, UK, 64 pp. pp.
Philippart, C.J., Anadón, R., Danovaro, R., Dippner, J.W., Drinkwater, K.F., Hawkins, S.J., Oguz, T., O'Sullivan, G. & Reid, P.C., 2011. Impacts of climate change on European marine ecosystems: observations, expectations and indicators. Journal of Experimental Marine Biology and Ecology, 400 (1), 52-69.
Picard, M. M. M., Johnson, L. E. & Côté, I. M., 2022. Effects of sediment on spore performance as a potential constraint on kelp distribution. Marine Pollution Bulletin, 185, 114336. DOI https://doi.org/10.1016/j.marpolbul.2022.114336
Powell-Jennings, C. & Callaway, R., 2018. The invasive, non-native slipper limpet Crepidula fornicata is poorly adapted to sediment burial. Marine Pollution Bulletin, 130, 95-104. DOI https://doi.org/10.1016/j.marpolbul.2018.03.006
Preston, J., Fabra, M., Helmer, L., Johnson, E., Harris-Scott, E. & Hendy, I.W., 2020. Interactions of larval dynamics and substrate preference have ecological significance for benthic biodiversity and Ostrea edulis Linnaeus, 1758 in the presence of Crepidula fornicata. Aquatic Conservation: Marine and Freshwater Ecosystems, 30 (11), 2133-2149. DOI https://doi.org/10.1002/aqc.3446
Price, H., 1982. An analysis of factors determining seasonal variation in the byssal attachment strength of Mytilus edulis. Journal of the Marine Biological Association of the United Kingdom, 62 (01), 147-155
Purchon, R.D., 1937. Studies on the biology of the Bristol Channel. Proceedings of the Bristol Naturalists' Society, 8, 311-329.
Raffaelli, D.G. & Hawkins, S.J., 1999. Intertidal Ecology 2nd edn.. London: Kluwer Academic Publishers.
Ramsay, K., Kaiser, M.J. & Hughes, R.N. 1998. The responses of benthic scavengers to fishing disturbance by towed gears in different habitats. Journal of Experimental Marine Biology and Ecology, 224, 73-89.
Rankin, C.J. & Davenport, J.A., 1981. Animal Osmoregulation. Glasgow & London: Blackie. [Tertiary Level Biology].
Read, K.R.H. & Cumming, K.B., 1967. Thermal tolerance of the bivalve molluscs Modiolus modiolus (L.), Mytilus edulis (L.) and Brachidontes demissus (Dillwyn). Comparative Biochemistry and Physiology, 22, 149-155.
Reichwaldt, E. S. & Ghadouani, A., 2016. Can mussels be used as sentinel organisms for characterization of pollution in urban water systems?. Hydrology and Earth System Sciences, 20 (7), 2679–2689. DOI http://doi.org/10.5194/hess-20-2679-2016
Reise, K., Buschbaum, C., Dolch, T., van Beusekom, J.E.E. & Wegner, K.M., 2025. Benthic losers and winners in a tidal bay since the 1920s. Marine Biodiversity, 55 (5). DOI https://doi.org/10.1007/s12526-025-01566-5
Richardson, S., Crook, A. & Fitzsimmons, C., 2021. An investigation into the drivers of Mytilus edulis decline within Northumberland Marine Special Protected Area. Masters Thesis, Newcastle University.
Ricklefs, K., Büttger, H. & Asmus, H., 2020. Occurrence, stability, and associated species of subtidal mussel beds in the North Frisian Wadden Sea (German North Sea Coast). Estuarine Coastal and Shelf Science, 233. DOI https://doi.org/10.1016/j.ecss.2019.106549
Riisgård, H.U., Lüskow, F., Pleissner, D., Lundgreen, K. & López, M., 2013. Effect of salinity on filtration rates of mussels Mytilus edulis with special emphasis on dwarfed mussels from the low-saline Central Baltic Sea. Helgoland Marine Research, 67, 591-8
Rinde, E. & Sjøtun, K., 2005. Demographic variation in the kelp Laminaria hyperborea along a latitudinal gradient. Marine Biology, 146 (6), 1051-1062.
Roberts, J.M., 2009. Cold-water corals: the biology and geology of deep-sea coral habitats. Cambridge University Press, Cambridge.
Roberts, L., Cheesman, S., Breithaupt, T. and Elliott, M., 2015. Sensitivity of the mussel Mytilus edulis to substrate‑borne vibration in relation to anthropogenically generated noise. Marine Ecology Progress Series, 538, 185-195.
Robledo, J.A.F., Santarem, M.M., Gonzalez, P. & Figueras, A., 1995. Seasonal variations in the biochemical composition of the serum of Mytilus galloprovincialis Lmk. and its relationship to the reproductive cycle and parasitic load. Aquaculture, 133 (3-4), 311-322.
Rogers-Bennett, L. & Catton, C.A., 2019. Marine heatwave and multiple stressors tip bull kelp forest to sea urchin barrens. Scientific Reports, 9 (1), 15050. DOI https://doi.org/10.1038/s41598-019-51114-y
Roleda, M. Y., Marfaing, H., Desnica, N., Jónsdóttir, R., Skjermo, J., Rebours, C. & Nitschke, U., 2019. Variations in polyphenol and heavy metal contents of wild-harvested and cultivated seaweed bulk biomass: Health risk assessment and implication for food applications. Food Control, 95, 121–134. DOI https://doi.org/10.1016/j.foodcont.2018.07.031
Roleda, M.Y., Morris, J.N., McGraw, C.M. & Hurd, C.L., 2012. Ocean acidification and seaweed reproduction: increased CO2 ameliorates the negative effect of lowered pH on meiospore germination in the giant kelp Macrocystis pyrifera (Laminariales, Phaeophyceae). Global Change Biology, 18 (3), 854-864. DOI https://doi.org/10.1111/j.1365-2486.2011.02594.x
Ronowicz, M., Kukliński, P. & Włodarska-Kowalczuk, M., 2018. Diversity of kelp holdfast-associated fauna in an Arctic fjord - inconsistent responses to glacial mineral sedimentation across different taxa. Estuarine, Coastal and Shelf Science, 205, 100–109. DOI https://doi.org/10.1016/j.ecss.2018.01.024
Ronowicz, M., Kukliński, P. & Włodarska-Kowalczuk, M., 2022. Morphological variation of kelps (Alaria esculenta, cf. Laminaria digitata, and Saccharina latissima) in an Arctic glacial fjord. Estuarine, Coastal and Shelf Science, 268, 107802. DOI https://doi.org/10.1016/j.ecss.2022.107802
Rosa, M., Capriotti, M., Austin, K., Shumway, S.E. & Ward, J.E., 2024. Effect of seasonal changes in temperature on capture efficiency in the blue mussel, Mytilus edulis, fed seston and microplastics. Invertebrate Biology, 143 (4). DOI https://doi.org/10.1111/ivb.12446
Rostron, D.M. & Bunker, F. St P.D., 1997. An assessment of sublittoral epibenthic communities and species following the Sea Empress oil spill. A report to the Countryside Council for Wales from Marine Seen & Sub-Sea Survey., Countryside Council for Wales, Bangor, CCW Sea Empress Contact Science, no. 177.
Saier, B., 2002. Subtidal and intertidal mussel beds (Mytilus edulis L.) in the Wadden Sea: diversity differences of associated epifauna. Helgoland Marine Research, 56, 44-50
Sawabe, T., Makino, H., Tatsumi, M., Nakano, K., Tajima, K., Iqbal, M.M., Yumoto, I., Ezura, Y. & Christen, R., 1998. Pseudoalteromonas bacteriolytica sp. nov., a marine bacterium that is the causative agent of red spot disease of Laminaria japonica. International Journal of Systematic Bacteriology, 48 (3), 769-774.
Schiel, D.R. & Foster, M.S., 1986. The structure of subtidal algal stands in temperate waters. Oceanography and Marine Biology: an Annual Review, 24, 265-307.
Schiel, D.R. & Taylor, D.I., 1999. Effects of trampling on a rocky intertidal algal assemblage in southern New Zealand. Journal of Experimental Marine Biology and Ecology, 235, 213-235.
Schoenrock, K.M., O’Callaghan, T., O’Callaghan, R. & Krueger-Hadfield, S.A., 2019. First record of Laminaria ochroleuca Bachelot de la Pylaie in Ireland in Béal an Mhuirthead, county Mayo. Marine Biodiversity Records, 12 (1), 9. DOI https://doi.org/10.1186/s41200-019-0168-3
Seapy , R.R. & Littler, M.M., 1982. Population and Species Diversity Fluctuations in a Rocky Intertidal Community Relative to Severe Aerial Exposure and Sediment Burial. Marine Biology, 71, 87-96.
Seed R., 1969. The ecology of Mytilus edulis L.(Lamellibranchiata) on exposed rocky shores. Oecologia, 3, 277-316.
Seed, R. & Suchanek, T.H., 1992. Population and community ecology of Mytilus. In The mussel Mytilus: ecology, physiology, genetics and culture, (ed. E.M. Gosling), pp. 87-169. Amsterdam: Elsevier Science Publ. [Developments in Aquaculture and Fisheries Science, no. 25.]
Seuront, L., Nicastro, K.R., Zardi, G.I. & Goberville, E., 2019. Decreased thermal tolerance under recurrent heat stress conditions explains summer mass mortality of the blue mussel Mytilus edulis. Scientific reports, 9 (1), 17498. DOI https://doi.org/10.1038/s41598-019-53580-w
Sheppard, C.R.C., Bellamy, D.J. & Sheppard, A.L.S., 1980. Study of the fauna inhabiting the holdfasts of Laminaria hyperborea (Gunn.) Fosl. along some environmental and geographical gradients. Marine Environmental Research, 4, 25-51.
Shumway, S.E., 1990. A review of the effects of algal blooms on shellfish and aquaculture. Journal of the World Aquaculture Society, 21, 65-104.
Silva, C. F., Pearson, G. A., Serrão, E. A., Bartsch, I. & Martins, N., 2022. Microscopic life stages of Arctic kelp differ in their resilience and reproductive output in response to Arctic seasonality. European Journal of Phycology, 57 (4), 381–395. DOI https://doi.org/10.1080/09670262.2021.2014983
Sivertsen, K., 1997. Geographic and environmental factors affecting the distribution of kelp beds and barren grounds and changes in biota associated with kelp reduction at sites along the Norwegian coast. Canadian Journal of Fisheries and Aquatic Sciences, 54, 2872-2887.
Sjøtun, K., Christie, H. & Helge Fosså, J., 2006. The combined effect of canopy shading and sea urchin grazing on recruitment in kelp forest (Laminaria hyperborea). Marine Biology Research, 2 (1), 24-32.
Sjøtun, K. & Schoschina, E.V., 2002. Gametophytic development of Laminaria spp. (Laminariales, Phaeophyta) at low temperatures. Phycologia, 41, 147-152.
Smaal, A. C., Kater, B. J. & Wijsman, J., 2009. Introduction, establishment and expansion of the Pacific oyster Crassostrea gigas in the Oosterschelde (SW Netherlands). Helgoland Marine Research, 63 (1), 75-83. DOI https://doi.org/10.1007/s10152-008-0138-3
Smaal, A.C. & Twisk, F., 1997. Filtration and absorption of Phaeocystis cf. globosa by the mussel Mytilus edulis L. Journal of Experimental Marine Biology and Ecology, 209, 33-46
Smale, D.A. & Vance, T., 2015. Climate-driven shifts in species’ distributions may exacerbate the impacts of storm disturbances on North-east Atlantic kelp forests. Marine and Freshwater Research, 67 (1), 65-74. DOI https://doi.org/10.1071/MF14155
Smale, D.A., 2020. Impacts of ocean warming on kelp forest ecosystems. New Phytologist, 225, 1447-1454. DOI https://doi.org/10.1111/nph.16107
Smale, D.A., Burrows, M.T., Evans, A.J., King, N., Sayer, M.D.J., Yunnie, A.L.E. & Moore, P.J., 2016. Linking environmental variables with regional-scale variability in ecological structure and standing stock of carbon within UK kelp forests. Marine Ecology Progress Series, 542, 79–95. DOI https://doi.org/10.3354/meps11544
Smale, D.A., Burrows, M.T., Moore, P., O'Connor, N. & Hawkins, S.J., 2013. Threats and knowledge gaps for ecosystem services provided by kelp forests: a northeast Atlantic perspective. Ecology and evolution, 3 (11), 4016-4038.
Smale, D.A., Wernberg, T., Yunnie, A.L. & Vance, T., 2014. The rise of Laminaria ochroleuca in the Western English Channel (UK) and comparisons with its competitor and assemblage dominant Laminaria hyperborea. Marine ecology.
Smale, D.A., Wernberg, T., Yunnie, A.L.E. & Vance, T., 2015. The rise of Laminaria ochroleuca in the Western English Channel (UK) and comparisons with its competitor and assemblage dominant Laminaria hyperborea. Marine Ecology, 36 (4), 1033-1044. DOI https://doi.org/10.1111/maec.12199
Smith, J.E. (ed.), 1968. 'Torrey Canyon'. Pollution and marine life. Cambridge: Cambridge University Press.
Smith, J.R. & Murray, S.N., 2005. The effects of experimental bait collection and trampling on a Mytilus californianus mussel bed in southern California. Marine Biology, 147, 699-706
Smyth, T. J., Wright, A. E., McKee, D., Tidau, S., Tamir, R., Dubinsky, Z., Iluz, D. & Davies, T. W., 2021. A global atlas of artificial light at night under the sea. Elementa: Science of the Anthropocene, 9 (1). DOI https://doi.org/10.1525/elementa.2021.00049
Sokolov, E.P., Adzigbli, L., Markert, S., Bundgaard, A., Fago, A., Becher, D., Hirschfeld, C. & Sokolova, I.M., 2021. Intrinsic mechanisms underlying hypoxia-tolerant mitochondrial phenotype during hypoxia-reoxygenation stress in a marine facultative anaerobe, the blue mussel Mytilus edulis. Frontiers in Marine Science, 8. DOI https://doi.org/10.3389/fmars.2021.773734
Somerfield, P.J. & Warwick, R.M., 1999. Appraisal of environmental impact and recovery using Laminaria holdfast faunas. Sea Empress, Environmental Evaluation Committee., Countryside Council for Wales, Bangor, CCW Sea Empress Contract Science, Report no. 321.
Sorte, C.J.B., Davidson, V.E., Franklin, M.C., Benes, K.M., Doellman, M.M., Etter, R.J., Hannigan, R.E., Lubchenco, J. & Menge, B.A., 2017. Long-term declines in an intertidal foundation species parallel shifts in community composition. Global Change Biology, 23 (1), 341–352. DOI https://doi.org/10.1111/gcb.13425
Spencer, B. E., Edwards, D. B., Kaiser, M. J. & Richardson, C. A., 1994. Spatfalls of the non-native Pacific oyster, Crassostrea gigas, in British waters. Aquatic Conservation: Marine and Freshwater Ecosystems, 4 (3), 203-217. DOI https://doi.org/10.1002/aqc.3270040303
Spiga, I., Caldwell, G.S. & Bruintjes, R., 2016. Influence of pile driving on the clearance rate of the blue mussel, Mytilus edulis (L.). Proceedings of Meetings on Acoustics, 27 (1). DOI https://doi.org/10.1121/2.0000277
Staehr, P.A. & Wernberg, T., 2009. Physiological responses of Ecklonia radiata (Laminariales) to a latitudinal gradient in ocean temperature. Journal of Phycology, 45, 91-99.
Staehr, P.A., Pedersen, M.F., Thomsen, M.S., Wernberg, T. & Krause-Jensen, D., 2000. Invasion of Sargassum muticum in Limfjorden (Denmark) and its possible impact on the indigenous macroalgal community. Marine Ecology Progress Series, 207, 79-88. DOI https://doi.org/10.3354/meps207079
Stagličić, N., Segvic-Bubic, T., Ezgeta-Balic, D., Varezic, D. B., Grubisic, L., Zuvic, L., Lin, Y. P. & Briski, E., 2020. Distribution patterns of two co-existing oyster species in the northern Adriatic Sea: The native European flat oyster Ostrea edulis and the non-native Pacific oyster Magallana gigas. Ecological Indicators, 113. DOI https://doi.org/10.1016/j.ecolind.2020.106233
Stefaniak, L., Zhang, H., Gittenberger, A., Smith, K., Holsinger, K., Lin, S. & Whitlatch, R.B., 2012. Determining the native region of the putatively invasive ascidian Didemnum vexillum Kott, 2002. Journal of Experimental Marine Biology and Ecology, 422-423, 64-71. DOI https://doi.org/10.1016/j.jembe.2012.04.012
Steffen, J.B.M., Falfushynska, H.I., Piontkivska, H. & Sokolova, I.M., 2020. Molecular biomarkers of the mitochondrial quality control are differently affected by hypoxia-reoxygenation stress in marine bivalves Crassostrea gigas and Mytilus edulis. Frontiers in Marine Science, 7. DOI https://doi.org/10.3389/fmars.2020.604411
Steneck, R.S., Graham, M.H., Bourque, B.J., Corbett, D., Erlandson, J.M., Estes, J.A. & Tegner, M.J., 2002. Kelp forest ecosystems: biodiversity, stability, resilience and future. Environmental conservation, 29 (04), 436-459.
Steneck, R.S., Vavrinec, J. & Leland, A.V., 2004. Accelerating trophic-level dysfunction in kelp forest ecosystems of the western North Atlantic. Ecosystems, 7 (4), 323-332.
Stiger-Pouvreau, V. & Thouzeau, G., 2015. Marine Species Introduced on the French Channel-Atlantic Coasts: A Review of Main Biological Invasions and Impacts. Open Journal of Ecology, 5, 227-257. DOI https://doi.org/10.4236/oje.2015.55019
Strong, J.A. & Dring, M.J., 2011. Macroalgal competition and invasive success: testing competition in mixed canopies of Sargassum muticum and Saccharina latissima. Botanica Marina, 54 (3), 223-229.
Suchanek, T.H., 1978. The ecology of Mytilus edulis L. in exposed rocky intertidal communities. Journal of Experimental Marine Biology and Ecology, 31, 105-120.
Suchanek, T.H., 1985. Mussels and their role in structuring rocky shore communities. In The Ecology of Rocky Coasts: essays presented to J.R. Lewis, D.Sc., (ed. P.G. Moore & R. Seed), pp. 70-96.
- Sun, T., Tang, X., Jiang, Y. & Wang, Y., 2017. Seawater acidification induced immune function changes of haemocytes in Mytilus edulis: a comparative study of CO2 and HCl enrichment. Scientific Reports, 7 (1), 41488. DOI https://doi.org/10.1038/srep41488
Sundene, O., 1962. The implications of transplant and culture experiments on the growth and distribution of Alaria esculenta. Nytt Magasin for Botanik, 9, 155-174.
Tagliapietra, D., Keppel, E., Sigovini, M. & Lambert, G., 2012. First record of the colonial ascidian Didemnum vexillum Kott, 2002 in the Mediterranean: Lagoon of Venice (Italy). Bioinvasions Records, 1 (4), 247-254. DOI http://dx.doi.org/10.3391/bir.2012.1.4.02
Talevi, J., Steeves, L., Coffin, M., Guyondet, T., Sakamaki, T., Comeau, L. & Filgueira, R., 2023. The physiological state of four commercially important bivalve species during a naturally occurring heatwave. Canadian Journal of Zoology, 101 (10), 913–929. DOI https://doi.org/10.1139/cjz-2022-0215
Tang, B.J. & Riisgård, H.U., 2018. Relationship between oxygen concentration, respiration and filtration rate in blue mussel Mytilus edulis. Journal of Oceanology and Limnology, 36 (2), 395–404. DOI https://doi.org/10.1007/s00343-018-6244-4
Tangen K., 1977. Blooms of Gyrodinium aureolum (Dinophygeae) in North European waters, accompanied by mortality in marine organisms. Sarsia, 6 , 123-33.
Taylor-Robinson, C., King, N.G., Foggo, A. & Smale, D.A., 2024. Spatiotemporal variability in the population demography of the golden kelp, Laminaria ochroleuca (Phaeophyceae), at its leading range edge. European Journal of Phycology, 60 (1), 24–34. DOI https://doi.org/10.1080/09670262.2024.2433471
Teagle, H., Hawkins, S. J., Moore, P. J. & Smale, D. A., 2017. The role of kelp species as biogenic habitat formers in coastal marine ecosystems. Journal of Experimental Marine Biology and Ecology, 492, 81-98. DOI https://doi.org/10.1016/j.jembe.2017.01.017
Telesca, L., Peck, L.S., Backeljau, T., Heinig, M.F. & Harper, E.M., 2021. A century of coping with environmental and ecological changes via compensatory biomineralization in mussels. Global Change Biology, 27 (3), 624–639. DOI https://doi.org/10.1111/gcb.15417
Terry, C. E., Liebzeit, J. A., Purvis, E. M. & Dowd, W. W., 2024. Interactive effects of temperature and salinity on metabolism and activity of the copepod Tigriopus californicus. Journal of Experimental Biology, 227 (17). DOI https://doi.org/10.1242/jeb.248040
Teschke, K., Karez, R., Schubert, P. R. & Beermann, J., 2020. Colonisation success of introduced oysters is driven by wave-related exposure. Biological Invasions, 22 (7), 2121-2127. DOI https://doi.org/10.1007/s10530-020-02246-0
Theisen, B.F., 1982. Variation in size of gills, labial palps, and adductor muscle in Mytilus edulis L. (Bivalvia) from Danish waters. Ophelia, 21 (1), 49-63.
Thieltges, D.W., Strasser, M. & Reise, K., 2003. The American slipper-limpet Crepidula fornicata (L.) in the Northern Wadden Sea 70 years after its introduction. Helgoland Marine Research, 57, 27-33
Thieltges, D.W., Strasser, M., Van Beusekom, J.E. & Reise, K., 2004. Too cold to prosper—winter mortality prevents population increase of the introduced American slipper limpet Crepidula fornicata in northern Europe. Journal of Experimental Marine Biology and Ecology, 311 (2), 375-391. DOI https://doi.org/10.1016/j.jembe.2004.05.018
Thomas, Y. & Bacher, C., 2018. Assessing the sensitivity of bivalve populations to global warming using an individual-based modelling approach. Global Change Biology, 24 (10), 4581–4597. DOI https://doi.org/10.1111/gcb.14402
Thomas, Y., Razafimahefa, N.R., Ménesguen, A. & Bacher, C., 2020. Multi-scale interaction processes modulate the population response of a benthic species to global warming. Ecological Modelling, 436. DOI https://doi.org/10.1016/j.ecolmodel.2020.109295
Thompson, G.A. & Schiel, D.R., 2012. Resistance and facilitation by native algal communities in the invasion success of Undaria pinnatifida. Marine Ecology, Progress Series, 468, 95-105.
Thompson, I., Richardson, C., Seed R. & Walker G., 2000. Quantification of mussel (Mytilus edulis) growth from power station cooling waters in response to chlorination procedures. Biofouling, 16(1), 1-15.
Thyrring, J., Rysgaard, S., Blicher, M.E. & Sejr, M.K., 2015. Metabolic cold adaptation and aerobic performance of blue mussels (Mytilus edulis) along a temperature gradient into the High Arctic region. Marine Biology, 162 (1), 235–243. DOI https://doi.org/10.1007/s00227-014-2575-7
Thyrring, J., Tremblay, R. & Sejr, M.K., 2019. Local cold adaption increases the thermal window of temperate mussels in the Arctic. Conservation Physiology, 7. DOI https://doi.org/10.1093/conphys/coz098
Tidau, S., Brough, F.T., Gimenez, L., Jenkins, S.R. & Davies, T.W., 2023. Impacts of artificial light at night on the early life history of two ecosystem engineers. Philosophical Transactions of the Royal Society B-Biological Sciences, 378 (1892). DOI https://doi.org/10.1098/rstb.2022.0363
Tidbury, H, 2020. Wakame (Undaria pinnatifida). GB Non-native Species Rapid Risk Assessment., 15 pp. Available from: http://www.nonnativespecies.org/index.cfm?pageid=143
Tracey, G.A., 1988. Effects of inorganic and organic nutrient enrichment on growth and bioenergetics of the blue mussel, Mytilus edulis. Journal of Shelfish Research, 7, 562.
Tran, D., Andrade, H., Durier, G., Ciret, P., Leopold, P., Sow, M., Ballantine, C., Camus, L., Berge, J. & Perrigault, M., 2020. Growth and behaviour of blue mussels, a re-emerging polar resident, follow a strong annual rhythm shaped by the extreme high Arctic light regime. Royal Society Open Science, 7 (10). DOI https://doi.org/10.1098/rsos.200889
Tremblay, R., Myrand, B., Sevigny, J.-M., Blier, P. & Guderley, H., 1998. Bioenergetic and genetic parameters in relation to susceptibility of blue mussels, Mytilus edulis (L.) to summer mortality. Journal of Experimental Marine Biology and Ecology, 221 (1), 27-58. DOI https://doi.org/10.1016/S0022-0981(97)00114-7
Troost, K., 2010. Causes and effects of a highly successful marine invasion: case-study of the introduced Pacific oyster Crassostrea gigas in continental NW European estuaries. Journal of Sea Research, 64 (3), 145-165. DOI https://doi.org/10.1016/j.seares.2010.02.004
Troost, K., van der Meer, J. & van Stralen, M., 2022. The longevity of subtidal mussel beds in the Dutch Wadden Sea. Journal of Sea Research, 181. DOI https://doi.org/10.1016/j.seares.2022.102174
Tsuchiya, M., 1983. Mass mortality in a population of the mussel Mytilus edulis L. Caused by high temperature on rocky shores. Journal of Experimental Marine Biology and Ecology 66: 101-11
Vadas, R.L. & Elner, R.W., 1992. Plant-animal interactions in the north-west Atlantic. In Plant-animal interactions in the marine benthos, (ed. D.M. John, S.J. Hawkins & J.H. Price), 33-60. Oxford: Clarendon Press. [Systematics Association Special Volume, no. 46].
Vadas, R.L., Johnson, S. & Norton, T.A., 1992. Recruitment and mortality of early post-settlement stages of benthic algae. British Phycological Journal, 27, 331-351.
Vajedsamiei, J., Wahl, M., Schmidt, A. L., Yazdanpanahan, M. & Pansch, C., 2021. The higher the needs, the lower the tolerance: Extreme events may select ectotherm recruits with lower metabolic demand and heat sensitivity. Frontiers in Marine Science, 8. DOI https://doi.org/10.3389/fmars.2021.660427
Vajedsamiei, J., Warlo, N., Meier, H. E. M. & Melzner, F., 2024. Predicting key ectotherm population mortality in response to dynamic marine heatwaves: A Bayesian-enhanced thermal tolerance landscape approach. Functional Ecology, 38 (9), 1875–1887. DOI https://doi.org/10.1111/1365-2435.14620
Valdizan, A., Beninger, P. G., Decottignies, P., Chantrel, M. & Cognie, B., 2011. Evidence that rising coastal seawater temperatures increase reproductive output of the invasive gastropod Crepidula fornicata. Marine Ecology Progress Series, 438, 153-165. DOI https://doi.org/10.3354/meps09281
Valentine, P.C., Carman, M.R., Blackwood, D.S. & Heffron, E.J., 2007a. Ecological observations on the colonial ascidian Didemnum sp. in a New England tide pool habitat. Journal of Experimental Marine Biology and Ecology, 342 (1), 109-121. DOI https://doi.org/10.1016/j.jembe.2006.10.021
Valentine, P.C., Collie, J.S., Reid, R.N., Asch, R.G., Guida, V.G. & Blackwood, D.S., 2007b. The occurrence of the colonial ascidian Didemnum sp. on Georges Bank gravel habitat — Ecological observations and potential effects on groundfish and scallop fisheries. Journal of Experimental Marine Biology and Ecology, 342 (1), 179-181. DOI https://doi.org/10.1016/j.jembe.2006.10.038
Valero, M., Destombe, C., Mauger, S., Ribout, C., Engel, C.R., Daguin-Thiebaut, C. & Tellier, F., 2011. Using genetic tools for sustainable management of kelps: a literature review and the example of Laminaria digitata. CBM-Cahiers de Biologie Marine, 52 (4), 467.
Van den Hoek, C., 1982. The distribution of benthic marine algae in relation to the temperature regulation of their life histories. Biological Journal of the Linnean Society, 18, 81-144.
Vaz-Pinto, F., Rodil, I.F., Mineur, F., Olabarria, C. & Arenas, F., 2014. Understanding biological invasions by seaweeds. In Pereira, L. & Neto, J.M. (eds.). Marine algae: biodiversity, taxonomy, environmental assessment and biotechnology. Boca Raton, Florida: CRC Press, pp. 140-177.
Vercaemer, B., Sephton, D., Clément, P., Harman, A., Stewart-Clark, S. & DiBacco, C., 2015. Distribution of the non-indigenous colonial ascidian Didemnum vexillum (Kott, 2002) in the Bay of Fundy and on offshore banks, eastern Canada. Management of Biological Invasions, 6, 385-394. DOI https://doi.org/10.3391/mbi.2015.6.4.07
Viejo, R.M., Arrontes, J. & Andrew, N.L., 1995. An Experimental Evaluation of the Effect of Wave Action on the Distribution of Sargassum muticum in Northern Spain. , 38 (1-6), 437-442. DOI https://doi.org/10.1515/botm.1995.38.1-6.437
Voet, H.E.E., Van Colen, C. & Vanaverbeke, J., 2022. Climate change effects on the ecophysiology and ecological functioning of an offshore wind farm artificial hard substrate community. Science of the Total Environment, 810. DOI https://doi.org/10.1016/j.scitotenv.2021.152194
Vost, L.M., 1983. The influence of Echinus esculentus grazing on subtidal algal communities. British Phycological Journal, 18, 211.
Wale, M.A., Briers, R.A., Hartl, M.G.J., Bryson, D. & Diele, K., 2019. From DNA to ecological performance: Effects of anthropogenic noise on a reef-building mussel. Science of The Total Environment, 689, 126–132. DOI https://doi.org/10.1016/j.scitotenv.2019.06.380
Wang, G., Shuai, L., Li, Y., Lin, W., Zhao, X. & Duan, D., 2008. Phylogenetic analysis of epiphytic marine bacteria on Hole-Rotten diseased sporophytes of Laminaria japonica. Journal of applied phycology, 20 (4), 403-409.
Wang, H.R., Tang, X.X., Chen, J., Shang, S., Zhu, M.L., Liang, S. & Zang, Y., 2021. Comparative studies on the response of Zostera marina leaves and roots to ammonium stress and effects on nitrogen metabolism. Aquatic Toxicology, 240. DOI https://doi.org/10.1016/j.aquatox.2021.105965
Wang, S.V., Ellrich, J.A., Beermann, J., Pogoda, B. & Boersma, M., 2024. Musseling through: Mytilus byssal thread production is unaffected by continuous noise. Marine Environmental Research, 200. DOI https://doi.org/10.1016/j.marenvres.2024.106661
Wang, W. & Widdows, J., 1991. Physiological responses of mussel larvae Mytilus edulis to environmental hypoxia and anoxia. Marine Ecology Progress Series, 70, 223-36
Weldrick, C.K. & Jelinski, D.E., 2016. Resource subsidies from multi-trophic aquaculture affect isotopic niche width in wild blue mussels (Mytilus edulis). Journal of Marine Systems, 157, 118–123. DOI https://doi.org/10.1016/j.jmarsys.2016.01.001
Wells, H.W. & Gray, I.E., 1960. The Seasonal Occurrence of Mytilus edulis on the Carolina Coast as a Result of Transport around Cape Hatteras. Biological Bulletin, 119 (3), 550-559. DOI https://doi.org/10.2307/1539267
Werner, A. & Kraan, S., 2004. Review of the potential mechanisation of kelp harvesting in Ireland. Marine Environment and Health Series, (No. 17).
Westerbom, M. & Jattu, S., 2006. Effects of wave exposure on the sublittoral distribution of blue mussels Mytilus edulis in a heterogeneous archipelago. Marine Ecology Progress Series, 306, 191-200.
Whitehouse, J., Coughlan, J., Lewis, B., Travade, F. & Britain, G., 1985. The control of biofouling in marine and estuarine power stations: a collaborative research working group report for use by station designers and station managers. Central Electricity Generating Board
Whittick, A., 1983. Spatial and temporal distributions of dominant epiphytes on the stipes of Laminaria hyperborea (Gunn.) Fosl. (Phaeophyta: Laminariales) in S.E. Scotland. Journal of Experimental Marine Biology and Ecology, 73, 1-10.
Widdows J., Lucas J.S., Brinsley M.D., Salkeld P.N. & Staff F.J., 2002. Investigation of the effects of current velocity on mussel feeding and mussel bed stability using an annular flume. Helgoland Marine Research, 56(1), 3-12.
Widdows, J., Bayne, B.L., Livingstone, D.R., Newell, R.I.E. & Donkin, P., 1979. Physiological and biochemical responses of bivalve molluscs to exposure to air. Comparative Biochemistry and Physiology, 62A, 301-308.
Widdows, J., Moore, M., Lowe, D. & Salkeld, P., 1979b. Some effects of a dinoflagellate bloom (Gyrodinium aureolum) on the mussel, Mytilus edulis. Journal of the Marine Biological Association of the United Kingdom, 59 (2), 522-524.
- Wiens, J.J., 2016. Climate-Related Local Extinctions Are Already Widespread among Plant and Animal Species. PLOS Biology, 14 (12), e2001104. DOI https://doi.org/10.1371/journal.pbio.2001104
Williams, R.J., 1970. Freezing tolerance in Mytilus edulis. Comparative Biochemistry and Physiology, 35, 145-161
Winter, J., 1972. Long-term laboratory experiments on the influence of ferric hydroxide flakes on the filter-feeding behaviour, growth, iron content and mortality in Mytilus edulis L. Marine pollution and sea life. (ed. Ruvio, M.) London, England, pp. 392-396.
Witman, J.D. & Suchanek, T.H., 1984. Mussels in flow: drag and dislodgement by epizoans. Marine Ecology Progress Series, 16 (3), 259-268.
Wood, L. E., Silva, T. A. M., Heal, R., Kennerley, A., Stebbing, P., Fernand, L. & Tidbury, H. J., 2021. Unaided dispersal risk of Magallana gigas into and around the UK: combining particle tracking modelling and environmental suitability scoring. Biological Invasions, 23 (6), 1719-1738. DOI https://doi.org/10.1007/s10530-021-02467-x
Wotton, D.M., O'Brien, C., Stuart, M.D. & Fergus, D.J., 2004. Eradication success down under: heat treatment of a sunken trawler to kill the invasive seaweed Undaria pinnatifida. Marine Pollution Bulletin, 49 (9), 844-849.
Yesson, C., Bush, L.E., Davies, A.J., Maggs, C.A. & Brodie, J., 2015b. Large brown seaweeds of the British Isles: Evidence of changes in abundance over four decades. Estuarine, Coastal and Shelf Science, 155, 167-175.
Yonemitsu, M. A., Giersch, R. M., Polo-Prieto, M., Hammel, M., Simon, A., Cremonte, F., Avilés, F. T., Merino-Veliz, N., Burioli, E. A. V. & Muttray, A. F., 2019. A single clonal lineage of transmissible cancer identified in two marine mussel species in South America and Europe. Elife, 8, e47788. DOI https://doi.org/10.7554/eLife.47788
Young, G.A., 1985. Byssus thread formation by the mussel Mytilus edulis: effects of environmental factors. Marine Ecology Progress Series, 24, 261-271.
Zacher, K., Bernard, M., Bartsch, I. & Wiencke, C., 2016. Survival of early life history stages of Arctic kelps (Kongsfjorden, Svalbard) under multifactorial global change scenarios. Polar Biology, 39 (11), 2009–2020. DOI https://doi.org/10.1007/s00300-016-1906-1
Zacher, K., Bernard, M., Daniel Moreno, A. & Bartsch, I., 2019. Temperature mediates the outcome of species interactions in early life-history stages of two sympatric kelp species. Marine Biology, 166 (12), 161. DOI http://doi.org/10.1007/s00227-019-3600-7
Zandee, D.I., Holwerda, D.A., Kluytmans, J.H. & De Zwaan, A., 1986. Metabolic adaptations to environmental anoxia in the intertidal bivalve mollusc Mytilus edulis L. Netherlands Journal of Zoology, 36(3), 322-343.
Zardi, G. I., Monsinjon, J. R., Seuront, L., Spilmont, N., McQuaid, C. D. & Nicastro, K. R., 2024. Symbiotic endolithic microbes reduce host vulnerability to an unprecedented heatwave. Marine Environmental Research, 199. DOI https://doi.org/10.1016/j.marenvres.2024.106622
Zippay, M.L. & Helmuth, B., 2012. Effects of temperature change on mussel, Mytilus. Integrative Zoology, 7 (3), 312-327. DOI https://doi.org/10.1111/j.1749-4877.2012.00310.x
de Zwaan, A. & Mathieu, M., 1992. Cellular biochemistry and endocrinology. In The mussel Mytilus: ecology, physiology, genetics and culture, (ed. E.M. Gosling), pp. 223-307. Amsterdam: Elsevier Science Publ. [Developments in Aquaculture and Fisheries Science, no. 25]
Citation
This review can be cited as:
Last Updated: 18/09/2026
- Dabberlocks